Call or Text 727-513-9780
  • Shopping Cart Shopping Cart
    0Shopping Cart
Pure Tested Peptides | America's most trusted Peptides for sale online
  • Peptides for sale
    • Oral Peptides for sale
      • Peptide Capsules for sale
      • BPC 157 Capsules 1000mcg
      • SLU-PP-332 Capsules | 1000 mcg
      • 5-Amino-1MQ 50mg Capsules
      • Tesofensine 500mcg
    • All Peptides for sale
    • Peptide Sprays
      • BPC 157 Nasal Spray Kit
      • BPC-157 TB500 Nasal Spray Kit
      • Semax Nasal Spray 10mg
      • Selank – Nasal Spray Kit – 10mg
      • Epithalon 50MG Nasal Spray Kit
      • Ipamorelin 10mg Nasal Spray
      • Klow Nasal Spray (BPC-157 + TB-500 + GHK-Cu + KPV) | 80mg
      • Hulk Nasal Spray Tesa / Ipa Blend 6/3 MG
      • Klow Nasal Spray
      • NAD + 500 mg Nasal Spray
      • PT-141 Nasal Spray Kit
    • GHRH Peptides
      • Ipa Peptides
      • CJC-1295 Peptides
        • CJC-1295 with DAC 5 mg
        • CJC-1295 without DAC 5 mg
        • CJC-1295 Ipa 10mg
      • Tesa Peptides
        • Tesa Peptide
        • Tesa 20 mg
    • GHK-Cu Peptides
      • All GHK-Cu Peptides
      • GHK-Cu 100mg
      • KLOW Peptide Blend – Buy KLOW blend online
    • BPC Peptides
      • All BPC Peptides
      • BPC-157
      • BPC-157 TB-500
      • BPC 157 capsules 1000mcg
    • SLU-PP-332 Peptides
      • All SLU-PP-332 Peptides
      • SLU-PP-332 5mg
    • GLP3 Peptides
    • PT-141 Peptides
      • PT-141 Peptides for sale
      • PT-141 10mg
      • PT-141 Nasal Spray
    • CAG Peptides
      • Lipo-C Peptide Blend
      • CAG 5mg
      • CAG 10mg
    • MOTS-C Peptides
      • MOTS-C Peptides for sale
      • MOTS-c peptide
      • MOTS-c 10mg *6 pack*
    • 5 Amino 1MQ Peptides
      • 5 Amino 1MQ Peptides for sale
      • 5-Amino-1MQ 50mg Capsules
      • 5-Amino-1MQ 5mg
    • Epithalon Peptides
      • Epithalon Peptides for sale
      • Epithalon 10mg
      • Epithalon 50mg
  • Shop
    • GLPs
      • 5-Amino-1MQ 50mg Capsules
      • 5-Amino-1MQ 5mg
      • L-Carnitine 500mg/ml
      • Tesofensine 500mcg
      • SLU-PP-332 5mg
      • MOTS-c 10mg *6 pack*
    • Epithalon & BPC Peptides
      • Epithalon 10mg
      • Epithalon 50mg
      • BPC-157
      • BPC 157 capsules 1000mcg
      • BPC-157 TB-500
      • BPC-157 TB500 Nasal Spray Kit
      • BPC 157 Nasal Spray Kit
    • BPC TB-500 & NAD+ Peptides
      • NAD+ 500 mg
      • KLOW Peptide Blend – Buy KLOW blend online
      • GLOW Peptide Blend
      • TB 500 5mg
      • BPC 157 capsules 1000mcg – Supplement
      • BPC 157 Nasal Spray Kit
      • BPC-157
      • BPC-157 TB500 Nasal Spray Kit
      • BPC-157 TB-500
      • BPC 157 capsules 1000mcg
    • LL-37 Peptide
      • LL-37 10 mg
    • MOTS-C & Selank
      • MOTS-c peptide
      • Selank 10mg
    • GHK Peptides
      • GHK-Cu 100mg
      • GLOW Peptide Blend
      • KLOW Peptide Blend – Buy KLOW blend online
  • COAs
  • Wholesale
    • Wholesale Peptides for sale
  • PTP FAQ
  • Affiliates
    • Selank Peptide: Advanced Pharmacological Mechanisms Underlying Its Anxiolytic and Nootropic Effects in Research
      • 5-Amino-1MQ Peptide: Detailed Mechanisms of NNMT Inhibition and Its Impact on Cellular Metabolism Research
        • MOTS-C Peptide: Unraveling Its Role in Mitochondrial Dynamics and Energy Metabolism Research
          • Epithalon Peptide and Telomerase Regulation: Investigating Its Impact on Cellular Senescence and Lifespan Research Models
            • GLP2-T vs GLP2 Tirz Peptide: Understanding the Naming, Mechanistic Nuances, and Research Implications for Gut Health
      • Peptides and Polypeptides in Modern Pharmacology: What Research on Metoprolol, Prednisone, and Amlodipine Reveals
        • Polypeptide Peptides vs NSAIDs: What Naproxen and Diclofenac Teach Tissue-Repair Researchers About BPC‑157 and TB‑500
          • Peptides and Polypeptides in Endocrine Pharmacology: How GLP-1, GLP-2, and GLP-3 Retatrutide Differ From Classic Drugs Like Prednisone and Amlodipine
          • 5‑Amino‑1MQ Peptide and NNMT Inhibition: How It Compares With Statins Like Atorvastatin in Adipose and Lipid Metabolism Research
      • Enclomiphene, Estrogen Receptor Signaling, and Luteinizing Phase Biology: What Hormone Researchers Should Measure
        • Mesenchymal Stem Cells, BPC‑157, and GHK‑Cu: How Tissue Repair Peptides Compare With Classic NSAIDs Like Naproxen in Injury Models
          • Peptide Calculator Use Cases Beyond Growth Hormone: Working Through GLP‑3 Retatrutide, MOTS‑c, and BPC‑157 Research Dosing
        • Polypeptide Peptides in Endocrine and Metabolic Pharmacology: Lessons From Amlodipine, Prednisone, and Metoprolol
        • Peptides Calculator for Advanced Blends: Worked Examples for Tesamorelin, CJC‑1295, and Ipamorelin Stacks
          • Peptides and Polypeptides in Human Physiology: How Molecular Size Shapes Research Applications
            • Selank Peptide: Advanced Pharmacological Mechanisms Underlying Its Anxiolytic and Nootropic Effects in Research
          • 5-Amino-1MQ Peptide: Detailed Mechanisms of NNMT Inhibition and Its Impact on Cellular Metabolism Research
            • MOTS-C Peptide: Unraveling Its Role in Mitochondrial Dynamics and Energy Metabolism Research
              • Epithalon Peptide and Telomerase Regulation: Investigating Its Impact on Cellular Senescence and Lifespan Research Models
                • GLP2-T vs GLP2 Tirz Peptide: Understanding the Naming, Mechanistic Nuances, and Research Implications for Gut Health
                  • Peptides and Polypeptides in Endocrine Pharmacology: How GLP-1, GLP-2, and GLP-3 Retatrutide Differ From Classic Drugs Like Prednisone and Amlodipine
                    • Polypeptide Peptides vs NSAIDs: What Naproxen and Diclofenac Teach Tissue-Repair Researchers About BPC‑157 and TB‑500
                      • Peptides and Polypeptides in Modern Pharmacology: What Research on Metoprolol, Prednisone, and Amlodipine Reveals
                        • 5‑Amino‑1MQ Peptide and NNMT Inhibition: How It Compares With Statins Like Atorvastatin in Adipose and Lipid Metabolism Research
                        • Enclomiphene, Estrogen Receptor Signaling, and Luteinizing Phase Biology: What Hormone Researchers Should Measure
                        • Mesenchymal Stem Cells, BPC‑157, and GHK‑Cu: How Tissue Repair Peptides Compare With Classic NSAIDs Like Naproxen in Injury Models
                        • Peptide Calculator Use Cases Beyond Growth Hormone: Working Through GLP‑3 Retatrutide, MOTS‑c, and BPC‑157 Research Dosing
                        • Polypeptide Peptides in Endocrine and Metabolic Pharmacology: Lessons From Amlodipine, Prednisone, and Metoprolol
                        • Peptides Calculator for Advanced Blends: Worked Examples for Tesamorelin, CJC‑1295, and Ipamorelin Stacks
                        • Peptides and Polypeptides in Human Physiology: How Molecular Size Shapes Research Applications
                        • Selank Peptide: Advanced Pharmacological Mechanisms Underlying Its Anxiolytic and Nootropic Effects in Research
                        • MOTS-C Peptide: Unraveling Its Role in Mitochondrial Dynamics and Energy Metabolism Research
                        • Peptides and Polypeptides in Modern Pharmacology: What Research on Metoprolol, Prednisone, and Amlodipine Reveals
                        • Peptides and Polypeptides in Endocrine Pharmacology: How GLP-1, GLP-2, and GLP-3 Retatrutide Differ From Classic Drugs Like Prednisone and Amlodipine
                        • 5-Amino-1MQ Peptide: Detailed Mechanisms of NNMT Inhibition and Its Impact on Cellular Metabolism Research
                        • Mesenchymal Stem Cells, BPC‑157, and GHK‑Cu: How Tissue Repair Peptides Compare With Classic NSAIDs Like Naproxen in Injury Models
                        • Peptide Calculator Use Cases Beyond Growth Hormone: Working Through GLP‑3 Retatrutide, MOTS‑c, and BPC‑157 Research Dosing
                        • GLP2-T vs GLP2 Tirz Peptide: Understanding the Naming, Mechanistic Nuances, and Research Implications for Gut Health
                        • Polypeptide Peptides in Endocrine and Metabolic Pharmacology: Lessons From Amlodipine, Prednisone, and Metoprolol
                        • Polypeptide Peptides vs NSAIDs: What Naproxen and Diclofenac Teach Tissue-Repair Researchers About BPC‑157 and TB‑500
                        • Peptides and Polypeptides in Human Physiology: How Molecular Size Shapes Research Applications
                        • Peptides Calculator for Advanced Blends: Worked Examples for Tesamorelin, CJC‑1295, and Ipamorelin Stacks
                        • 5‑Amino‑1MQ Peptide and NNMT Inhibition: How It Compares With Statins Like Atorvastatin in Adipose and Lipid Metabolism Research
                        • Enclomiphene, Estrogen Receptor Signaling, and Luteinizing Phase Biology: What Hormone Researchers Should Measure
                        • Epithalon Peptide and Telomerase Regulation: Investigating Its Impact on Cellular Senescence and Lifespan Research Models
                        • Best research protocol Klow blend
                        • best time to take BPC-157
                        • best time to take DSIP (Delta Sleep Inducing Peptide)
                        • best time to take CJC-1295
                        • best time to take AOD-9604
                        • best time to take Follistatin 344
                        • best time to take Ipamorelin
                        • best time to take MK-677 (Ibutamoren)
                        • best time to take Ligandrol (LGD-4033) — research compound
                        • best time to take Ostarine (MK-2866) — research compound
                        • best time to take GHK-CU
                        • best time to take TB-500
                        • best time to take MOTS-c
                        • best time to take Semax
                        • best time to take RAD-140 (Testolone) — research compound
                        • best time to take Thymosin Alpha-1
                        • best time to take PEG-MGF
                        • Biolife Plasma, Octapharma Plasma, and Research Peptides: How Plasma Donation Labs Differ From Peptide Suppliers
                        • best time to take YK-11 — research compound
                        • best time to take PT-141 (Bremelanotide)
                        • Best research protocol Klow blend
                        • 5-Amino-1MQ and MOTS-C Synergy: Metabolic Signaling, Mitochondria, and Research Design
                        • BPC-157 and TB-500: Investigating Their Combined Effects on Angiogenesis and Cellular Migration in Tissue Repair Models
                        • BPC-157 Peptide: Gut Barrier Function, Inflammation, and Tissue-Recovery Research
                        • 5‑Amino‑1MQ and MOTS‑c Synergy in Metabolic Research: Designing NNMT and Mitochondrial Biogenesis Stacks
                        • CJC-1295 with DAC vs. Without DAC: Half-Life, Release Kinetics, and Research Implications
                        • CJC‑1295 with DAC vs. Without DAC: Expanding on Half‑Life Differences Using Tesamorelin and Ipamorelin Blend Case Studies
                        • Collagen Biology and Copper‑Binding Peptides: How GHK‑Cu, Glow Blend, and Klow Blend Interact with Skin and Connective Tissue
                        • Collagen Biology and Regenerative Peptides: How GHK‑Cu, Glow Blend, and Klow Blend Affect Extracellular Matrix Research
                    • DNA, Telomeres, and Longevity Peptides: Positioning Epithalon and MOTS‑c in Genetic Aging Research
                      • Enclomiphene Citrate: serm Mechanism, Testosterone Research, and Stack Compatibility
                        • Enclomiphene vs Enclomiphene Citrate: Formulation, Bioavailability, and Research Distinctions
                        • Epithalon Peptide Research: Telomerase Activation, Aging, and Pineal Gland Function
                        • Estrogen Receptor Signaling and Enclomiphene: How Selective Modulators Compare with Classic Polypeptide Hormones
                        • GHK-Cu Peptide: Advanced Mechanisms in Extracellular Matrix Remodeling and Wound Healing Research
                        • GHK-Cu Peptide: Collagen Synthesis, Wound Repair, and Skin-Barrier Research Models
                        • GLP-1 vs GLP-3 vs GLP-2: Peptide Classification and Research Applications
                        • GLP-2 Peptide Research Guide: Gut Barrier Function, Nutrient Absorption, and Intestinal Recovery Models
                        • GLP-3 Retatrutide vs. GLP-1 Drugs: What Triple-Agonist Biology Changes in Research Models
                        • Ipamorelin and Tesamorelin Combination: Synergistic GH Secretagogue Research and Dosing Protocols
                        • GLP2 Tirz Peptide: What It Is, Why the Name Exists, and How Researchers Should Interpret It
                        • Klow Blend Peptide Nasal Spray: What the Formulation Is Trying to Do in Cognitive Research
                        • Mitochondria, NNMT Inhibition, and Peptide Modulators: Where MOTS‑c and 5‑Amino‑1MQ Fit in Cellular Energy Research
                        • MOTS-c Peptide: Mitochondrial Function, Energy Metabolism, and What Researchers Measure
                        • MOTS-c vs. 5-Amino-1MQ: Which Metabolic Research Questions Each Compound Actually Answers
                        • Nasal Spray Peptides: Bioavailability, Administration, and Semax/Selank Research Applications
                        • PT-141 Peptide Research: Mechanism of Action and Melanocortin Receptor Signaling
                        • Retatrutide for Research: Mechanism, Structure, and GLP-1/GLP-3 Dual Action
                        • Retatrutide for Obesity and Type 2 Diabetes: What the Latest Trial Data Suggest
                        • Tesofensine Peptide Research: Mechanism, Appetite Suppression, and Neuropeptide Y Pathways
  • Contact
    • Contact Customer Service
    • Text Customer Support
  • About US
  • Shop all peptides
  • Affiliate Program
    • Affiliate Signup
  • Login / Register Login / Register Page Link Login / Register Page Link
  • Click to open the search input field Click to open the search input field Search
  • Menu Menu

Tag Archive for: nnmt inhibitor

MOTS-c and 5-Amino-1MQ in Skeletal-Muscle Models: Mitochondrial Flux, NNMT, and Insulin-Signaling Controls

MOTS-c and 5-Amino-1MQ in Skeletal-Muscle Models: Mitochondrial Flux, NNMT, and Insulin-Signaling Controls

October 20, 2026/0 Comments/in Uncategorized/by

Skeletal-muscle MOTS-c levels rise approximately 11.9-fold in young men following a single acute exercise session, a magnitude that places this mitochondrial-derived peptide in a category of its own among exercise-induced metabolic signals. Yet combining that finding with data on 5-Amino-1MQ, a selective NNMT inhibitor, requires careful separation of muscle-specific endpoints from whole-body metabolic readouts. This article unpacks how MOTS-c and 5-Amino-1MQ in skeletal-muscle models operate through distinct but potentially complementary mechanisms, covering mitochondrial flux, NNMT biology, and insulin-signaling controls, while keeping tissue-specific effects clearly distinguished.

Key Takeaways

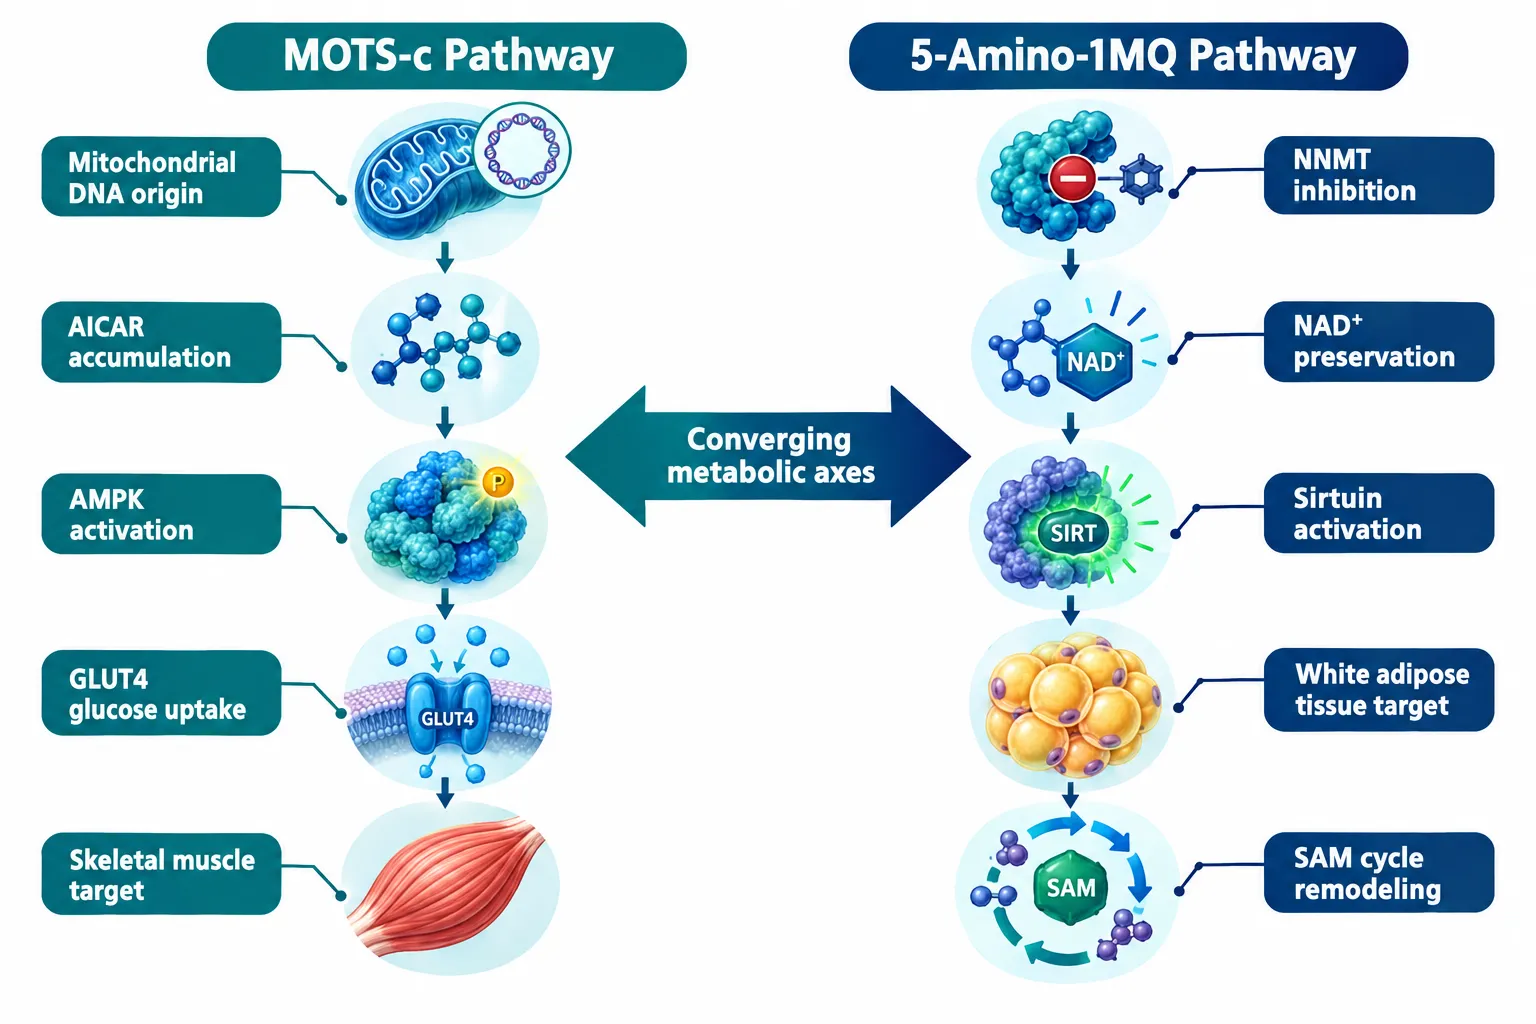
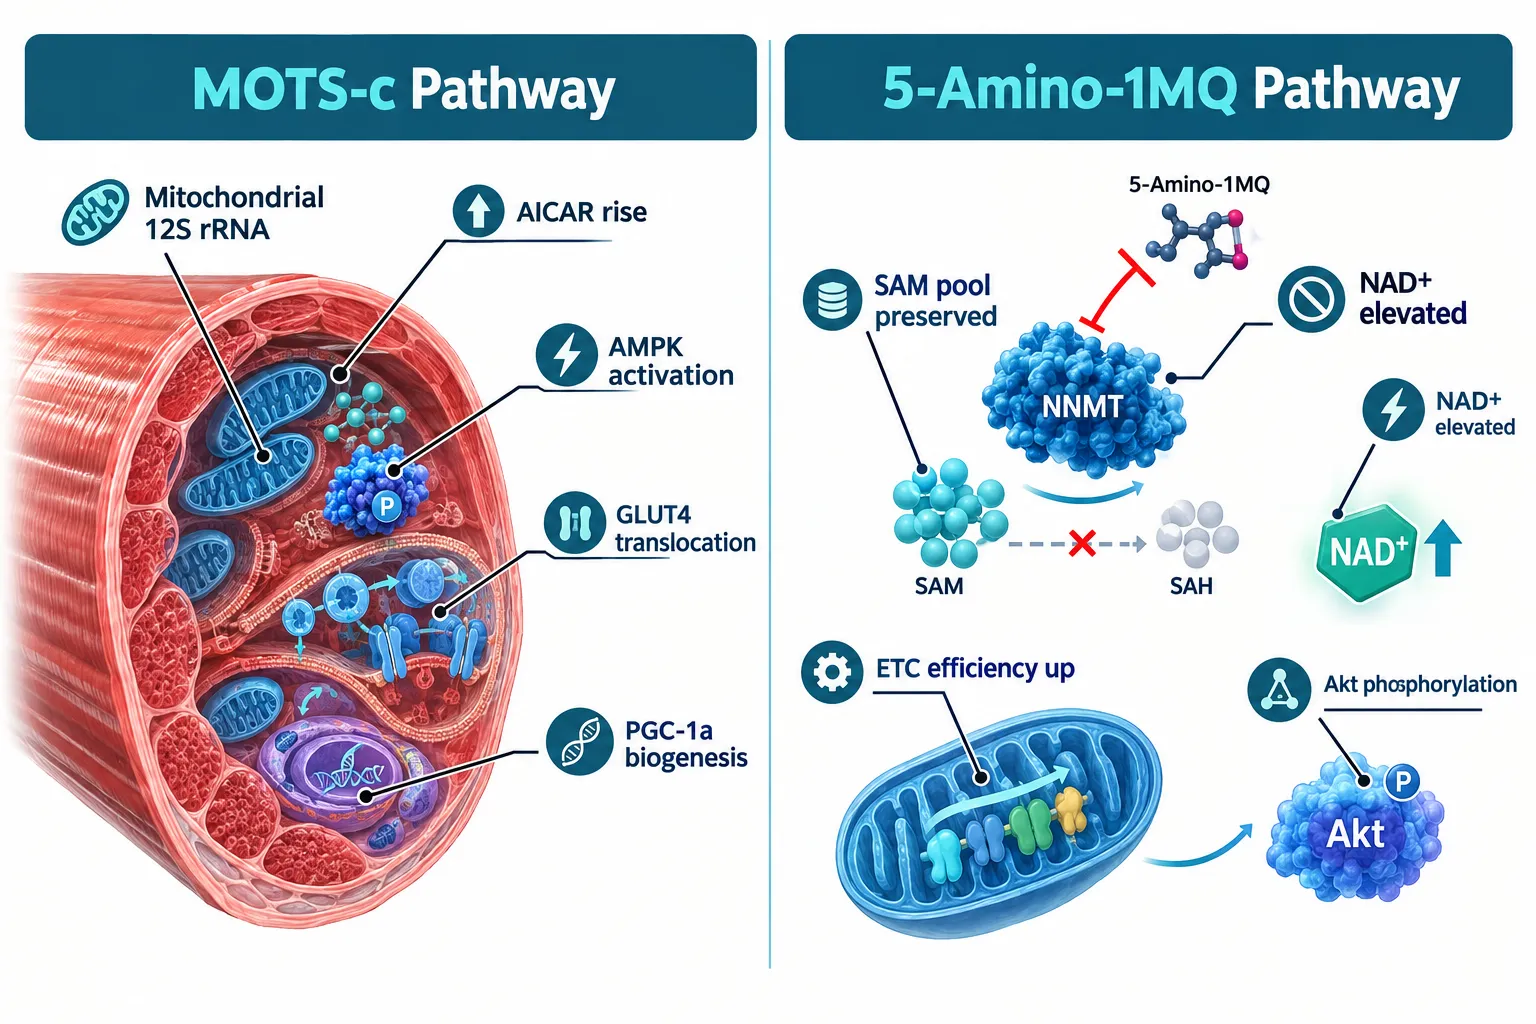
  • MOTS-c is a 16-amino-acid mitochondrial-derived peptide that activates AMPK through the folate-AICAR axis, driving GLUT4 translocation and mitochondrial biogenesis primarily in muscle fibers.
  • 5-Amino-1MQ inhibits NNMT with an IC50 of approximately 1.2 µM, raising intracellular NAD+ and SAM levels to support mitochondrial electron-transport efficiency, mainly through an indirect redox mechanism.
  • These compounds operate on different primary compartments: MOTS-c on muscle and liver via AMPK/PGC-1a; 5-Amino-1MQ on adipose and aged muscle stem cells via the NNMT/NAD+ axis.
  • Conflating systemic metabolic improvements with direct muscle-fiber effects is a common error; glucose uptake, respiration, methylation markers, and cytotoxicity must each be measured independently.
  • Both compounds remain research-only tools in 2026, with no approved therapeutic indications or large controlled human trials.

How MOTS-c Drives Mitochondrial Flux in Muscle Fibers
How MOTS-c Drives Mitochondrial Flux in Muscle Fibers

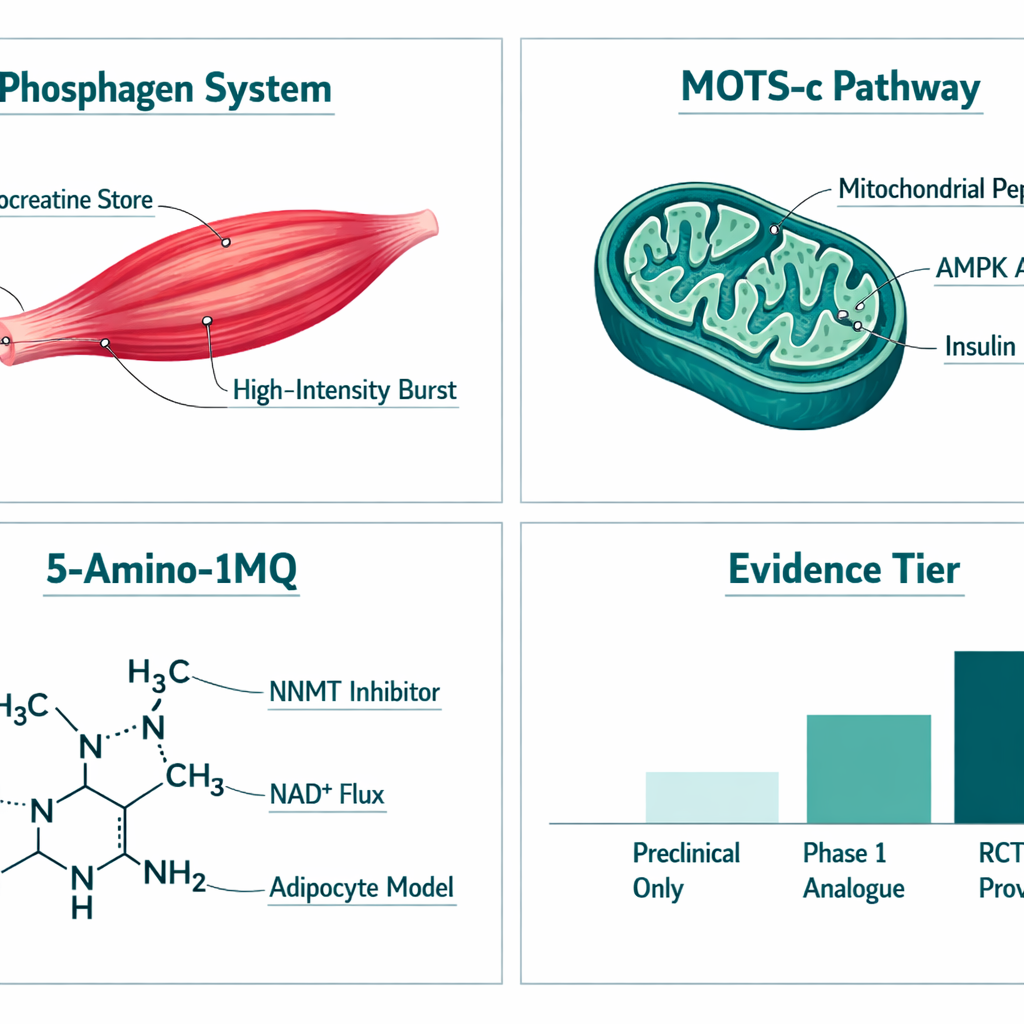
MOTS-c is encoded within the mitochondrial 12S rRNA gene and released as a 16-amino-acid peptide that translocates to the nucleus under metabolic stress. Its primary signaling route runs through the folate cycle: MOTS-c disrupts one-carbon metabolism, causing AICAR (an AMPK activator) to accumulate. The resulting AMPK activation triggers downstream effects that are well-documented in skeletal-muscle models.

Muscle-specific readouts linked to MOTS-c include:

  • Increased mitochondrial oxygen consumption and bioenergetic efficiency
  • Greater fatty-acid oxidation relative to glucose oxidation
  • Reduced mitochondrial reactive oxygen species (ROS) emission
  • Lower oxidative protein damage markers within muscle tissue
  • GLUT4 vesicle translocation to the sarcolemma, enhancing glucose uptake

Crucially, PGC-1a upregulation downstream of AMPK links MOTS-c directly to mitochondrial biogenesis, new mitochondria, not just better-functioning existing ones. This explains why researchers describe the peptide as an exercise-mimetic rather than simply an insulin sensitizer.

For broader context on mitochondrial peptide research themes, the MOTS-c and elamipretide comparison resource offers useful parallel reading, as does the SS-31 mitochondrial research themes overview.

One important distinction worth emphasizing: human evidence is currently correlational. Endurance training increases both skeletal-muscle mitochondrial respiration and endogenous MOTS-c secretion together, but exogenous MOTS-c administration has not yet been shown to fully reproduce exercise-derived benefits in controlled human trials. Treating the correlation as proof of causation in muscle models is a methodological hazard researchers should actively avoid.


5-Amino-1MQ, NNMT Inhibition, and the NAD+ Axis: Separating Muscle from Adipose Effects
5-Amino-1MQ, NNMT Inhibition, and the NAD+ Axis: Separating Muscle from Adipose Effects

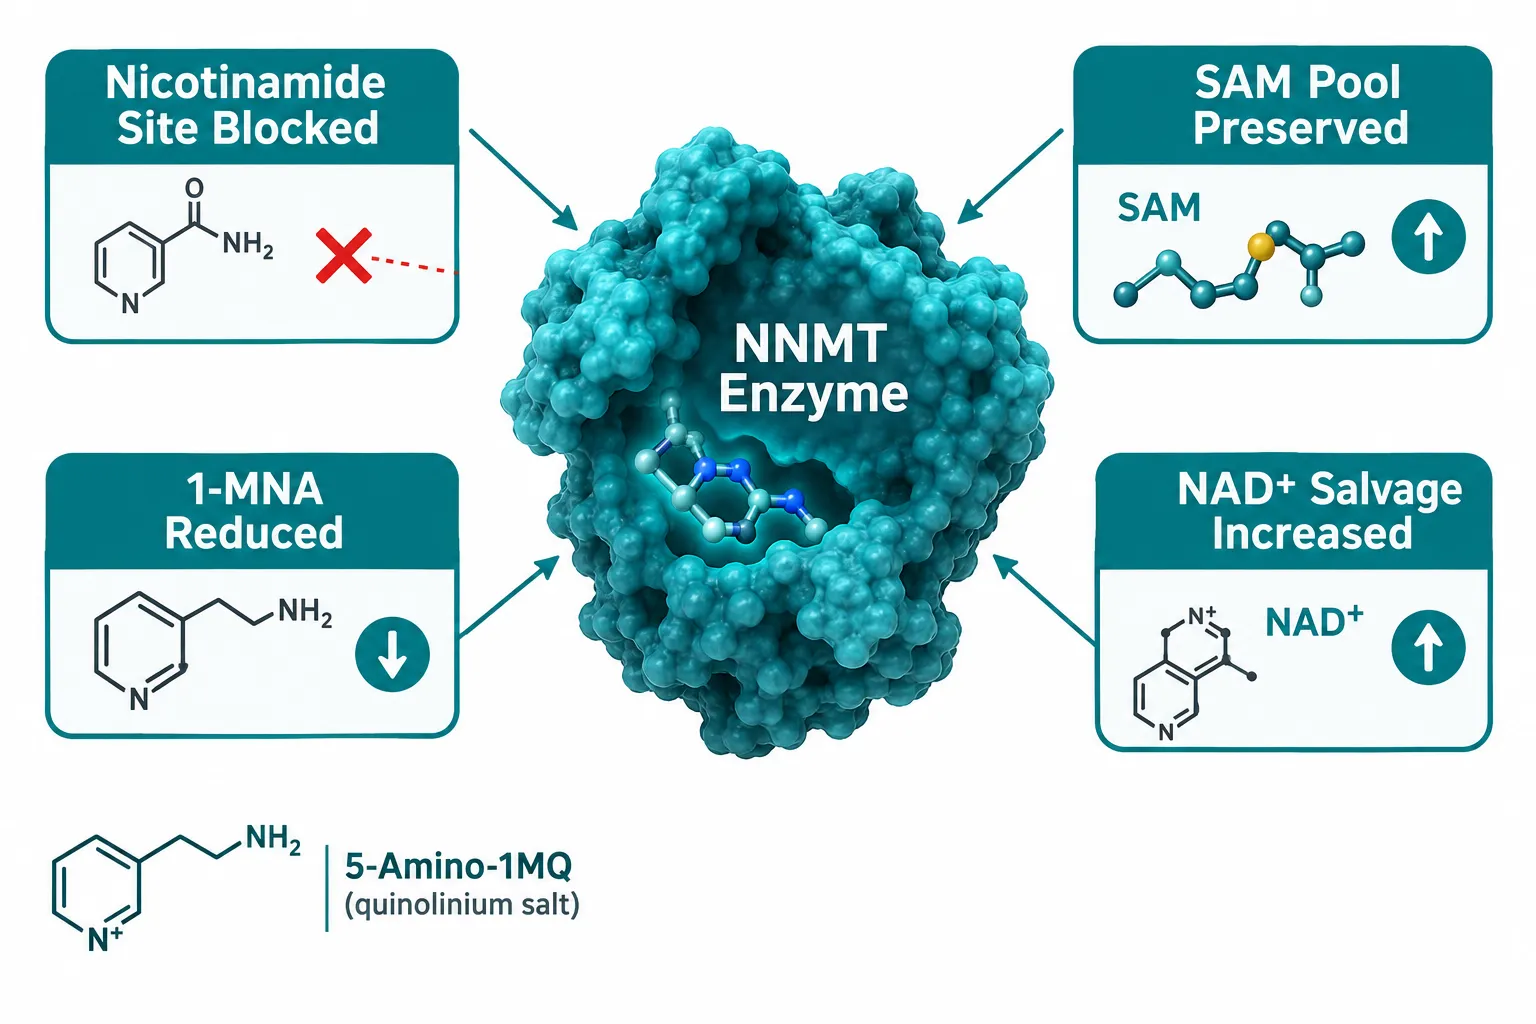
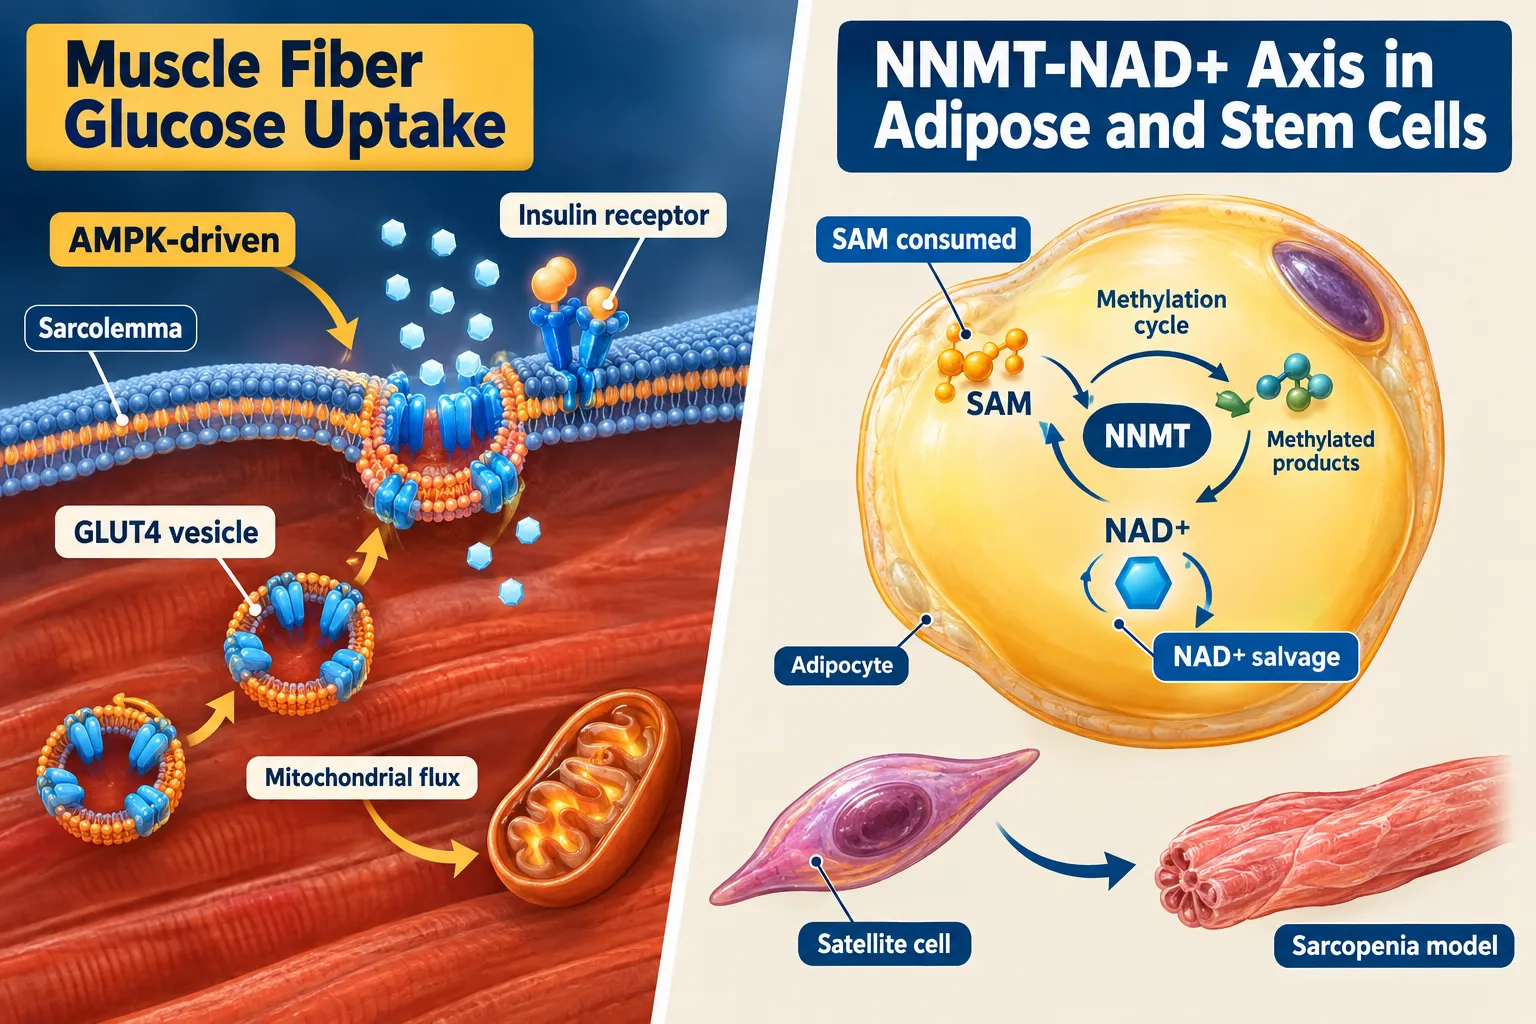
Nicotinamide N-methyltransferase (NNMT) consumes S-adenosylmethionine (SAM) while converting nicotinamide to 1-methylnicotinamide. When NNMT is overactive, a feature of obese adipose tissue, it depletes both SAM and NAD+ precursors, suppressing mitochondrial electron-transport-chain (ETC) efficiency and cellular energy expenditure. 5-Amino-1MQ blocks NNMT selectively, sparing related SAM-dependent methyltransferases and NAD+ salvage enzymes.

What inhibiting NNMT does at the cellular level:

Readout Direction with 5-Amino-1MQ
Intracellular NAD+ Increases
SAM pool Preserved / elevated
ETC efficiency Improved (indirect)
Akt phosphorylation (insulin-stimulated) Enhanced in adipocytes
Glucose uptake (adipocytes) Improved

The IC50 for NNMT inhibition sits at approximately 1.2 ± 0.1 µM, a potency figure that grounds its use in in vitro and preclinical muscle and adipose models.

A common error in summarizing 5-Amino-1MQ data is treating adipocyte insulin-signaling improvements as direct skeletal-muscle fiber effects. NNMT knockdown and pharmacologic inhibition consistently enhance insulin-stimulated Akt phosphorylation and glucose uptake in adipocytes, but this does not automatically translate to the same magnitude of effect in differentiated muscle fibers. The primary tissue target is white adipose, with secondary applications in aged muscle stem cells, specifically satellite-cell biology in sarcopenia models, where NAD+ preservation supports regenerative capacity.

For those exploring mitochondrial-targeted compounds alongside NNMT inhibitors, the MOTS-c peptide research page and the SS-31 peptide category provide relevant reference material on complementary mitochondrial tools.


Integrating Both Compounds: Pathway Complementarity and Experimental Design Considerations
Integrating Both Compounds: Pathway Complementarity and Experimental Design Considerations

The conceptual appeal of studying MOTS-c and 5-Amino-1MQ in skeletal-muscle models together rests on pathway complementarity. MOTS-c drives AMPK-mediated mitochondrial biogenesis and GLUT4-dependent glucose uptake in muscle fibers. 5-Amino-1MQ modulates the NNMT/NAD+/SAM axis, primarily in adipose and aged muscle stem cells, with indirect effects on ETC redox balance. Combining AMPK activation with NNMT inhibition could theoretically broaden coverage of mitochondrial flux and insulin-signaling control points across both muscle and adipose compartments.

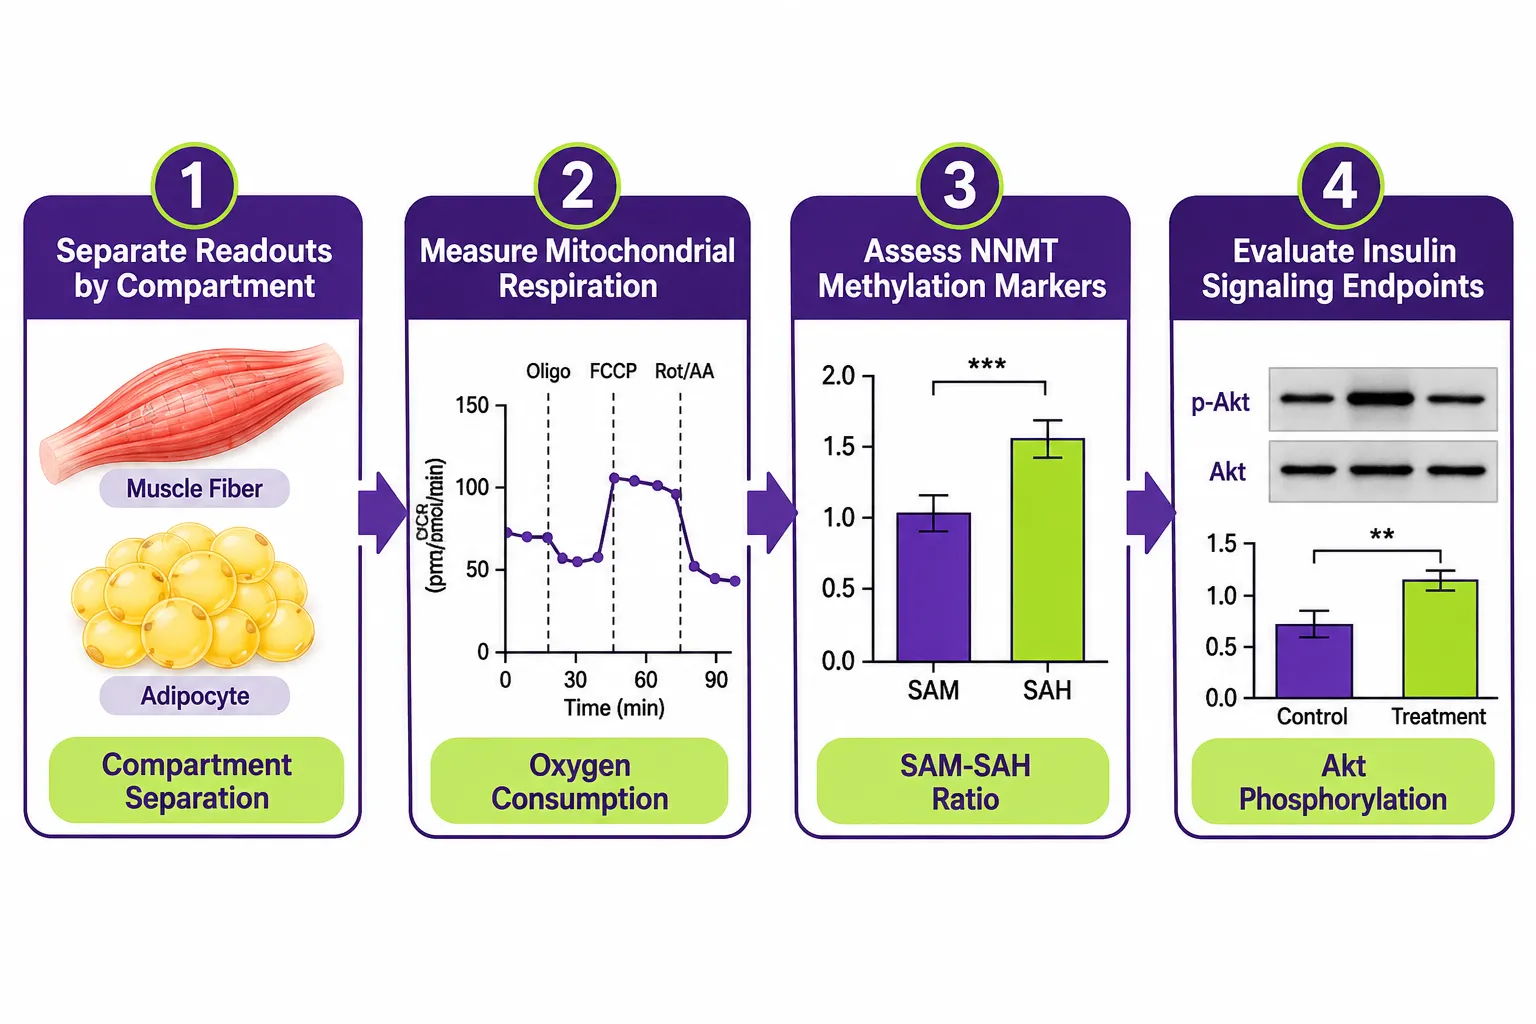
However, rigorous experimental design must separate four distinct readout categories:

  1. Muscle-specific glucose uptake, measure GLUT4 translocation and 2-deoxyglucose uptake directly in myotubes, not inferred from systemic glycemia.
  2. Mitochondrial respiration, use Seahorse XF or equivalent to assess oxygen consumption rate (OCR) and extracellular acidification rate (ECAR) in isolated muscle preparations.
  3. Methylation-related readouts, quantify SAM/SAH ratios and 1-methylnicotinamide levels as direct NNMT-activity markers, separating them from general metabolic changes.
  4. Cytotoxicity screening, run parallel LDH release or MTT assays at experimental concentrations to confirm effects are not confounded by cellular stress or death.

Treating systemic improvements in obese animal models as evidence of direct muscle-fiber effects for either compound is a recurring limitation in preclinical literature. Tissue-specific protein analysis, p-Akt/Akt in muscle versus adipose fractions, muscle-specific PGC-1a protein, and AMPK phosphorylation status, should be reported separately for each compartment.

"Combining AMPK activation with NNMT inhibition could yield broader modulation of mitochondrial flux and insulin signaling, but only if tissue-specific endpoints are tracked independently."

As of 2026, MOTS-c is more directly relevant to exercise-mimetic and mitochondrial-flux research in muscle fibers, while 5-Amino-1MQ is more directly relevant to aged muscle stem-cell biology and adipose energy expenditure. Future research directions likely include MOTS-c analogs in age-related metabolic decline and type 2 diabetes, and NNMT inhibitors in muscle-regeneration indications, but these remain speculative frameworks, not established clinical pipelines.

For researchers interested in the broader mitochondrial peptide landscape, the SS-31 mitochondrial research resource and the SS-31 kidney health research page illustrate how tissue-specific readouts are handled in adjacent mitochondrial-peptide programs.


Conclusion

The intersection of MOTS-c and 5-Amino-1MQ in skeletal-muscle models: mitochondrial flux, NNMT, and insulin-signaling controls is a productive but precision-demanding research space. The actionable steps for investigators in 2026 are clear:

  • Distinguish muscle-fiber endpoints from adipose and systemic endpoints in every experimental design.
  • Measure NNMT activity and NAD+/SAM pools as primary readouts for 5-Amino-1MQ, not just downstream glucose tolerance.
  • Use direct mitochondrial respiration assays rather than proxy metabolic markers for MOTS-c.
  • Include cytotoxicity controls at all tested concentrations.
  • Avoid extrapolating correlational human exercise data to exogenous MOTS-c efficacy claims.

Both compounds are research-only tools. Investigators should source materials from suppliers that provide third-party purity verification, such as lab-tested peptides with documented quality control, to ensure that experimental variability reflects biology rather than compound quality.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/mots-c-and-5-amino-1mq-in-skeletal-muscle-models-mitochondrial-flux-nnmt-and-ins.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-20 13:05:032026-10-20 13:05:03MOTS-c and 5-Amino-1MQ in Skeletal-Muscle Models: Mitochondrial Flux, NNMT, and Insulin-Signaling Controls
Slupp332 and 5-Amino-1MQ: Liver, Adipocyte, and Mitochondrial Safety Endpoints for Combination Studies

Slupp332 and 5-Amino-1MQ: Liver, Adipocyte, and Mitochondrial Safety Endpoints for Combination Studies

October 20, 2026/0 Comments/in Uncategorized/by

Zero controlled human safety trials exist for either SLU-PP-332 or 5-Amino-1MQ as of 2026, yet capsule stacks combining both compounds are sold openly online, promoted with mouse-injection data and no validated organ toxicology. That gap between commercial availability and scientific evidence defines the central challenge when evaluating Slupp332 and 5-Amino-1MQ: liver, adipocyte, and mitochondrial safety endpoints for combination studies.

This article examines what is known, what is missing, and what rigorous preclinical and clinical safety programs would need to address before either compound, let alone both together, could be used with any meaningful confidence.

Key Takeaways

  • SLU-PP-332 activates estrogen-related receptors (ERRα/β/γ) to drive mitochondrial biogenesis; 5-Amino-1MQ inhibits NNMT in adipose tissue to reduce fat mass, both effects are confirmed only in rodent models.
  • No human pharmacokinetic, hepatotoxicity, or mitochondrial safety data exist for either compound as of late 2026.
  • The quinolinium chemical class to which 5-Amino-1MQ belongs carries unresolved genotoxicity concerns; NNMT inhibition may also suppress 1-methylnicotinamide with hypothetical cardiovascular implications.
  • Grey-market combination products rely entirely on animal injection data, providing no validated liver, adipocyte, or mitochondrial safety endpoints.
  • Future development programs would require GLP-grade rodent toxicology covering hepatic enzymes, adipose morphology, mitochondrial function assays, and cardiovascular markers before any human trial could be justified.

Mechanisms Behind the Combination: What Each Compound Does

Understanding why researchers are interested in pairing these two agents requires a clear look at their individual mechanisms.

Mechanisms Behind the Combination: What Each Compound Does

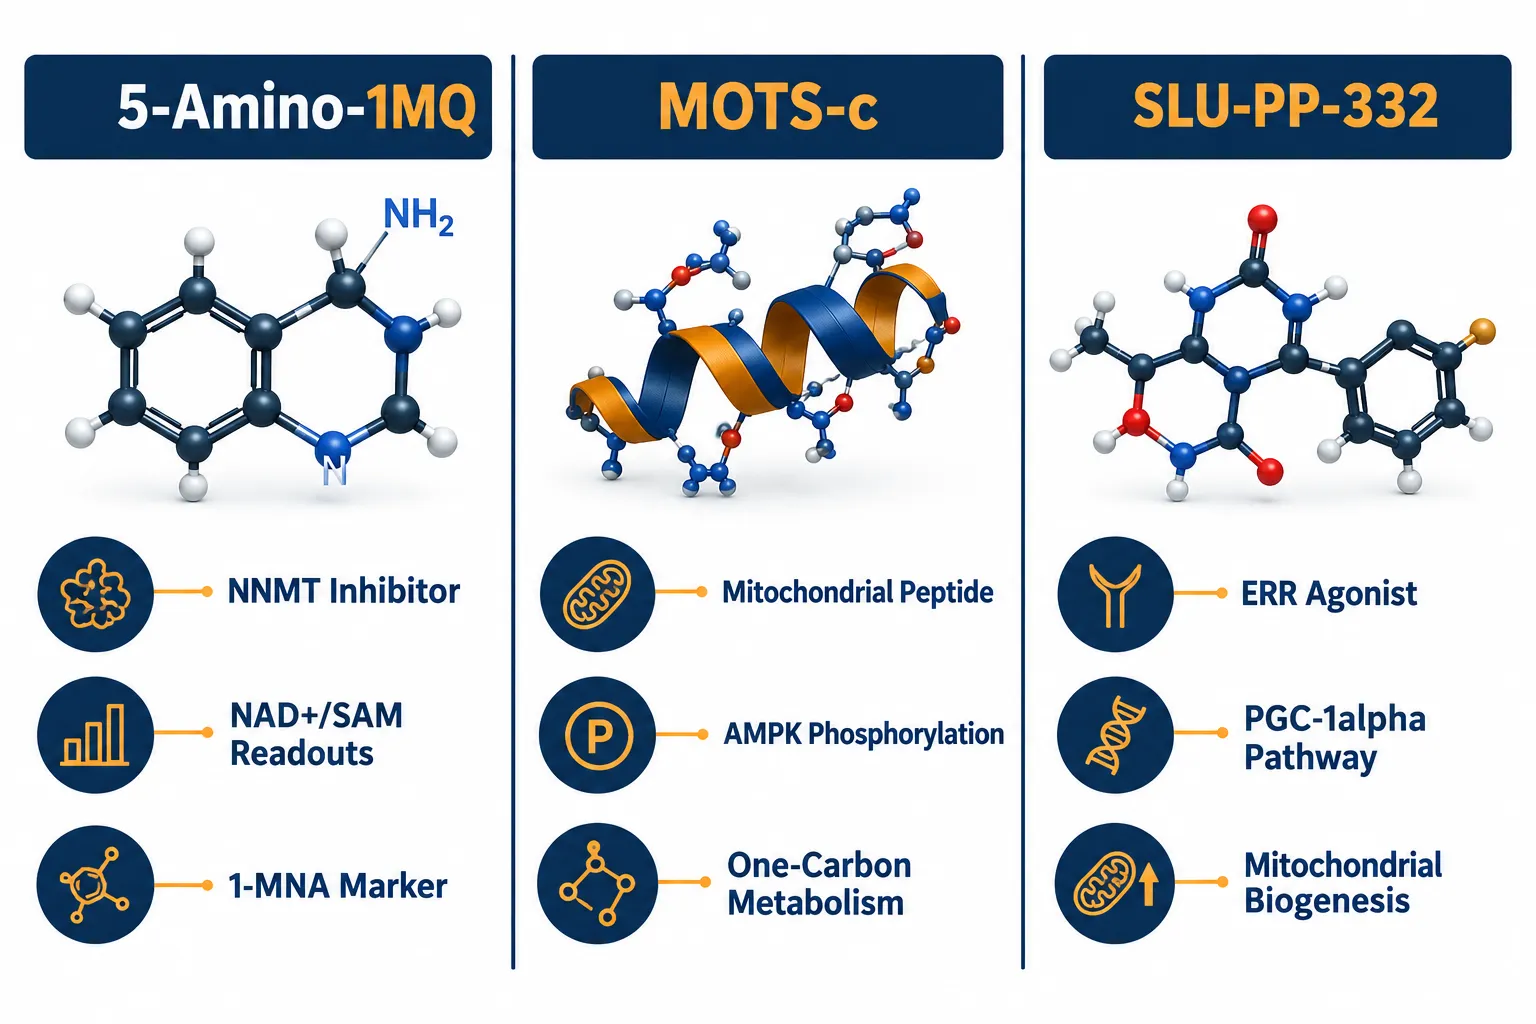
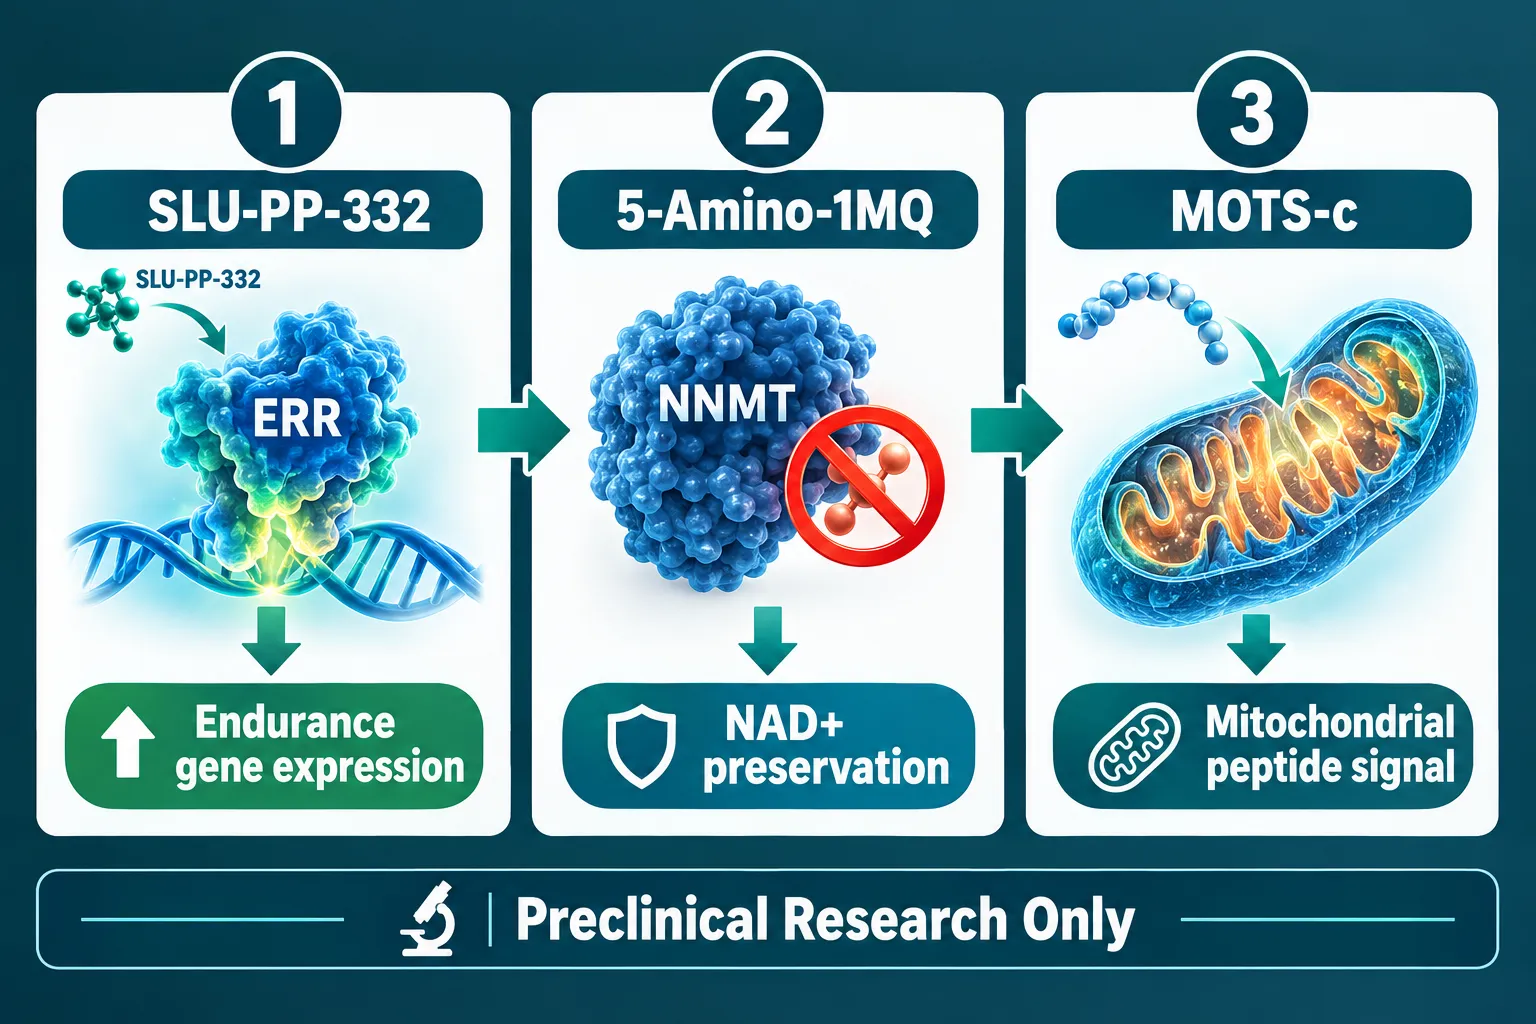
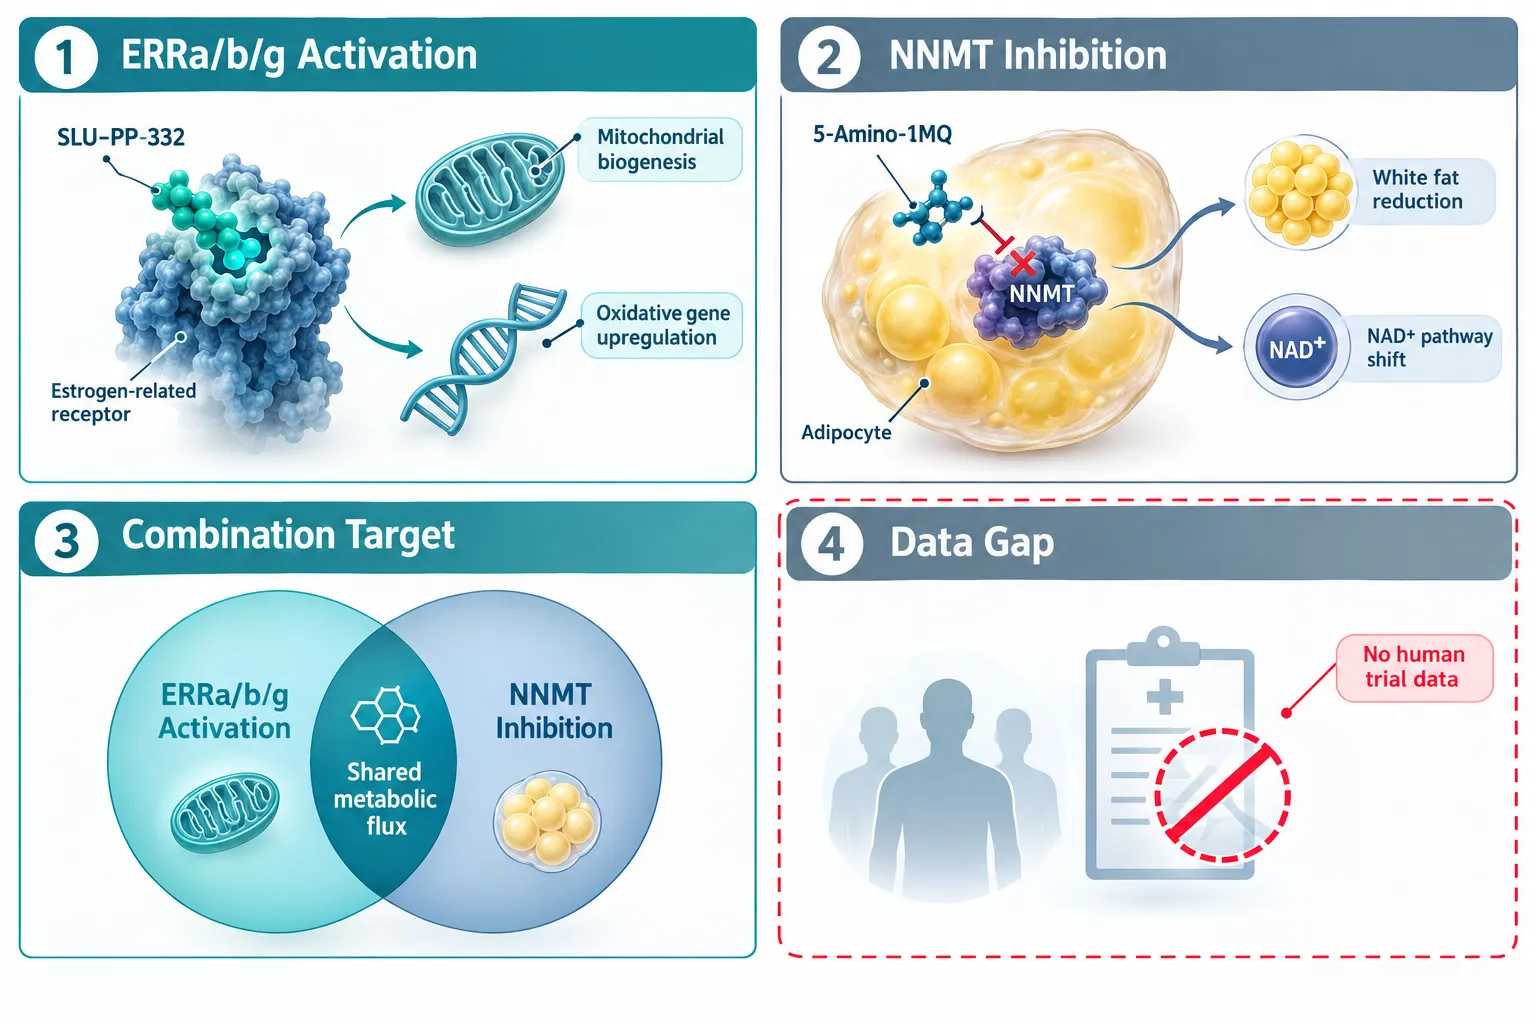
SLU-PP-332 is a synthetic pan-agonist of estrogen-related receptors. It simultaneously activates ERRα, ERRβ, and ERRγ, nuclear receptors that regulate oxidative phosphorylation and mitochondrial biogenesis. In diet-induced obese mouse models, SLU-PP-332 increased expression of oxidative metabolic genes in skeletal muscle, improved running endurance, reduced fat mass, and enhanced insulin sensitivity. Critically, these results came from injected doses; oral bioavailability is acknowledged to be poor even by vendor documentation.

5-Amino-1MQ (5-amino-1-methylquinolinium) is a small-molecule inhibitor of nicotinamide N-methyltransferase (NNMT), an enzyme highly expressed in white adipose tissue. NNMT methylates nicotinamide, diverting it from NAD+ biosynthesis. When NNMT is blocked, more substrate flows back toward NAD+, shifting adipocyte energy balance and reducing white adipose mass in obese rodent models. The compound is not FDA-approved, does not appear in DailyMed, and has no registered human clinical trials as of 2026.

"The mechanistic rationale for combining an ERR pan-agonist with an NNMT inhibitor is scientifically coherent, both touch NAD-related and mitochondrial pathways, but mechanistic plausibility is not the same as demonstrated safety."

Both compounds are frequently mis-marketed as peptides. They are small molecules. That distinction matters for predicting metabolism, hepatic clearance, and potential drug interactions.


Liver, Adipocyte, and Mitochondrial Safety Endpoints: What the Data Actually Show

When evaluating Slupp332 and 5-Amino-1MQ: liver, adipocyte, and mitochondrial safety endpoints for combination studies, the honest summary is brief: rodent data shows no acute organ failure at tested doses, and that is largely where the evidence stops.

Liver, Adipocyte, and Mitochondrial Safety Endpoints: What the Data Actually Show

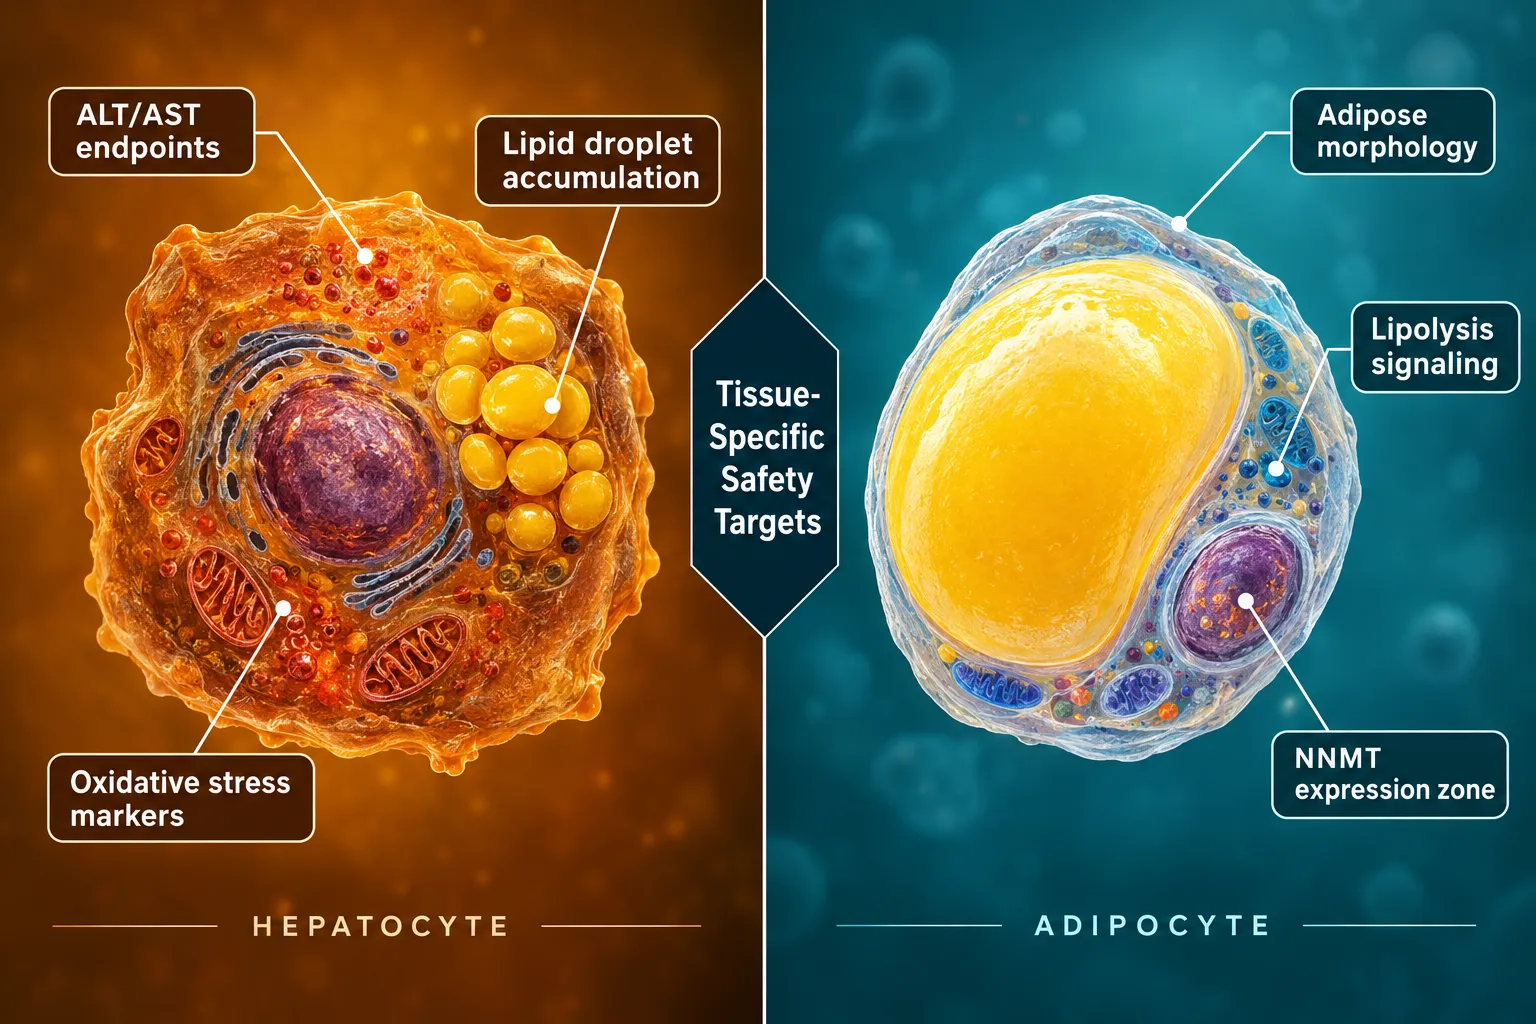
Hepatic Safety Endpoints

No controlled study has measured alanine aminotransferase (ALT), aspartate aminotransferase (AST), or liver histology in animals or humans after either compound at doses translatable to human use. Key gaps include:

  • Transaminase monitoring, no baseline or post-exposure enzyme data in published literature
  • Lipid droplet accumulation, NNMT plays a role in hepatic lipid metabolism; inhibition effects on liver steatosis are uncharacterized
  • Oxidative stress in hepatocytes, ERR activation increases reactive oxygen species (ROS) alongside mitochondrial biogenesis; liver-specific ROS burden has not been quantified

For researchers exploring SS-31 mitochondrial research as a reference point, SS-31's hepatic profile is far better characterized than either compound discussed here, underscoring how immature the SLU-PP-332 and 5-Amino-1MQ safety literature remains.

Adipocyte Safety Endpoints

5-Amino-1MQ targets adipose tissue directly, making adipocyte viability a first-order concern. Missing data include:

Safety Endpoint Rodent Data Available Human Data Available
Adipocyte morphology changes Limited None
Lipolysis dysregulation Indirect None
NNMT expression in non-target tissues Partial None
Adipokine secretion profile None None

The concern is not just toxicity but dysfunction: excessive or off-target NNMT inhibition could disrupt adipokine signaling, with downstream effects on insulin sensitivity and inflammation that no current study has addressed.

Mitochondrial Safety Endpoints

SLU-PP-332's core mechanism, upregulating mitochondrial biogenesis via ERR activation, is also its primary safety question. More mitochondria are not unconditionally beneficial. Uncoupled or dysfunctional mitochondria generate excess ROS. No study has measured:

  • Mitochondrial membrane potential under prolonged ERR activation
  • Oxygen consumption rate in non-muscle tissues (especially liver)
  • Mitophagy regulation or mitochondrial quality control markers

Resources on SS-31 peptide benefits illustrate that mitochondria-targeting compounds require specific assay frameworks; those frameworks simply do not exist yet for SLU-PP-332.


Combination Safety Concerns and Exposure Controls

Evaluating Slupp332 and 5-Amino-1MQ: liver, adipocyte, and mitochondrial safety endpoints for combination studies as a stack introduces additive and potentially synergistic unknowns.

Combination Safety Concerns and Exposure Controls

Genotoxicity and Chemical Class Risk

The quinolinium scaffold in 5-Amino-1MQ is structurally related to known mutagens. Genotoxicity for 5-Amino-1MQ itself has not been formally confirmed or ruled out. Any responsible development program would require an Ames test and in vitro chromosomal aberration assay as first-line screening before advancing to organ-specific endpoints.

1-Methylnicotinamide Suppression

NNMT inhibition reduces 1-methylnicotinamide (1-MNA), a metabolite with proposed cardioprotective and anti-inflammatory properties. Chronic suppression of 1-MNA is a hypothetical cardiovascular risk that has not been evaluated in any controlled model, and it represents a distinct concern from liver or mitochondrial toxicity.

What a Responsible Safety Program Would Require

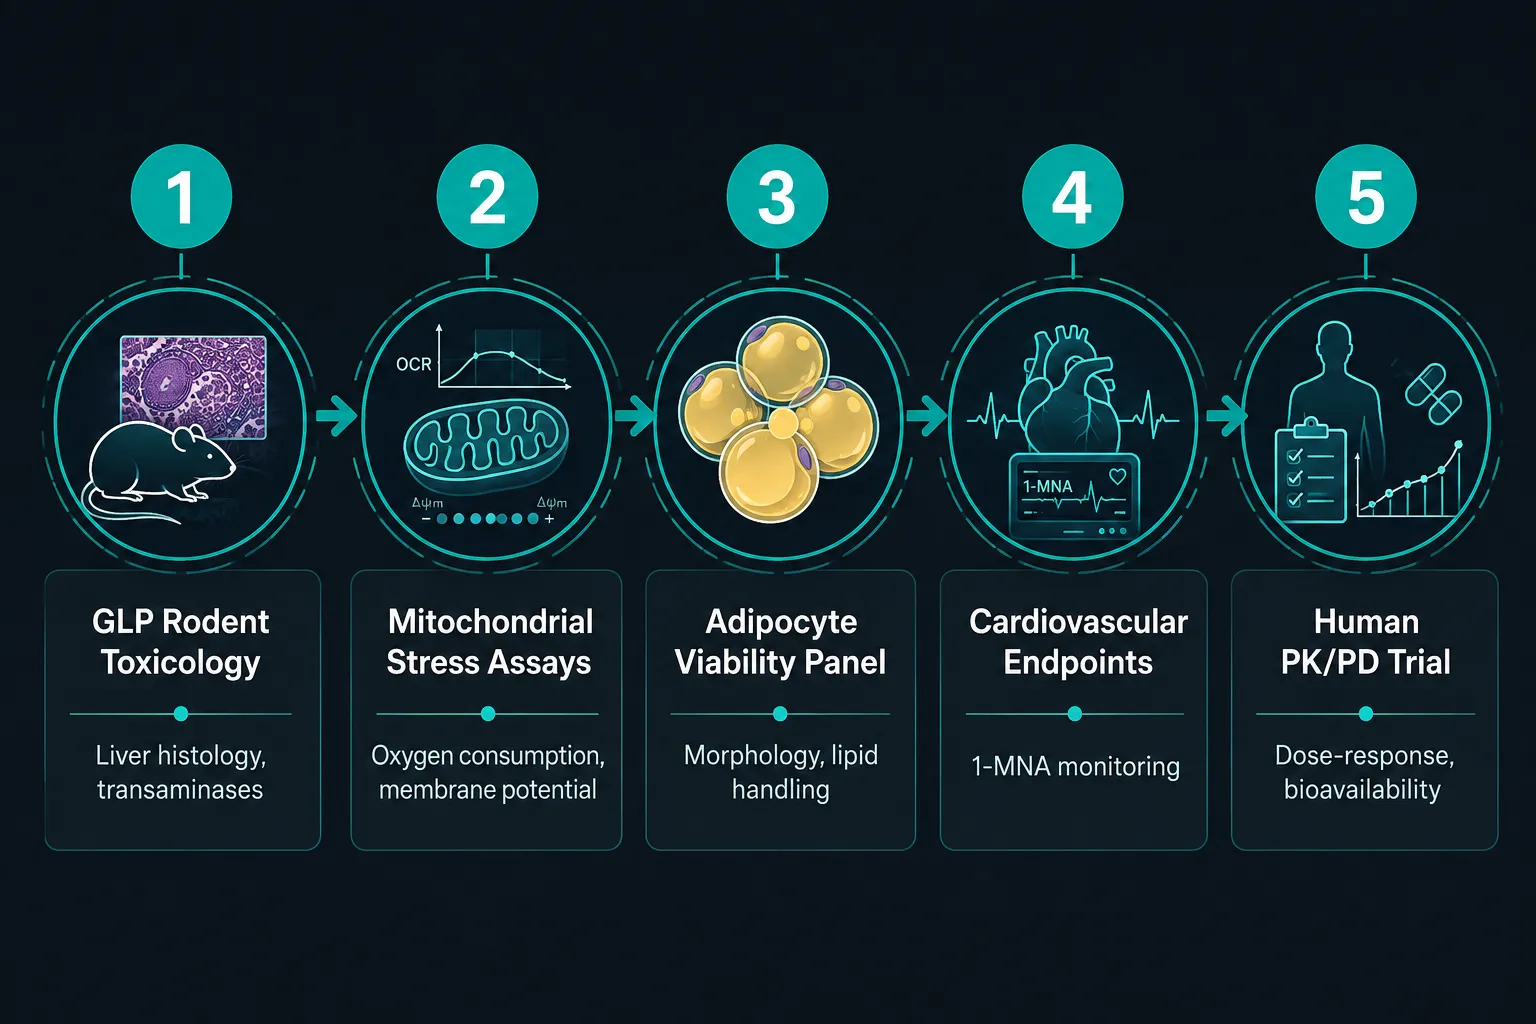
Before any human combination study could be justified, reviewers and mechanistic analyses converge on a minimum preclinical package:

  1. GLP rodent toxicology, 28-day and 90-day repeat-dose studies with full histopathology including liver, kidney, heart, and adipose
  2. Mitochondrial function assays, Seahorse respirometry in hepatocytes and adipocytes exposed to both compounds individually and combined
  3. Hepatic enzyme panels, Serial ALT, AST, alkaline phosphatase, and bilirubin at multiple dose levels
  4. Genotoxicity battery, Ames test, micronucleus assay
  5. Cardiovascular markers, 1-MNA levels, echocardiography in rodent models
  6. Human pharmacokinetic studies, Oral bioavailability, half-life, protein binding, and metabolite identification

For context on how peptide and small-molecule research stacks approach metabolic fat-loss endpoints more broadly, resources on tesa dosage for fat loss demonstrate that even well-studied compounds require robust dose-finding and monitoring before clinical use. Both SLU-PP-332 and 5-Amino-1MQ remain far behind that standard.

Grey-market products now combine 50 mg 5-Amino-1MQ with 1 mg SLU-PP-332 in a single capsule, labeled "not for human consumption." None of these products report GLP-grade toxicology, and all product descriptions draw on rodent injection data, a pharmacokinetic model that does not translate directly to human oral dosing. Interested readers can also review AOD 9604 price and research context as a comparison point for how even more established metabolic research compounds carry significant regulatory and data limitations.


Conclusion

The scientific case for combining SLU-PP-332 and 5-Amino-1MQ is mechanistically interesting: ERR pan-agonism plus NNMT inhibition could theoretically complement each other across mitochondrial and adipose metabolic pathways. However, the safety case does not exist yet. As of 2026, no human clinical data, no formal hepatic enzyme monitoring, no adipocyte viability assays, and no mitochondrial stress protocols have been published for either compound, individually or in combination.

Actionable next steps for researchers and clinicians:

  • Treat any commercial combination product as entirely experimental with undetermined organ-specific risk.
  • Prioritize genotoxicity screening for 5-Amino-1MQ given its quinolinium structure before any chronic exposure model.
  • Design future preclinical programs to include liver histology, mitochondrial respirometry, adipose morphology, and 1-MNA cardiovascular monitoring as minimum endpoints.
  • Consult resources on established mitochondria-targeting compounds, such as SS-31 elamipretide, to understand what a mature safety profile for a mitochondrial compound actually looks like.
  • Do not conflate rodent injection efficacy data with human oral safety data; the two are categorically different.

The evidence gap is not a reason to dismiss future research into this combination, it is a precise map of what that research must address first.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/slupp332-and-5-amino-1mq-liver-adipocyte-and-mitochondrial-safety-endpoints-for.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-20 13:03:502026-10-20 13:03:50Slupp332 and 5-Amino-1MQ: Liver, Adipocyte, and Mitochondrial Safety Endpoints for Combination Studies
Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy

Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy

October 14, 2026/0 Comments/in Uncategorized/by

Fewer than a dozen peer-reviewed studies have examined SLU-PP-332 in living systems, and preclinical data for 5-Amino-1MQ remain almost entirely confined to rodent adipose models, yet both compounds are already being marketed together as a "multifaceted metabolic approach." The topic of Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy matters precisely because combining two mechanistically distinct research compounds without a proper factorial design produces uninterpretable data and, worse, misleading conclusions.

Key Takeaways

  • SLU-PP-332 and 5-Amino-1MQ act through completely separate molecular targets and should never be assumed to produce synergistic effects without statistical proof.
  • A factorial experimental design with at least four treatment arms is the minimum standard for testing whether an interaction between these compounds actually exists.
  • Metabolic flux endpoints, oxygen consumption rate, NAD+/NADH ratio, NNMT enzyme activity, must be measured independently before any combination data can be interpreted.
  • Neither compound has completed human obesity trials or received regulatory approval as of 2026; all data are preclinical or in vitro.
  • Marketing language about "synergy" is not a substitute for an interaction F-test in a properly powered study.

Distinct Mechanisms: Why Assuming Synergy Is a Scientific Error

Distinct Mechanisms: Why Assuming Synergy Is a Scientific Error

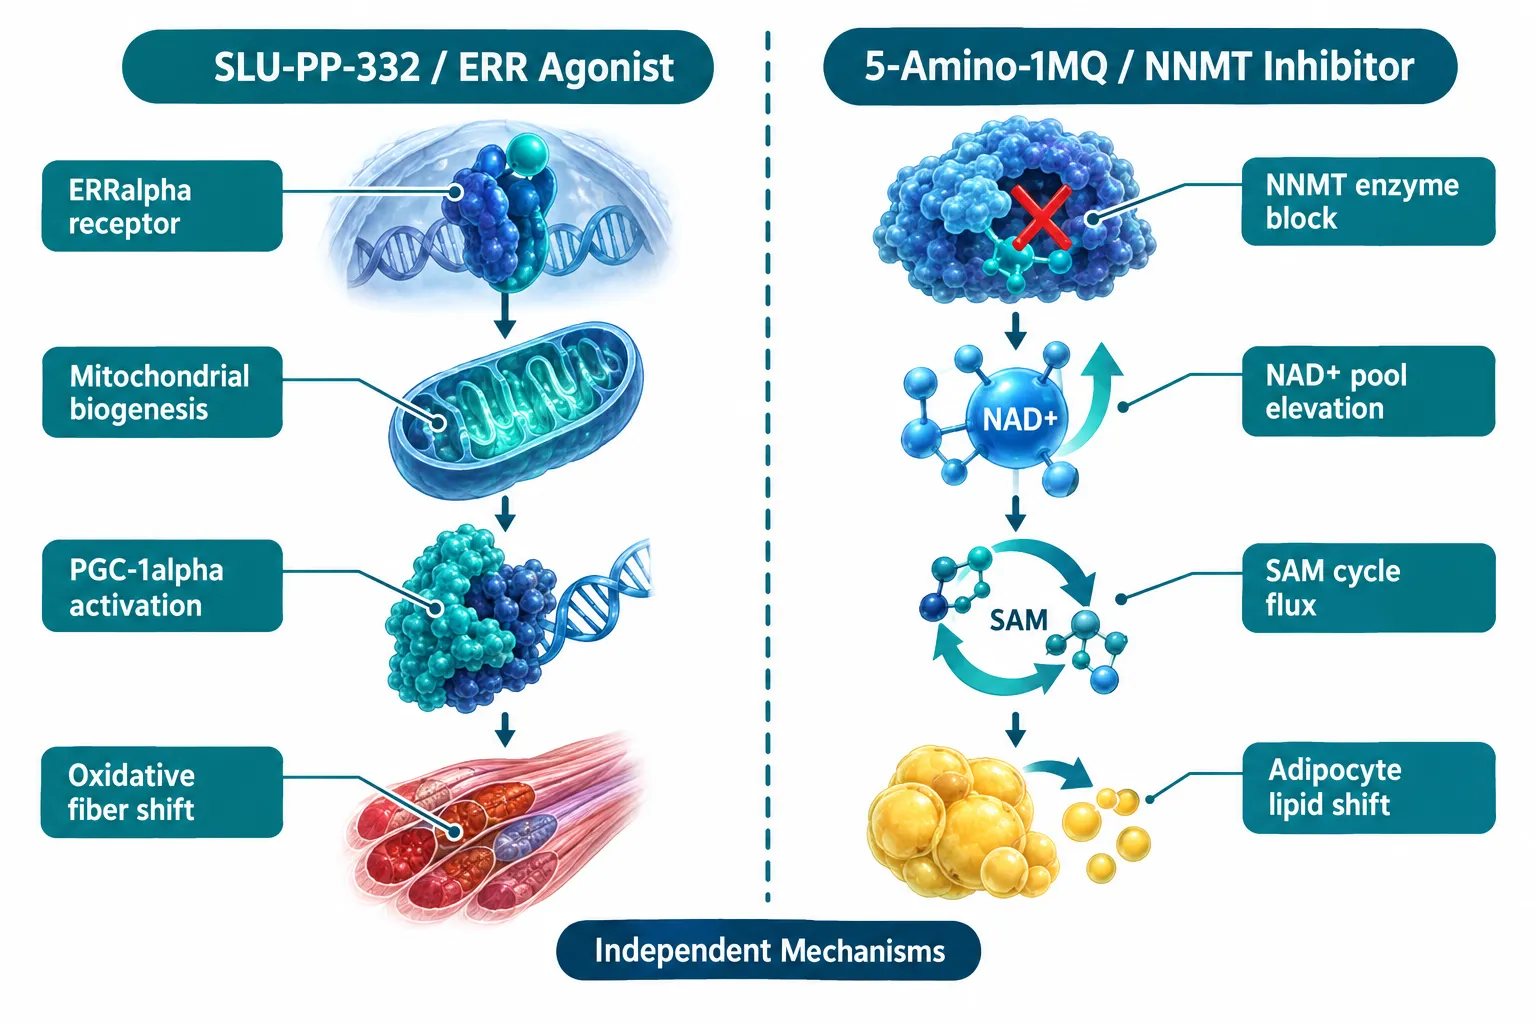
Understanding Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy begins with a clear separation of mechanisms.

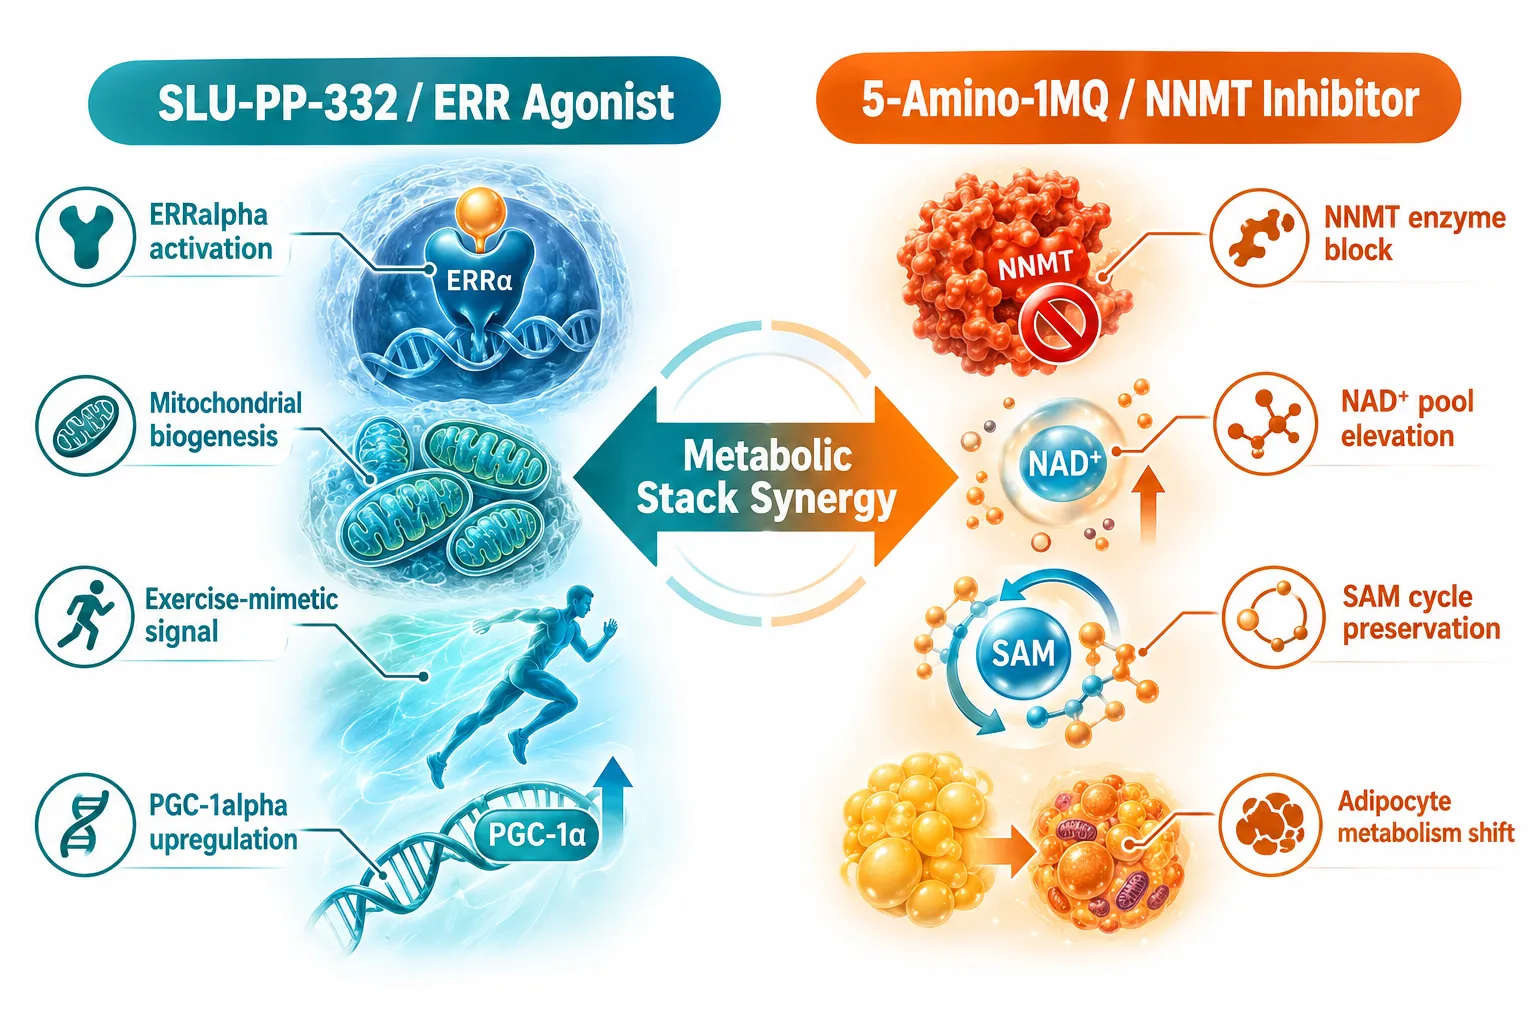
SLU-PP-332 (SLU-PP-332) is an agonist of estrogen-related receptors, particularly ERRalpha and ERRgamma. These nuclear receptors regulate mitochondrial biogenesis, oxidative phosphorylation gene expression, and the shift toward slow-twitch, fatigue-resistant muscle fiber types. Its endurance-related effects in rodent models have drawn comparisons to exercise adaptation, which is where the "exercise pill" label, and the skepticism that follows it, originates.

5-Amino-1MQ works through an entirely different mechanism. It inhibits nicotinamide N-methyltransferase (NNMT), an enzyme that consumes S-adenosylmethionine (SAM) while methylating nicotinamide. By blocking NNMT, the compound is thought to elevate intracellular NAD+ pools and shift the SAM cycle, which in turn influences adipocyte differentiation and lipid storage. Preclinical obesity data in rodents show modest reductions in fat mass, but these findings have not been replicated in human trials.

"Two compounds acting on different enzymes and receptors are not automatically additive, let alone synergistic. Interaction must be demonstrated, not assumed."

The practical implication is straightforward: because ERR agonism and NNMT inhibition operate on separate nodes of the metabolic network, their combined effect could be additive, sub-additive, or genuinely synergistic, and only a properly designed experiment can tell which.

For broader context on how small molecules like these fit into the research peptide landscape, the Peptides 101 for research-use only buyers guide provides useful background on structure, mechanisms, and compound classification.


Building a Factorial Design for Metabolic Flux Research

Building a Factorial Design for Metabolic Flux Research

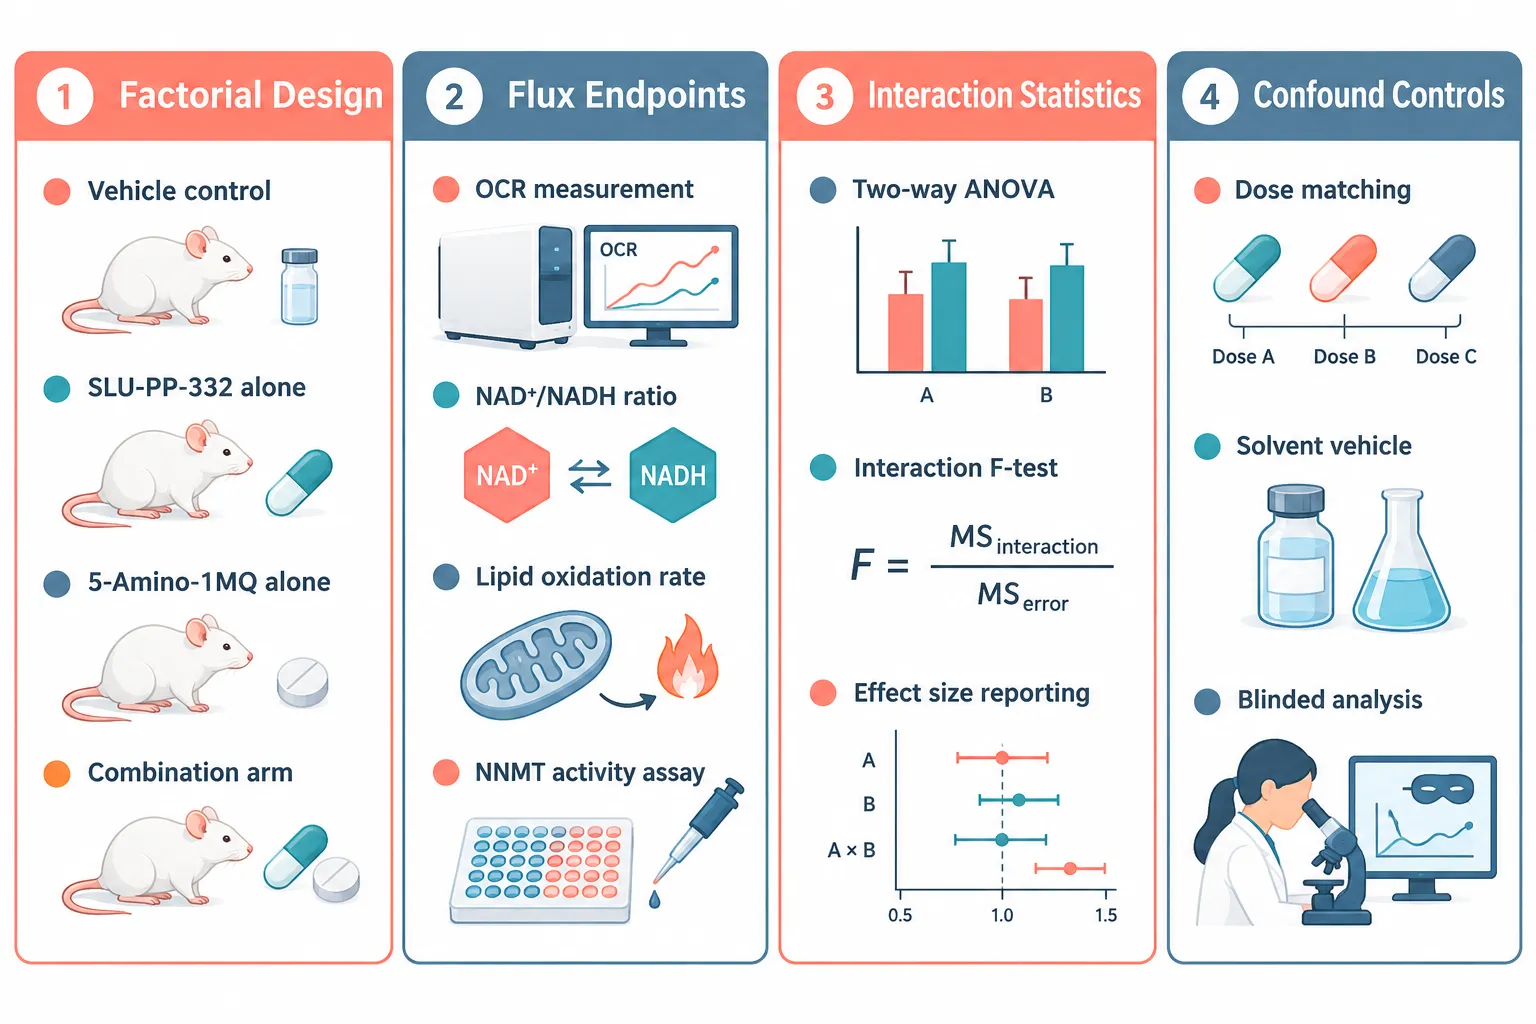
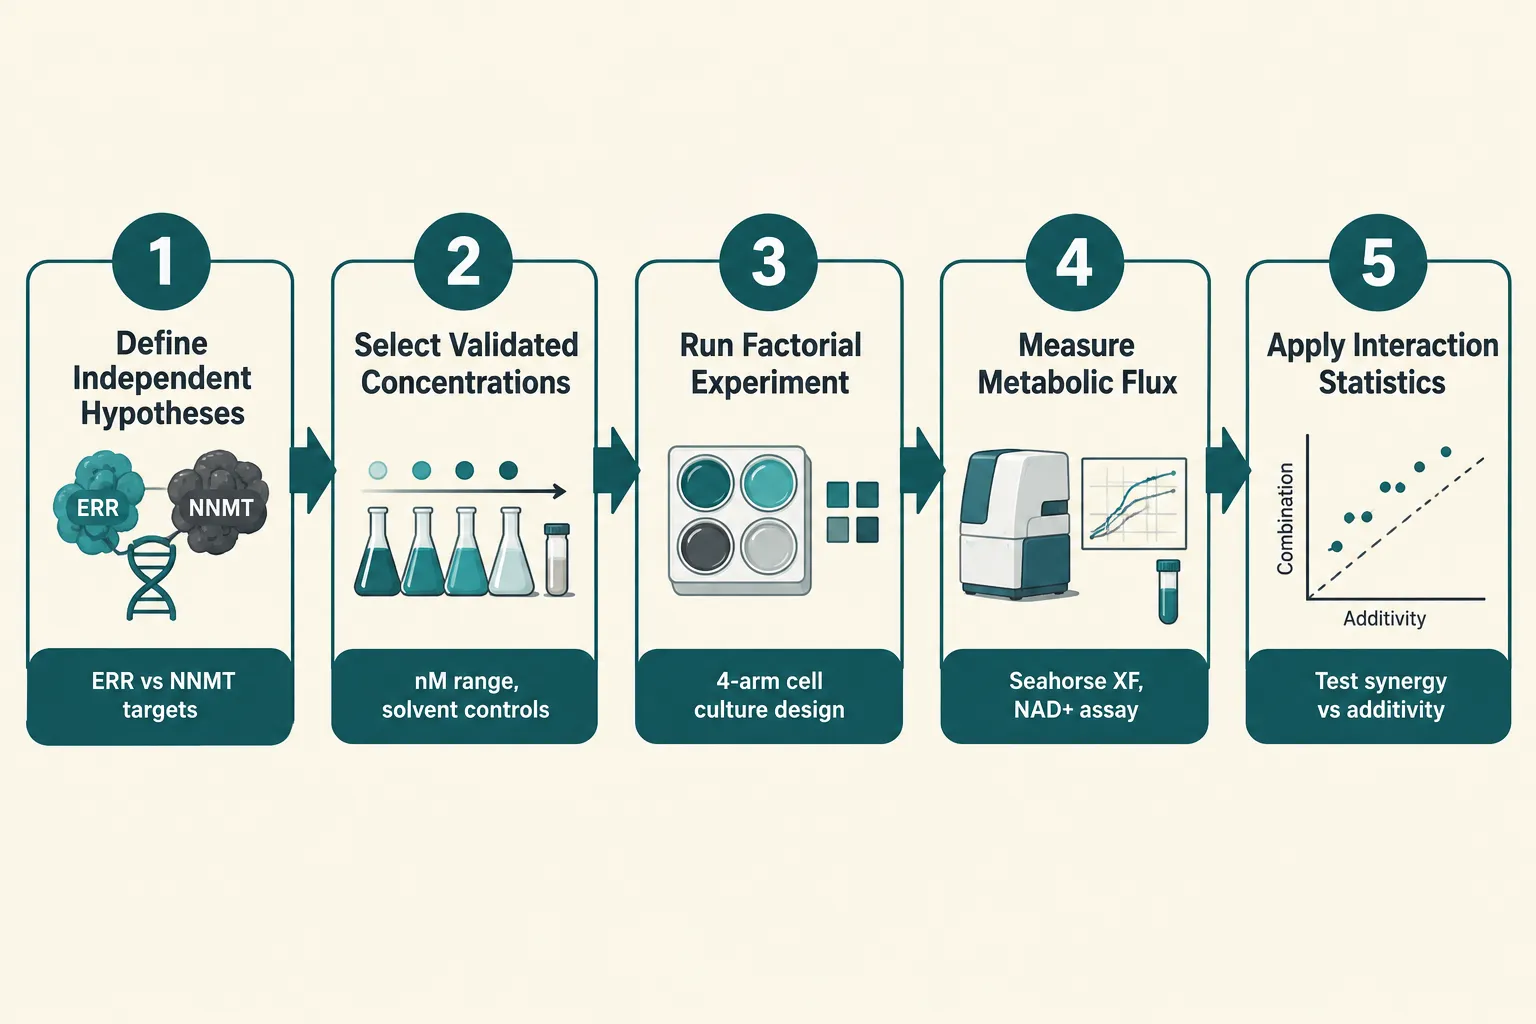
The core framework for Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy is a 2×2 factorial design with four treatment arms:

Building a Factorial Design for Metabolic Flux Research

Arm SLU-PP-332 5-Amino-1MQ
1 (Vehicle control) No No
2 (ERR agonist only) Yes No
3 (NNMT inhibitor only) No Yes
4 (Combination) Yes Yes

This structure allows researchers to calculate a true interaction term using two-way ANOVA. If the combination arm produces an effect that is statistically greater than the sum of arms 2 and 3, synergy is supported. If not, the null hypothesis of additivity stands.

Concentration and Solvent Controls

Both compounds present solubility challenges. SLU-PP-332 is typically dissolved in DMSO, and 5-Amino-1MQ requires aqueous buffering at physiological pH. Solvent vehicle controls must be matched across all arms, a step frequently omitted in informal or commercially motivated reports. Recommended starting concentrations for in vitro work are in the low nanomolar to low micromolar range, with dose-response curves run before any combination experiment begins.

Choosing Flux-Oriented Endpoints

The following endpoints are appropriate for this experimental framework:

  • Oxygen consumption rate (OCR): Measured via Seahorse XF analysis; reflects mitochondrial respiration and is the primary readout for SLU-PP-332 activity.
  • NAD+/NADH ratio: Enzymatic cycling assay; the primary quantitative readout for 5-Amino-1MQ's effect on the NAD+ pool.
  • NNMT enzyme activity: Direct fluorometric assay using nicotinamide substrate; confirms target engagement for 5-Amino-1MQ.
  • Lipid oxidation rate: Radiolabeled fatty acid oxidation or Seahorse fatty acid oxidation kit; relevant to both compounds' downstream effects on adipose metabolism.
  • PGC-1alpha and ERR target gene expression: RT-qPCR panel; confirms SLU-PP-332 target engagement at the transcriptional level.

Researchers interested in related metabolic compounds used in aging-support contexts can explore the aging support product category for additional reference compounds.


Interpreting Results and Avoiding Hype-Driven Conclusions

Once data are collected, the analysis must be hypothesis-driven. The interaction F-test in the two-way ANOVA is the statistical gatekeeper. A non-significant interaction term means the compounds behave independently at the doses tested, a finding that is scientifically valid and publishable, even if it contradicts marketing claims.

Expert commentary in the metabolic pharmacology field consistently flags two problems with current discourse around these compounds:

  1. The "exercise pill" narrative overstates SLU-PP-332's translatability from rodent treadmill models to human endurance physiology.
  2. The "fat-loss stack" narrative for 5-Amino-1MQ extrapolates rodent adipose data to human obesity without bridging pharmacokinetic or dose-equivalence data.

Neither compound has completed a human obesity trial or received regulatory approval as of late 2026. Researchers should clearly label any speculative expectations as such in publications and protocols.

For comparison, examining how well-characterized peptide combinations are studied, such as the safety considerations for combining Tesamorelin with CJC Ipamorelin, illustrates the importance of independent mechanism validation before combination claims are made. Similarly, the Tesamorelin vs Sermorelin comparison demonstrates how mechanistic differences between compounds inform experimental design choices.

Researchers working with growth hormone-related peptides in parallel studies may also find the Sermorelin vs CJC-1295 analysis useful for understanding how distinct receptor targets require separate experimental arms.

Reporting Standards

Published reports on this compound pair should include:

  • Full dose-response data for each compound alone
  • Solvent vehicle control data
  • The interaction F-statistic and p-value
  • Effect sizes (partial eta-squared or Cohen's d)
  • Clear labeling of in vitro vs. in vivo results

Conclusion

The scientific value of studying SLU-PP-332 and 5-Amino-1MQ together depends entirely on the rigor of the experimental design. Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy is not just a methodological preference, it is the minimum standard for producing data that can actually advance understanding of metabolic flux modulation.

Actionable next steps for researchers:

  • Run single-compound dose-response curves before any combination experiment.
  • Build a 2×2 factorial design with matched solvent controls in all four arms.
  • Select flux endpoints that directly reflect each compound's known mechanism: OCR for SLU-PP-332, NAD+/NADH and NNMT activity for 5-Amino-1MQ.
  • Pre-register the interaction hypothesis and the statistical analysis plan before data collection begins.
  • Report interaction statistics explicitly, and distinguish between additive and synergistic outcomes in all communications.

The field does not need more marketing-style synergy claims. It needs properly powered factorial experiments with quantitative flux data and honest statistical reporting.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/slupp332-and-5-amino-1mq-designing-metabolic-flux-experiments-without-assuming-s.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-14 13:04:262026-10-14 13:04:26Slupp332 and 5-Amino-1MQ: Designing Metabolic Flux Experiments Without Assuming Synergy
Vitamin D, MOTS-c, and 5-Amino-1MQ: Designing Nutrient-Controlled Cellular Energy Experiments

Vitamin D, MOTS-c, and 5-Amino-1MQ: Designing Nutrient-Controlled Cellular Energy Experiments

October 2, 2026/0 Comments/in Uncategorized/by

Researchers who publish conflicting results on metabolic peptides often share one overlooked flaw: they never standardized the vitamin D status of their cell cultures or animal models before the experiment began. That single omission can silently shift AMPK activity, mitochondrial respiration, and insulin signaling, making every downstream comparison unreliable. Understanding how to design nutrient-controlled cellular energy experiments around Vitamin D, MOTS-c, and 5-Amino-1MQ is therefore not a minor methodological footnote; it is the foundation of reproducible metabolic science.

Key Takeaways

  • Vitamin D, acting through the vitamin D receptor (VDR), directly modulates AMPK, mTOR, and mitochondrial oxidative capacity, making vitamin D status a critical baseline variable in any cellular energy experiment.
  • MOTS-c is a 16-amino-acid mitochondrial-derived peptide that activates AMPK by accumulating AICAR, linking mitochondrial stress signals to whole-cell energy regulation.
  • 5-Amino-1MQ inhibits nicotinamide N-methyltransferase (NNMT), redirecting nicotinamide toward NAD+ biosynthesis and reshaping cellular energy and lipid metabolism.
  • All three agents converge on the AMPK-SIRT1-PGC-1alpha axis, meaning their effects are not independent, experimental designs must account for this overlap.
  • Standardizing media composition, vitamin D concentration, and mitochondrial readout methods before adding peptide or small-molecule treatments is essential for valid, reproducible results.

Why Vitamin D Status Must Be Standardized First

Why Vitamin D Status Must Be Standardized First

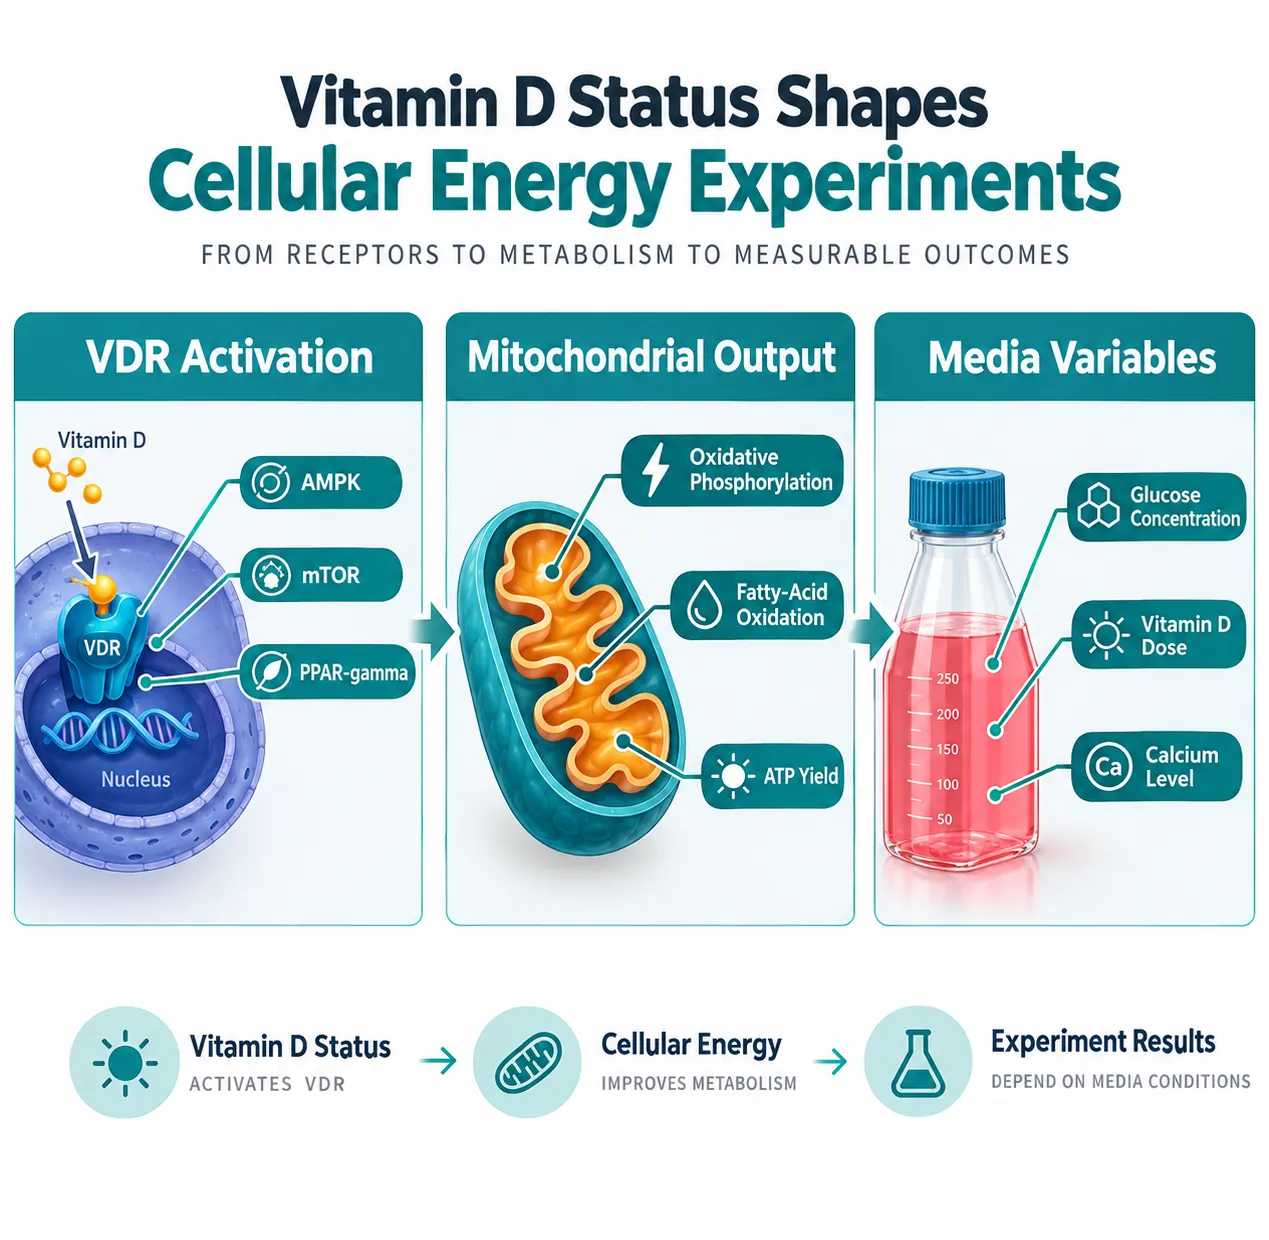
Most cell-culture media formulations contain little to no vitamin D, yet researchers rarely report the vitamin D content of their experimental system. This gap matters because the active form of vitamin D, calcitriol, enhances mitochondrial fatty-acid oxidation and oxidative phosphorylation in muscle cells. Human supplementation studies confirm that cholecalciferol increases oxidative phosphorylation capacity and improves muscle function, effects that translate directly to the readouts used in cellular energy assays.

The mechanism runs through the vitamin D receptor (VDR), which is expressed in adipocytes, hepatocytes, skeletal muscle, beta-cells, endothelial cells, and immune cells. VDR activation modulates several signaling nodes that are central to cellular energy regulation:

Signaling Node Role in Energy Metabolism
AMPK Cellular energy sensor; activates catabolic pathways
mTOR Anabolic signaling; suppressed during energy deficit
NF-kB Inflammatory regulator; linked to mitochondrial stress
PPAR-gamma Lipid metabolism and adipogenesis control

Because these pathways overlap with classic exercise and nutrient-stress responses, an experiment that ignores vitamin D status is effectively running with an uncontrolled variable sitting at the top of the signaling cascade. A 2026 mechanistic review on vitamin D and metabolic syndrome positions VDR-dependent signaling as a core modulator of insulin sensitivity, oxidative stress, and mitochondrial function, reinforcing that vitamin D belongs in the experimental design checklist, not the supplementary materials.

Practical standardization steps include:

  • Measuring baseline 25-hydroxyvitamin D in serum before animal studies
  • Supplementing cell culture media with a defined calcitriol concentration
  • Running a vitamin D-deficient control arm alongside replete conditions
  • Reporting media composition fully in the methods section

MOTS-c and 5-Amino-1MQ: Mechanisms Within a Nutrient-Controlled Framework

MOTS-c and 5-Amino-1MQ: Mechanisms Within a Nutrient-Controlled Framework

With a stable vitamin D baseline established, researchers can introduce the two experimental agents most relevant to nutrient-controlled cellular energy work: the mitochondrial peptide MOTS-c and the NNMT inhibitor 5-Amino-1MQ.

MOTS-c: A Mitochondrial Stress Peptide That Reads Nutrient State

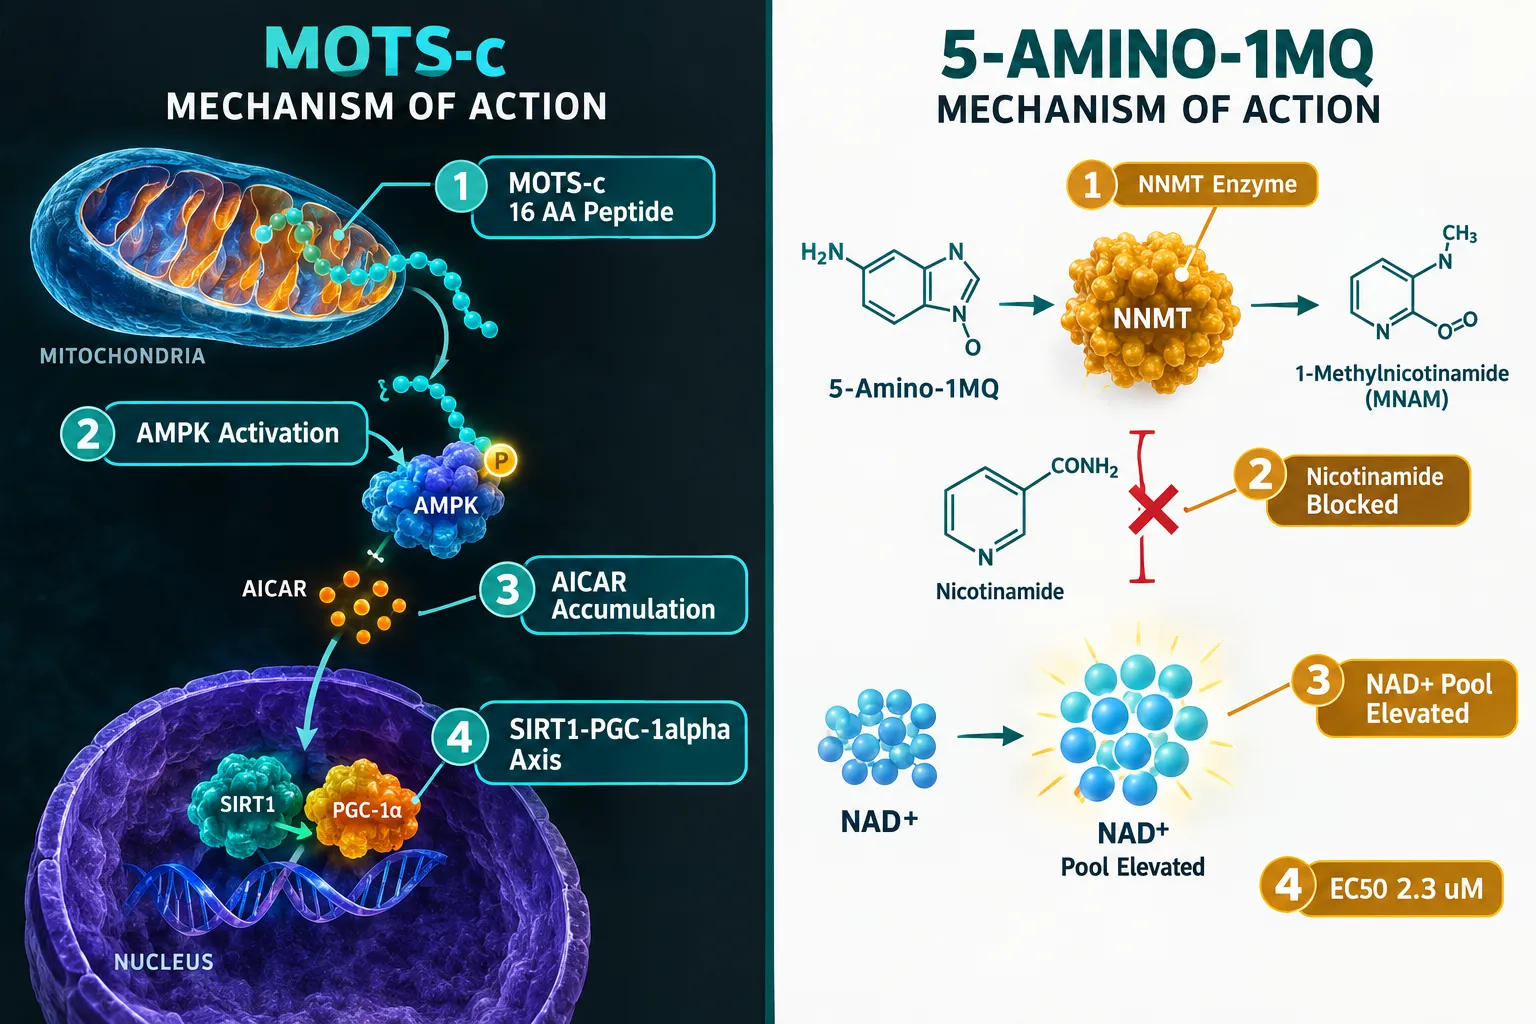
MOTS-c is a 16-amino-acid microprotein encoded within the 12S rRNA of mitochondrial DNA. Its primary mechanism involves inhibiting the folate cycle and de novo purine synthesis, which causes accumulation of AICAR, an endogenous AMPK agonist. This makes MOTS-c a direct link between mitochondrial stress and the cell's central energy "fuel gauge."

Under metabolic stress such as nutrient deprivation or mitochondrial dysfunction, MOTS-c translocates to the nucleus in an AMPK-dependent manner, where it regulates gene expression programs that optimize mitochondrial function and enhance antioxidant defenses. A 2026 translational review describes MOTS-c as part of a secreted mitochondrial microprotein network engaging the canonical AMPK → SIRT1 → PGC-1alpha axis, the same cascade driven by endurance exercise and caloric restriction.

Preclinical data from 2025 show that MOTS-c restores mitochondrial respiration in the type 2 diabetic heart, improving oxygen consumption and cardiac bioenergetics. Separate 2025 work reports that MOTS-c prevents metabolic derangements via regulation of both AMPK and mTOR pathways. Researchers exploring these effects can source MOTS-c peptide for in-vitro and preclinical work.

"MOTS-c does not act in isolation, its potency is shaped by the nutrient environment the cell is already experiencing when the peptide arrives."

5-Amino-1MQ: Redirecting NAD+ Through NNMT Inhibition

5-Amino-1MQ (5-amino-1-methylquinolinium) is a small-molecule inhibitor of nicotinamide N-methyltransferase (NNMT), the cytosolic enzyme that methylates nicotinamide, a NAD+ precursor, using SAM as the methyl donor. By occupying the nicotinamide-binding pocket of NNMT, 5-Amino-1MQ blocks this diversion and reshapes cellular NAD+ and methyl-donor pools.

In differentiated adipocyte models, 5-Amino-1MQ demonstrates concentration-dependent NNMT inhibition with a calculated EC50 of approximately 2.3 µM, providing a practical dose range for in-vitro studies. At effective concentrations, it reduces intracellular 1-methylnicotinamide, elevates NAD+ levels, and suppresses lipogenesis, demonstrating that NNMT inhibition can reroute nicotinamide toward energy metabolism rather than fat-storage pathways.

Preclinical obesity models show that 5-Amino-1MQ reverses diet-induced obesity, improves glucose tolerance, enhances insulin sensitivity, and attenuates fatty-liver changes. Research on 5-Amino-1MQ capsules and related 5-amino peptide compounds continues to expand as interest in NAD+ metabolism grows. Notably, NNMT inhibition also helps preserve nicotinamide and NMN as NAD+ precursors in skeletal muscle, connecting 5-Amino-1MQ to muscle bioenergetics research.


Designing the Three-Axis Experiment

Designing the Three-Axis Experiment

The convergence of all three agents on the AMPK-SIRT1-PGC-1alpha axis is both an opportunity and a methodological challenge. Vitamin D acts primarily via nuclear VDR-dependent transcription. MOTS-c operates as a mitochondria-encoded stress peptide converging on AMPK and SIRT1. 5-Amino-1MQ reshapes NAD+ availability, which directly feeds SIRT1 activity. These are not independent levers, pulling one affects the others.

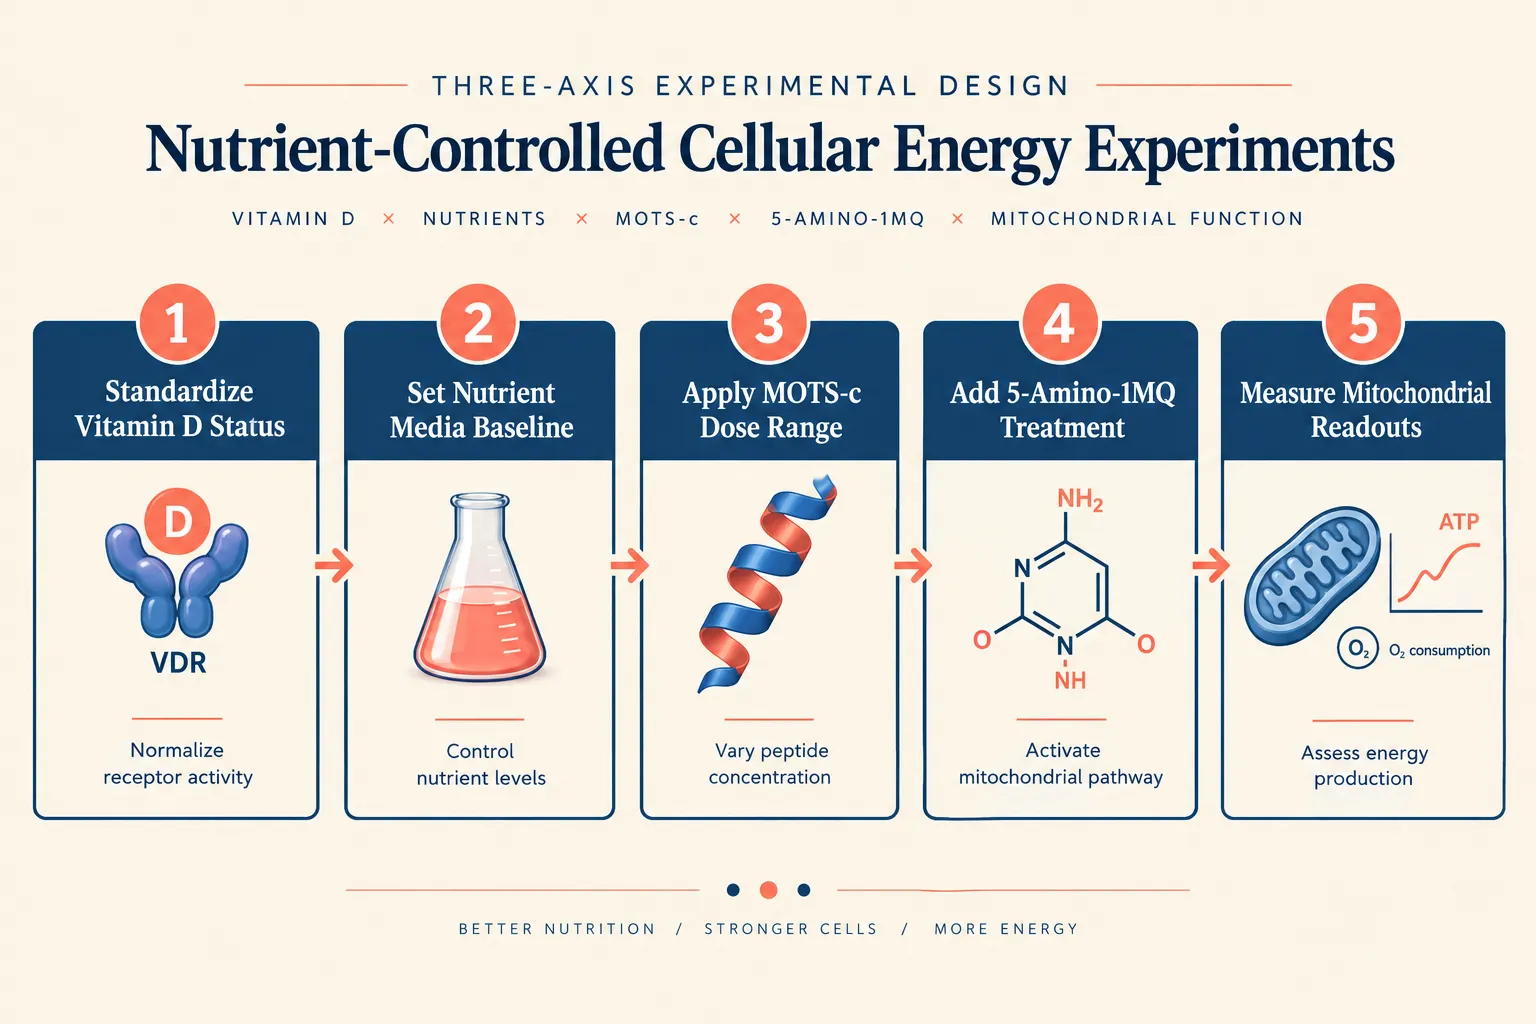
A rational three-axis experimental framework for Vitamin D, MOTS-c, and 5-Amino-1MQ: Designing Nutrient-Controlled Cellular Energy Experiments looks like this:

Axis 1, Vitamin D (VDR-dependent metabolic signaling)

  • Vary: deficient vs. replete calcitriol concentrations in media
  • Measure: VDR target gene expression, AMPK phosphorylation, mitochondrial membrane potential

Axis 2, MOTS-c (acute AMPK activation and stress response)

  • Vary: peptide concentration and timing relative to nutrient stress
  • Measure: oxygen consumption rate, AICAR levels, PGC-1alpha expression

Axis 3-5-Amino-1MQ (NAD+ salvage and NNMT inhibition)

  • Vary: concentration from sub-EC50 to supra-EC50 (reference: ~2.3 µM EC50)
  • Measure: intracellular NAD+/NADH ratio, 1-methylnicotinamide, lipogenesis markers

Combining these axes with controlled glucose, fatty-acid, and amino-acid availability allows researchers to interrogate how endocrine nutrients, mitochondrial microproteins, and NAD+ salvage pathways jointly determine ATP production, substrate choice, and resilience to metabolic stress. For researchers interested in related mitochondrial research tools, SS-31 mitochondrial research resources and NAD+ compounds offer complementary experimental angles. Additional context on how peptides fit into broader cardiometabolic models can be found in this overview of polypeptides in cardiometabolic models.

Critical readouts to standardize across all arms:

  • Oxygen consumption rate (OCR) and extracellular acidification rate (ECAR) via Seahorse or equivalent
  • ATP production rate separated by oxidative phosphorylation vs. glycolysis
  • Mitochondrial biogenesis markers (PGC-1alpha, TFAM, mtDNA copy number)
  • Oxidative stress indicators (mitochondrial ROS, glutathione ratio)

Conclusion

Designing nutrient-controlled cellular energy experiments with Vitamin D, MOTS-c, and 5-Amino-1MQ requires treating vitamin D not as background noise but as an active experimental variable. Before any peptide or small molecule is introduced, vitamin D status in the model system must be defined, controlled, and reported. From that stable foundation, MOTS-c can be used to probe acute AMPK-driven mitochondrial stress responses, while 5-Amino-1MQ reshapes the NAD+ landscape through NNMT inhibition, two complementary tools that, together with vitamin D, map the full AMPK-SIRT1-PGC-1alpha signaling network.

Actionable next steps for researchers in 2026:

  1. Audit current cell-culture and animal-model protocols for vitamin D content and add a deficient-versus-replete arm to ongoing studies.
  2. Select MOTS-c dose ranges based on published preclinical respiration data and confirm AICAR accumulation as a mechanistic marker.
  3. Use the ~2.3 µM EC50 reference for 5-Amino-1MQ to build a concentration-response curve before committing to a single treatment dose.
  4. Report all three axes, vitamin D status, peptide concentration, and NNMT inhibitor dose, alongside nutrient media composition in every methods section.
  5. Prioritize OCR and NAD+/NADH ratio as primary readouts to capture both mitochondrial and metabolic dimensions of the experiment.

All three agents remain experimental tools rather than approved therapeutics, but their mechanistic precision makes them among the most powerful instruments available for dissecting nutrient-sensing and energy-metabolism pathways in 2026.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/vitamin-d-mots-c-and-5-amino-1mq-designing-nutrient-controlled-cellular-energy-e.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-02 13:10:472026-10-02 13:10:47Vitamin D, MOTS-c, and 5-Amino-1MQ: Designing Nutrient-Controlled Cellular Energy Experiments
5-Amino-1MQ and MOTS-c Co-Treatment: A Matrix for Dose-Response, Additivity, and Interaction Testing

5-Amino-1MQ and MOTS-c Co-Treatment: A Matrix for Dose-Response, Additivity, and Interaction Testing

October 2, 2026/0 Comments/in Uncategorized/by

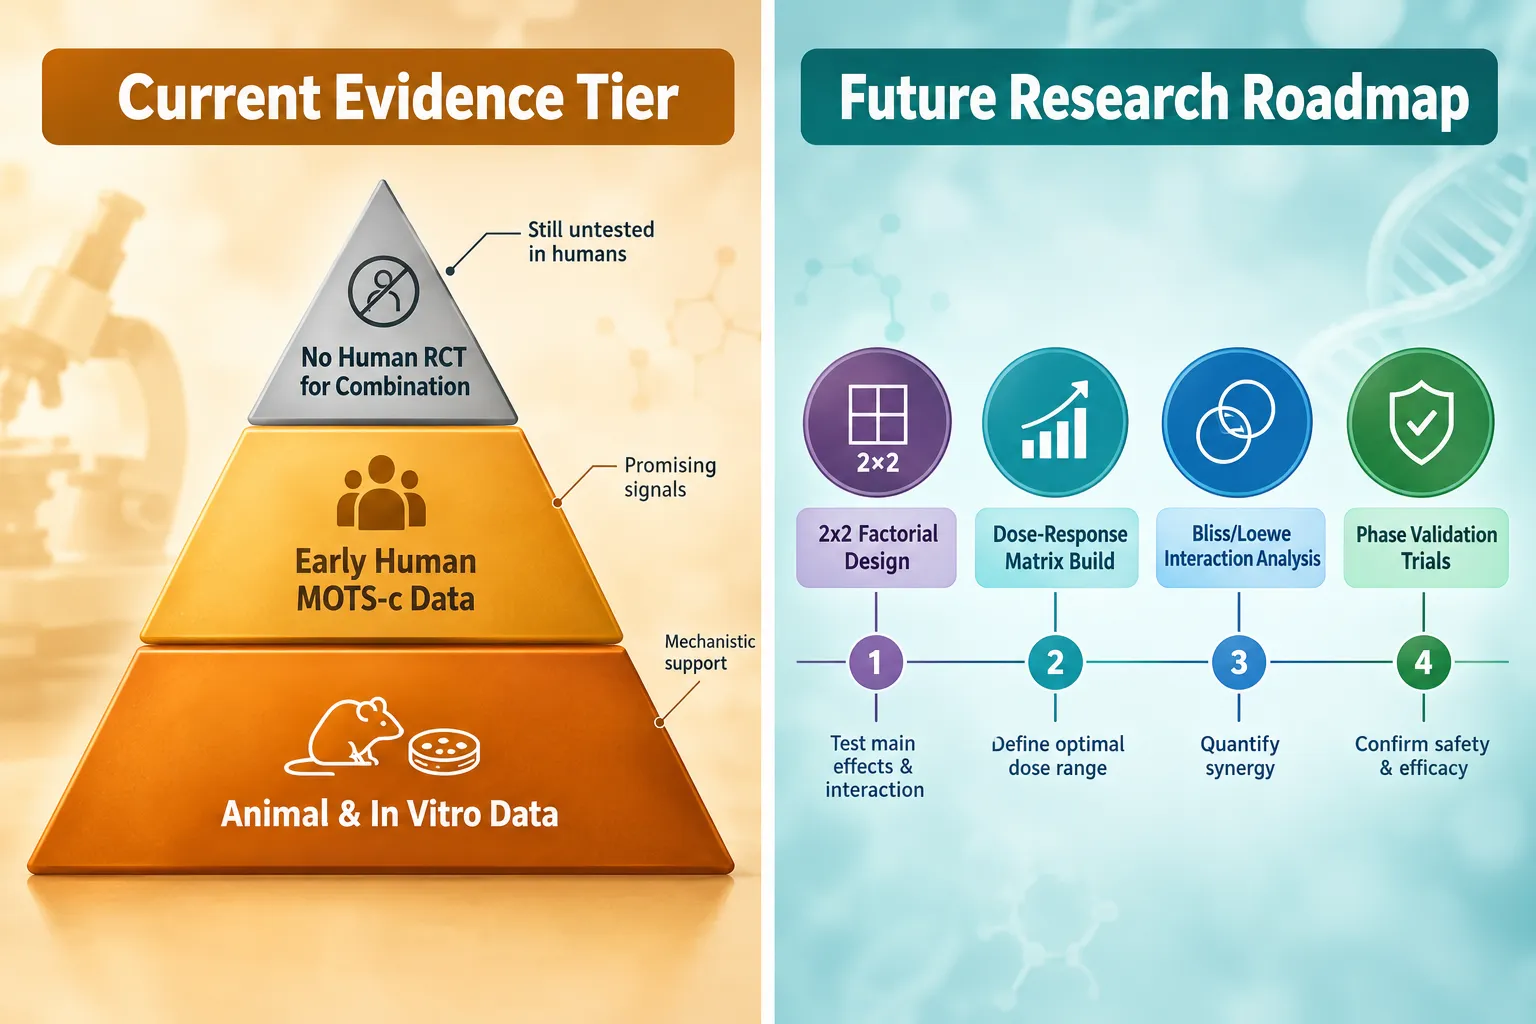
Preclinical data show that combining NNMT inhibition with mitochondrial peptide signaling can increase fat oxidation by roughly 47% above baseline, yet no published, peer-reviewed study has formally tested 5-Amino-1MQ and MOTS-c together in any model, human or animal. That gap between mechanistic promise and experimental evidence is precisely why a rigorous combination-study framework matters. Designing 5-Amino-1MQ and MOTS-c co-treatment: a matrix for dose-response, additivity, and interaction testing is not a dosing guide, it is a blueprint for generating credible data where none currently exists.

Key Takeaways

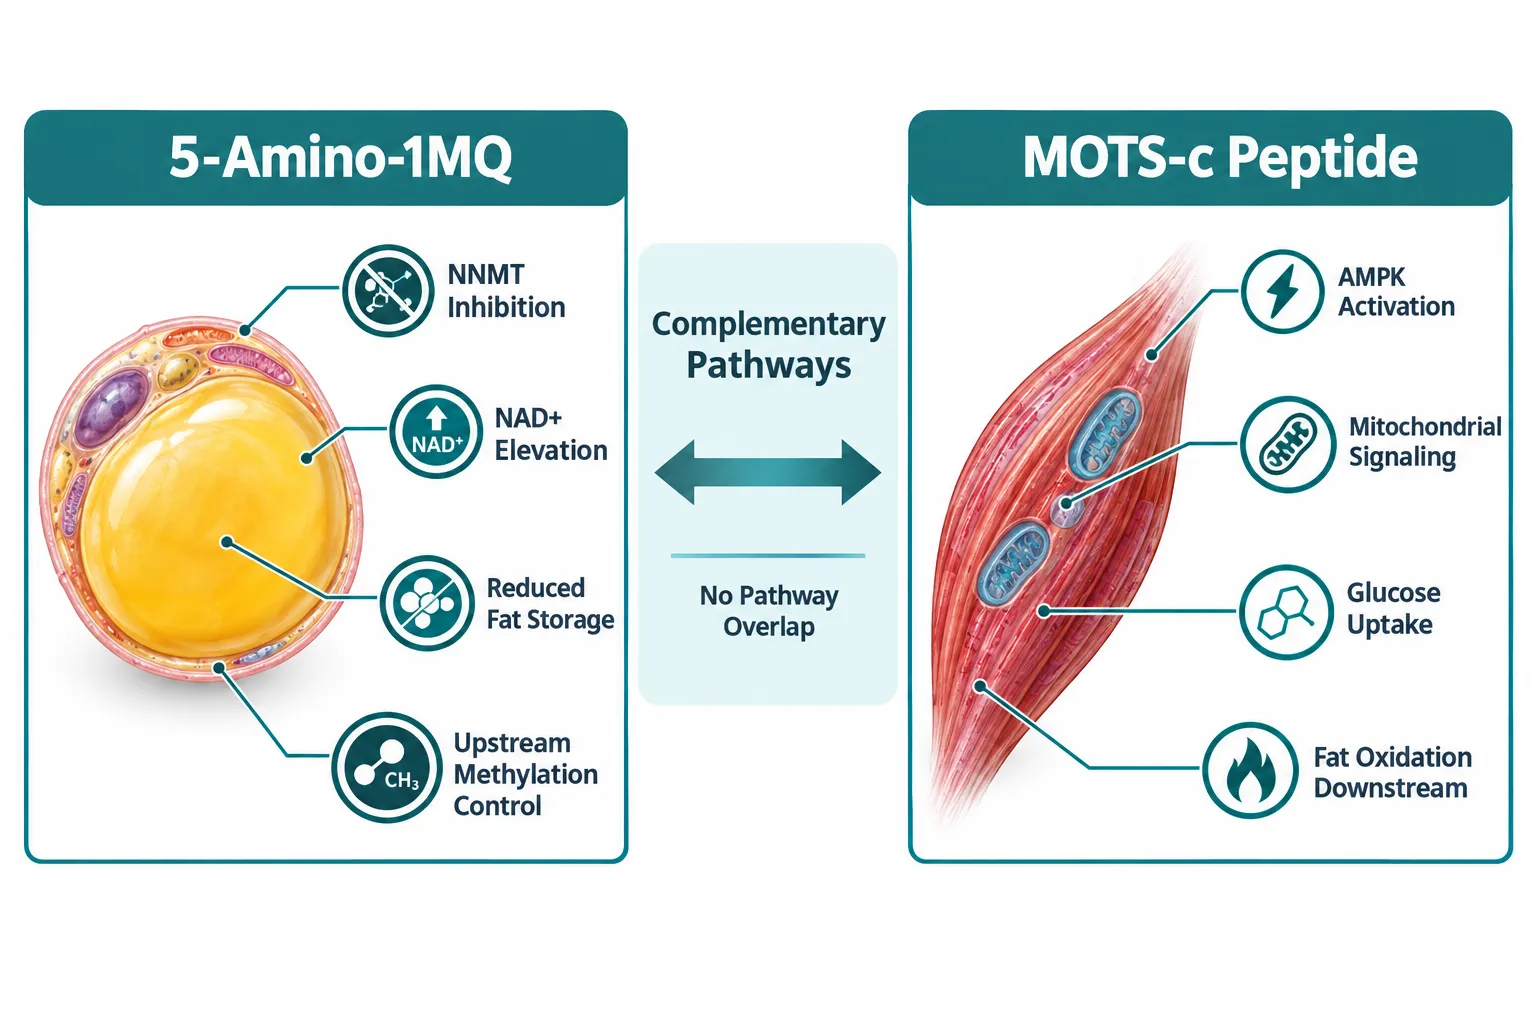
  • 5-Amino-1MQ inhibits NNMT and raises NAD+ in adipose tissue; MOTS-c activates AMPK in skeletal muscle, the pathways are complementary, not overlapping.
  • No published study has tested the two compounds together; any combination matrix is currently hypothetical experimental design, not completed research.
  • A 2×2 factorial layout (vehicle, each agent alone, combination) is the minimum structure needed to detect true interaction effects.
  • Bliss independence and Loewe additivity models are the standard analytical tools for quantifying whether a combination is additive, synergistic, or antagonistic.
  • Both compounds are sold for research use only; 5-Amino-1MQ has no registered human trials, while MOTS-c has limited early human mechanistic data.

Why These Two Compounds Belong in the Same Experimental Frame

Why These Two Compounds Belong in the Same Experimental Frame

Understanding the rationale for 5-Amino-1MQ and MOTS-c co-treatment begins with their distinct, non-overlapping mechanisms.

5-Amino-1MQ is a small-molecule inhibitor of nicotinamide N-methyltransferase (NNMT), an enzyme that consumes NAD+ precursors in white adipose tissue. By suppressing NNMT, the compound elevates intracellular NAD+ and alters methylation-dependent regulation of fat storage. In obese mouse models, it reduced body weight without changing food intake or lean mass, a profile that suggests a direct effect on adipose metabolism rather than appetite suppression. Researchers can explore 5-Amino-1MQ capsules as a reference-grade research compound.

MOTS-c is a 16-amino-acid peptide encoded in mitochondrial DNA. It activates AMPK and related metabolic stress pathways, primarily in skeletal muscle, enhancing glucose uptake and fat oxidation. Unlike 5-Amino-1MQ, MOTS-c has early human mechanistic data in metabolic and exercise contexts. Researchers can review MOTS-c and Elamipretide for context on mitochondrial-targeted peptide combinations.

The conceptual logic for pairing them is straightforward: 5-Amino-1MQ acts upstream on NNMT and NAD+ in white fat; MOTS-c acts downstream on mitochondrial signaling and AMPK in muscle. There is no obvious pathway competition, which creates a plausible, though unproven, basis for additivity or synergy.

"Mechanistic complementarity is a hypothesis, not a result. It justifies building a dose-response matrix; it does not replace one."


Building the Experimental Matrix: Factorial Design and Dose Selection

Building the Experimental Matrix: Factorial Design and Dose Selection

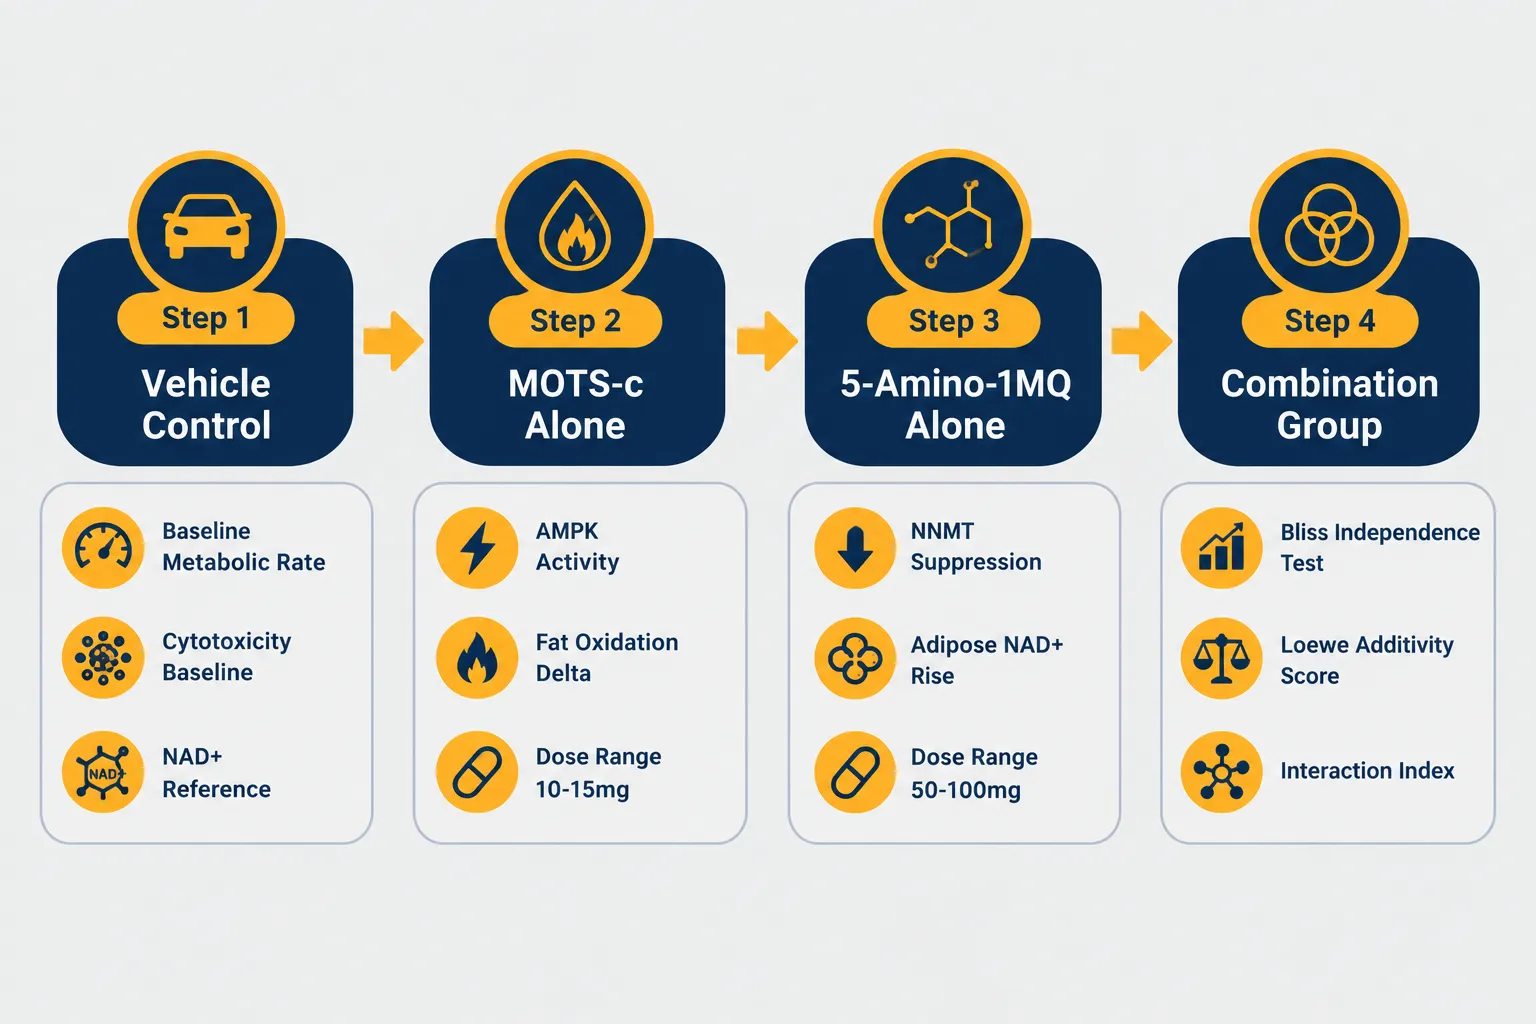
The foundation of 5-Amino-1MQ and MOTS-c co-treatment: a matrix for dose-response, additivity, and interaction testing is a properly structured factorial experiment. A 2×2 factorial layout, vehicle control, MOTS-c alone, 5-Amino-1MQ alone, and the combination, is the minimum design capable of detecting interaction effects. Anything less cannot distinguish true synergy from simple additive responses.

Dose Range Selection

Research-oriented protocols commonly reference the following ranges, extrapolated from animal and mechanistic data rather than large randomized human trials:

Compound Typical Research Range Route
5-Amino-1MQ 50-100 mg once daily Oral
MOTS-c 10-15 mg once daily Subcutaneous

For a proper dose-response matrix, each compound should be tested at a minimum of three concentration levels (low, mid, high) within these ranges. This produces a 3×3 grid of nine treatment conditions plus vehicle control, sufficient to fit a response surface and identify the concentration pair that maximizes effect while minimizing off-target risk.

Endpoints to Measure

A credible matrix requires mechanistic endpoints, not just body-weight readouts:

  • NAD+ and SAM pool quantification, both pathways influence NAD+ availability by different mechanisms, and their interaction on methyl donor pools is currently unknown
  • AMPK phosphorylation, primary downstream marker of MOTS-c activity
  • NNMT enzyme activity, direct measure of 5-Amino-1MQ target engagement
  • Mitochondrial oxygen consumption rate (OCR), Seahorse or equivalent assay
  • Cytotoxicity controls, cell viability at every dose level to separate metabolic effects from toxicity artifacts

Omitting cytotoxicity controls is a common methodological error in preclinical peptide research. Any apparent "synergy" in a metabolic endpoint is uninterpretable if cell viability is simultaneously compromised.


Interaction Analysis: Bliss, Loewe, and What the Data Actually Need to Show

Interaction Analysis: Bliss, Loewe, and What the Data Actually Need to Show

Once dose-response data are collected, the analytical framework determines whether the combination qualifies as additive, synergistic, or antagonistic. Two models dominate combination pharmacology:

Bliss Independence assumes that each agent acts independently. The expected combined effect is calculated as: E(A+B) = E(A) + E(B) − E(A)×E(B). If the observed effect exceeds this prediction, synergy is indicated; if it falls short, antagonism is present.

Loewe Additivity treats the two drugs as if they were dilutions of each other. It calculates a combination index (CI): CI < 1 indicates synergy, CI = 1 indicates additivity, CI > 1 indicates antagonism. Loewe is generally preferred when the two compounds share a common downstream endpoint, in this case, fat oxidation or AMPK activity.

For 5-Amino-1MQ and MOTS-c co-treatment: a matrix for dose-response, additivity, and interaction testing, researchers should apply both models and report where they agree and diverge. Discordance between Bliss and Loewe often signals that the mechanistic assumption of independence or dose-equivalence needs revision, itself a valuable finding.

A Critical Caution on NAD+ Interaction

Both compounds influence NAD+ availability, though by different mechanisms. 5-Amino-1MQ raises NAD+ by blocking its consumption via NNMT; MOTS-c influences NAD+-dependent AMPK signaling from the mitochondrial side. Whether co-administration amplifies NAD+ effects, creates redundancy, or produces unexpected depletion of shared methyl donor (SAM) pools is unknown. This interaction should be treated as an explicit hypothesis within the matrix, not an assumed benefit.

Multi-compound stacks that combine these agents with NAD+ precursors, some commercial vials contain approximately 10 mg 5-Amino-1MQ, 10 mg MOTS-c, and 100 mg NAD+, add a third variable that further complicates interaction modeling. Researchers interested in related mitochondrial peptide combinations can also review SS-31 and MOTS-c stacks for comparative mechanistic context.

When sourcing compounds for any in-vitro or animal study, purity verification is non-negotiable. Lab-tested peptides with documented certificate-of-analysis data are the baseline standard for credible preclinical work.


Conclusion

The scientific case for exploring 5-Amino-1MQ and MOTS-c co-treatment: a matrix for dose-response, additivity, and interaction testing rests on mechanistic complementarity, upstream NNMT inhibition in adipose tissue paired with downstream AMPK activation in skeletal muscle. That complementarity is conceptually sound, but it remains a hypothesis. No peer-reviewed study has yet tested this combination formally.

Actionable next steps for researchers:

  1. Design a 3×3 dose-response matrix with vehicle control and measure at least four mechanistic endpoints, including cytotoxicity at every concentration.
  2. Apply both Bliss independence and Loewe additivity models to the combination data; report the combination index and flag any discordance between models.
  3. Explicitly test NAD+ and SAM pool effects as a primary endpoint, not a secondary observation, this is the most likely site of unexpected interaction.
  4. Use only purity-verified, lab-tested compounds and document batch-level CoA data in any publication.
  5. Frame all findings as hypothesis-generating until Phase-grade human trial data exist; 5-Amino-1MQ remains entirely preclinical, and no human dose-response validation for either compound in combination has been registered.

The matrix described here does not yet exist in the literature. Building it rigorously is the work that needs to happen before any clinical extrapolation is warranted.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/5-amino-1mq-and-mots-c-co-treatment-a-matrix-for-dose-response-additivity-and-in.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-02 13:03:482026-10-02 13:03:485-Amino-1MQ and MOTS-c Co-Treatment: A Matrix for Dose-Response, Additivity, and Interaction Testing
MOTS-c and 5-Amino-1MQ: A Practical Guide to Separating Mitochondrial, NNMT, and Energy-Flux Readouts

MOTS-c and 5-Amino-1MQ: A Practical Guide to Separating Mitochondrial, NNMT, and Energy-Flux Readouts

October 1, 2026/0 Comments/in Uncategorized/by

Attributing an observed metabolic effect to the wrong mechanism is one of the most common errors in multi-compound research protocols. When two agents act on overlapping but distinct pathways, as MOTS-c and 5-Amino-1MQ do, a poorly designed assay panel can make a mitochondrial signal look like an NAD+ effect, or vice versa. This practical guide to MOTS-c and 5-Amino-1MQ covers how to separate mitochondrial, NNMT, and energy-flux readouts so that each intervention gets credited for what it actually does.

Key Takeaways

  • MOTS-c is a mitochondrial-derived peptide that activates AMPK primarily in skeletal muscle, driving glucose uptake and fatty-acid oxidation.
  • 5-Amino-1MQ inhibits NNMT, preserving the intracellular NAD+ pool and activating sirtuin-linked pathways mainly in white adipose tissue and liver.
  • Both compounds can influence NAD+ levels, but through mechanistically different routes that require distinct assays to distinguish.
  • A well-designed study pairs mitochondrial respiration assays, NAD-related measurements, NNMT-linked markers, ATP quantification, and cell-viability controls in the same protocol.
  • The evidence base for both agents remains preclinical; neither is an approved therapeutic.

Understanding the Two Pathways Before Designing Any Assay

Understanding the Two Pathways Before Designing Any Assay

Any practical guide to MOTS-c and 5-Amino-1MQ must begin with a clear picture of what each compound does independently. Confusing their mechanisms at the design stage leads to assay panels that cannot answer the questions being asked.

MOTS-c is a 16-amino-acid peptide encoded within mitochondrial DNA, first characterized by a University of Southern California research group in 2015. It interferes with the folate-methionine one-carbon cycle and de novo purine biosynthesis inside cells, causing AICAR to accumulate. AICAR is a well-established indirect activator of AMP-activated protein kinase (AMPK). The downstream result is increased fatty-acid oxidation, enhanced GLUT4-mediated glucose uptake, and improved insulin sensitivity, effects observed most strongly in skeletal muscle in animal models. Animal studies have shown prevention of diet-induced obesity and age-related insulin resistance.

Researchers interested in MOTS-c peptide research materials should note that its primary readout territory is mitochondrial bioenergetics and substrate oxidation, not direct NAD+ salvage.

5-Amino-1MQ (5-amino-1-methylquinolinium) is a small, membrane-permeable molecule that directly inhibits nicotinamide N-methyltransferase (NNMT). NNMT converts nicotinamide to 1-methylnicotinamide, consuming S-adenosylmethionine (SAM) in the process. By blocking this enzyme, 5-Amino-1MQ reduces SAM consumption, preserves the intracellular NAD+ pool, and activates NAD+-dependent pathways including sirtuins and mitochondrial biogenesis. Preclinical mouse data have shown reductions in fat mass without reduced food intake. Its primary action zone is white adipose tissue and liver, where NNMT is upregulated in obesity.

"Both compounds can nudge NAD+ levels upward, but they pull different levers to get there, and conflating those levers produces uninterpretable data."

This mechanistic divergence is exactly why a guide to separating mitochondrial, NNMT, and energy-flux readouts is necessary before any combined protocol begins.


How to Separate Mitochondrial, NNMT, and Energy-Flux Readouts in Practice

How to Separate Mitochondrial, NNMT, and Energy-Flux Readouts in Practice

The core design principle is simple: assign each readout category its own assay layer, and run all three layers in the same experimental unit so that confounding is controlled rather than ignored.

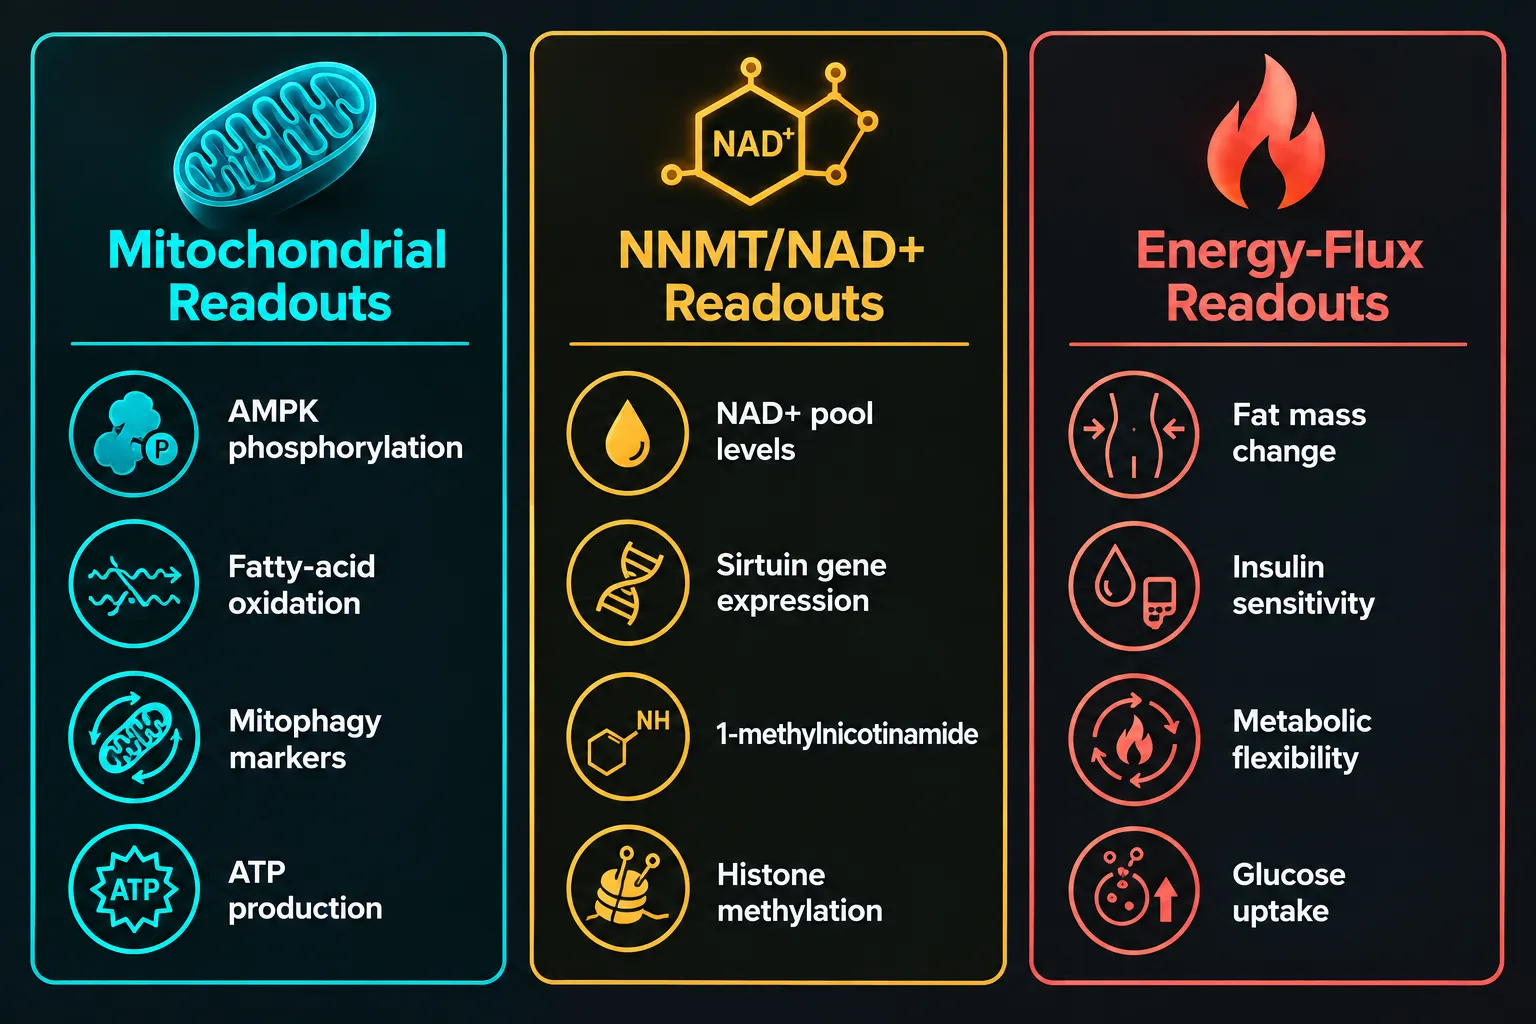
Mitochondrial Readouts

These assays capture AMPK-centric activity attributable to MOTS-c.

Readout Recommended Assay What It Captures
AMPK activation Western blot for p-AMPK/AMPK ratio Direct MOTS-c downstream signal
Oxygen consumption rate (OCR) Seahorse XF Analyzer Mitochondrial respiration flux
Fatty-acid oxidation Radiolabeled palmitate oxidation Substrate shift toward lipids
Mitophagy/biogenesis LC3-II, PGC-1alpha expression Mitochondrial quality control

NNMT and NAD+ Readouts

These assays isolate the 5-Amino-1MQ contribution.

  • NAD+/NADH ratio: A direct readout of NAD+ pool preservation. If 5-Amino-1MQ is working, this ratio rises without a proportional change in NAMPT activity.
  • 1-methylnicotinamide (MNA) levels: MNA is the product of NNMT activity. Reduced MNA confirms NNMT inhibition, not just a generic NAD+ boost.
  • SAM/SAH ratio: Reflects the methylation economy downstream of NNMT blockade.
  • Sirtuin-linked gene expression: SIRT1 and SIRT3 targets confirm NAD+-dependent pathway activation.

Critically, if MOTS-c is present in the same well and AMPK is active, NAD+ consumption will increase through energy-demanding pathways. That can mask 5-Amino-1MQ's preserving effect. Measuring MNA and SAM/SAH alongside NAD+/NADH disambiguates the source.

Energy-Flux Readouts

These whole-system markers capture the integrated output of both interventions.

  • Fat mass change (in animal models): Reflects combined lipolytic and oxidative effects.
  • Insulin sensitivity: Glucose tolerance tests and HOMA-IR scores capture GLUT4-mediated improvements driven by MOTS-c.
  • Metabolic flexibility: The ability to switch between glucose and fat oxidation, measurable via respiratory exchange ratio (RER).
  • ATP quantification: Total cellular ATP reflects the net energy-production outcome and serves as a cross-check on both mitochondrial respiration and NAD+ pathway activity.

For context on how other mitochondrial-targeting peptides are studied, the SS-31 mitochondrial research themes resource illustrates how cardiolipin-targeted agents use similar OCR-based designs, offering useful methodological parallels. Additional background on SS-31 elamipretide research approaches can inform how to structure mitochondrial membrane integrity controls.


Building an Attribution-Proof Protocol: Step-by-Step

Building an Attribution-Proof Protocol: Step-by-Step

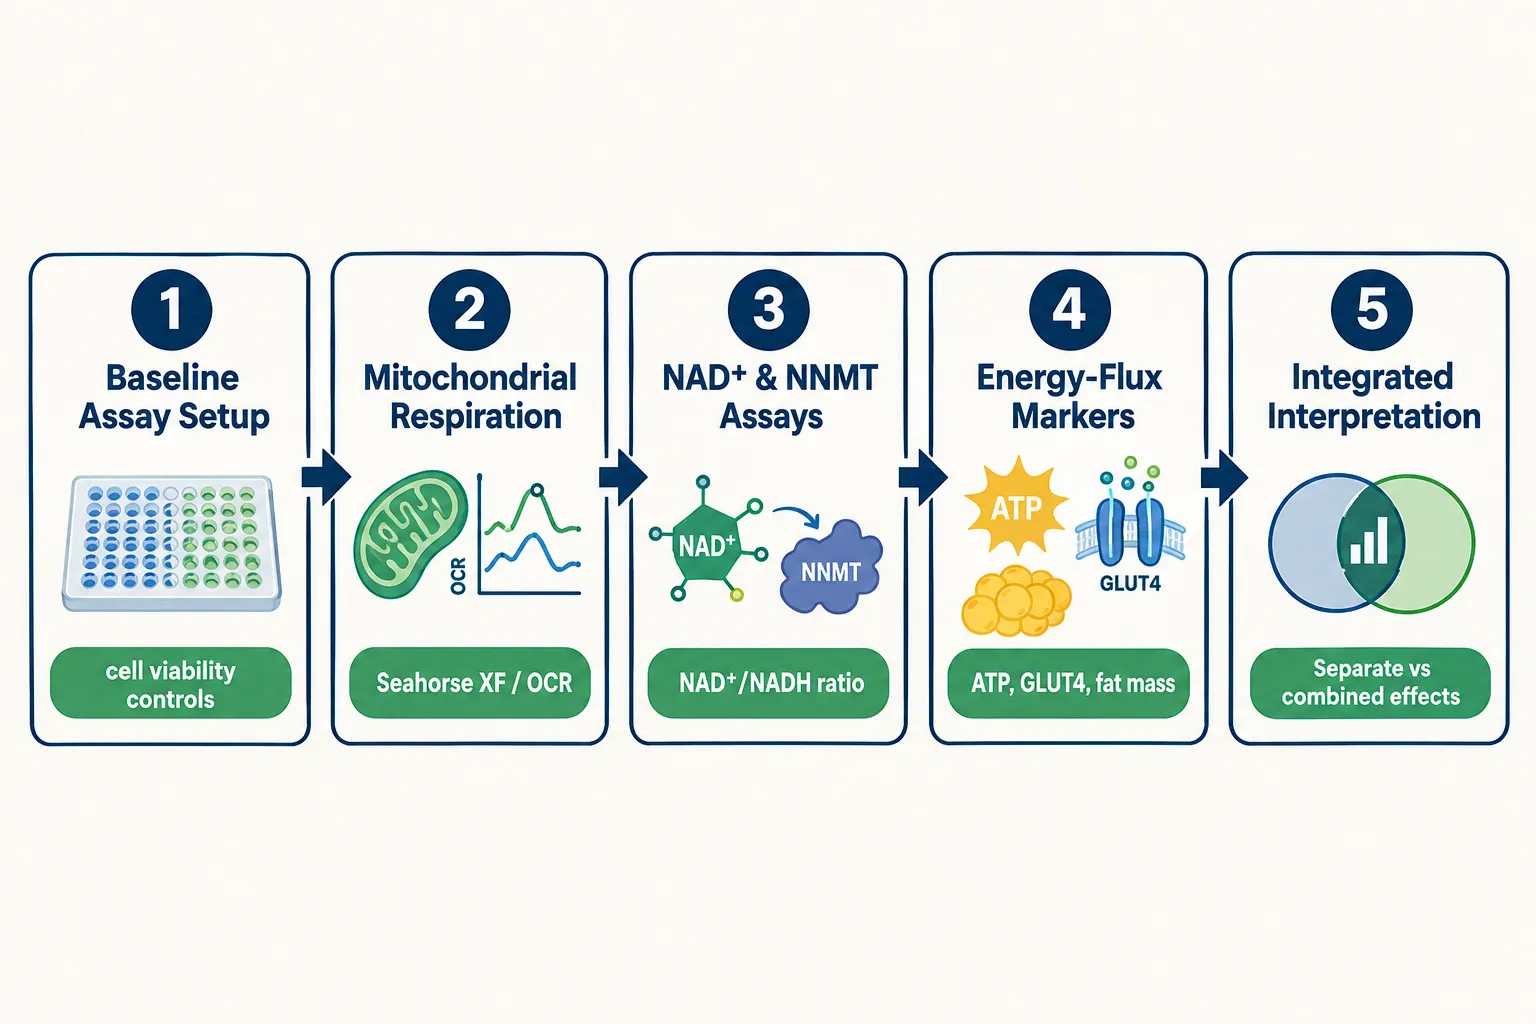
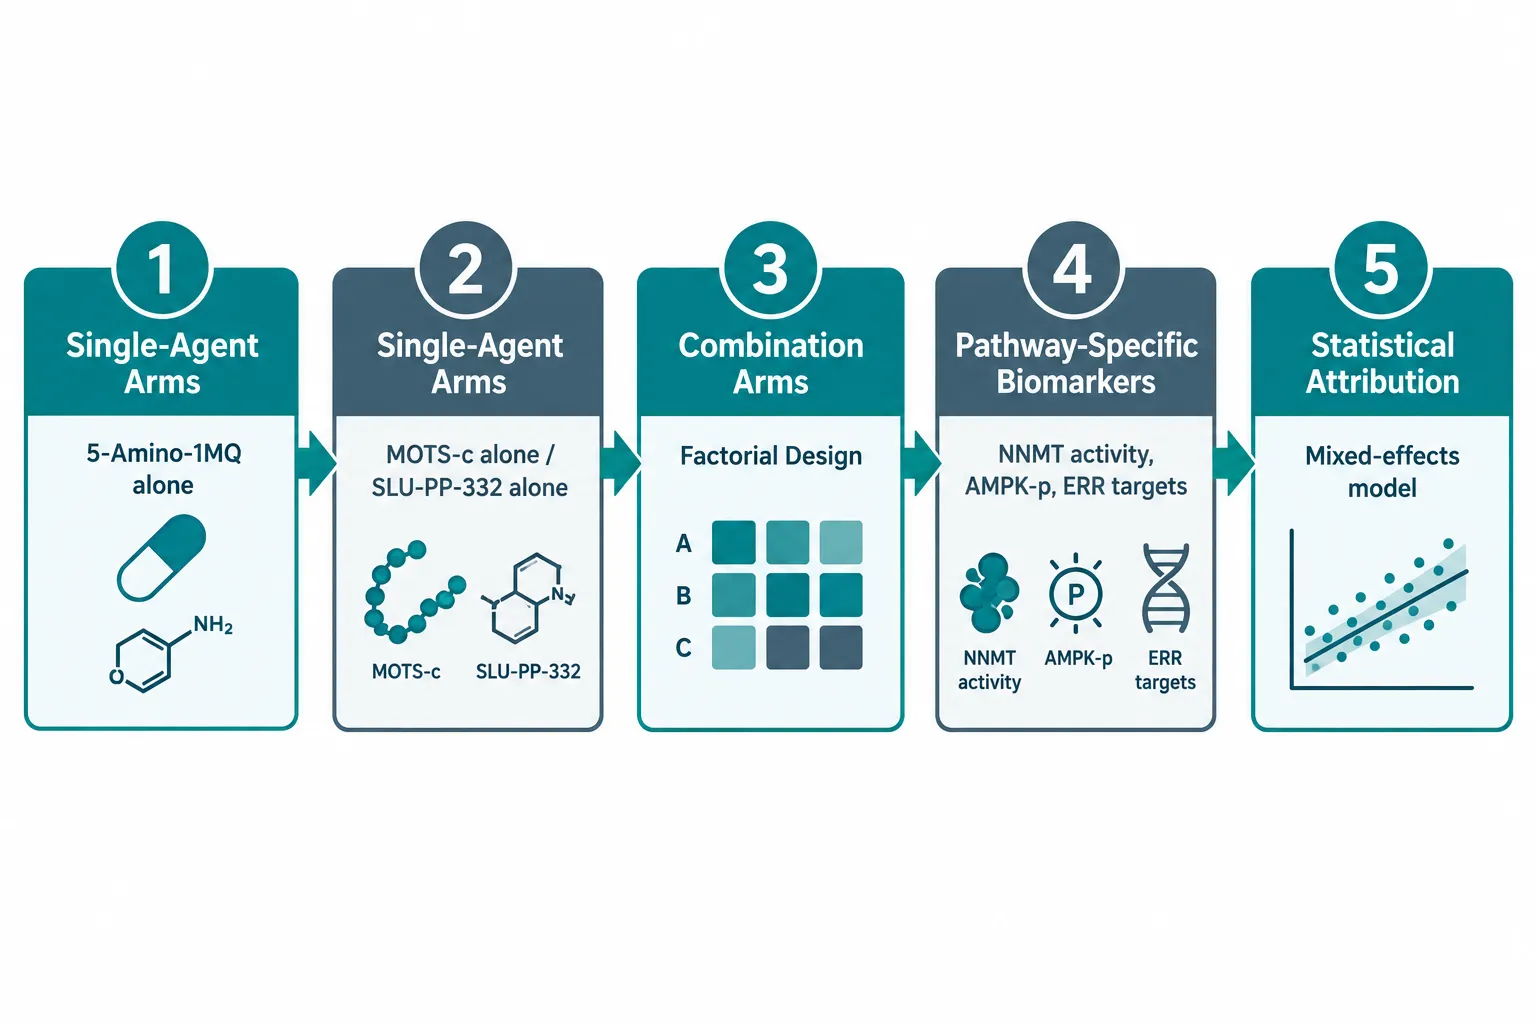
The following five-step framework minimizes attribution error when running MOTS-c and 5-Amino-1MQ together.

Step 1, Establish baseline cell viability controls. Run MTT or CellTiter-Glo assays at every dose tested. If viability drops, any observed change in OCR or NAD+ is a toxicity artifact, not a mechanism signal.

Step 2, Run single-agent arms first. Before combining, characterize each compound alone. This produces a mechanistic fingerprint: MOTS-c alone should shift OCR and raise p-AMPK; 5-Amino-1MQ alone should lower MNA and raise the NAD+/NADH ratio.

Step 3, Apply the full assay panel to the combination arm. All readouts from Steps 1 and 2 must be measured simultaneously. Partial panels in the combination arm are the primary source of attribution errors.

Step 4, Use pathway inhibitors as mechanistic controls. An AMPK inhibitor (such as Compound C) can silence the MOTS-c arm pharmacologically, allowing the NNMT signal to be read in isolation within the same combined-treatment context. An NNMT-overexpression control does the reverse.

Step 5, Interpret energy-flux markers last. Fat mass, insulin sensitivity, and ATP changes are downstream integrations of both pathways. They should be interpreted only after the upstream mitochondrial and NNMT readouts have been attributed.

For researchers also exploring growth-hormone-mediated metabolic comparisons, reviewing how peptides in cardiometabolic models differ from small-molecule drugs provides useful framing for why AMPK agonists, NNMT inhibitors, and GH-driven agents require separate readout categories. Similarly, understanding visceral fat research methodology helps contextualize fat-mass endpoints.


Conclusion

A practical guide to MOTS-c and 5-Amino-1MQ separating mitochondrial, NNMT, and energy-flux readouts comes down to one discipline: never let overlapping downstream effects collapse distinct upstream mechanisms into a single unattributed signal.

Actionable next steps for researchers:

  1. Map each compound to its primary assay layer before designing the protocol.
  2. Always include MNA quantification alongside NAD+/NADH to distinguish NNMT inhibition from AMPK-driven NAD+ consumption.
  3. Run single-agent arms before the combination arm to establish mechanistic fingerprints.
  4. Include cell-viability controls at every dose and time point.
  5. Reserve energy-flux endpoints (fat mass, insulin sensitivity, ATP) for last-stage interpretation, not primary attribution.

Both MOTS-c and 5-Amino-1MQ remain research-stage compounds with a predominantly preclinical evidence base. No large, controlled human trials have confirmed the animal findings, and neither agent is an approved drug. All protocols should be conducted within appropriate research frameworks and regulatory guidelines.

https://www.puretestedpeptides.com/wp-content/uploads/2026/10/mots-c-and-5-amino-1mq-a-practical-guide-to-separating-mitochondrial-nnmt-and-en.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-10-01 13:04:082026-10-01 13:04:08MOTS-c and 5-Amino-1MQ: A Practical Guide to Separating Mitochondrial, NNMT, and Energy-Flux Readouts
What Is Slupp332 With 5-Amino-1MQ? Research Context, Naming Confusion, and Potential Metabolic Relevance

What Is Slupp332 With 5-Amino-1MQ? Research Context, Naming Confusion, and Potential Metabolic Relevance

September 29, 2026/0 Comments/in Uncategorized/by

A single search for "Slupp332 with 5-Amino-1MQ" returns product pages, research forums, and peptide vendor catalogs that use the term in completely different ways. For researchers and clinicians trying to parse the science, that inconsistency is a real problem. Understanding what is Slupp332 with 5-Amino-1MQ, including the research context, naming confusion, and potential metabolic relevance, requires separating two distinct compounds that are often sold together but work through entirely different biological mechanisms.

Key Takeaways

  • "Slupp332" is an informal spelling of SLU-PP-332, a beta-3 adrenergic receptor agonist studied as an exercise mimetic in preclinical models.
  • 5-Amino-1MQ (5-amino-1-methylquinolinium) is a separate small-molecule inhibitor of the enzyme NNMT, studied for its role in NAD+ preservation and fat metabolism.
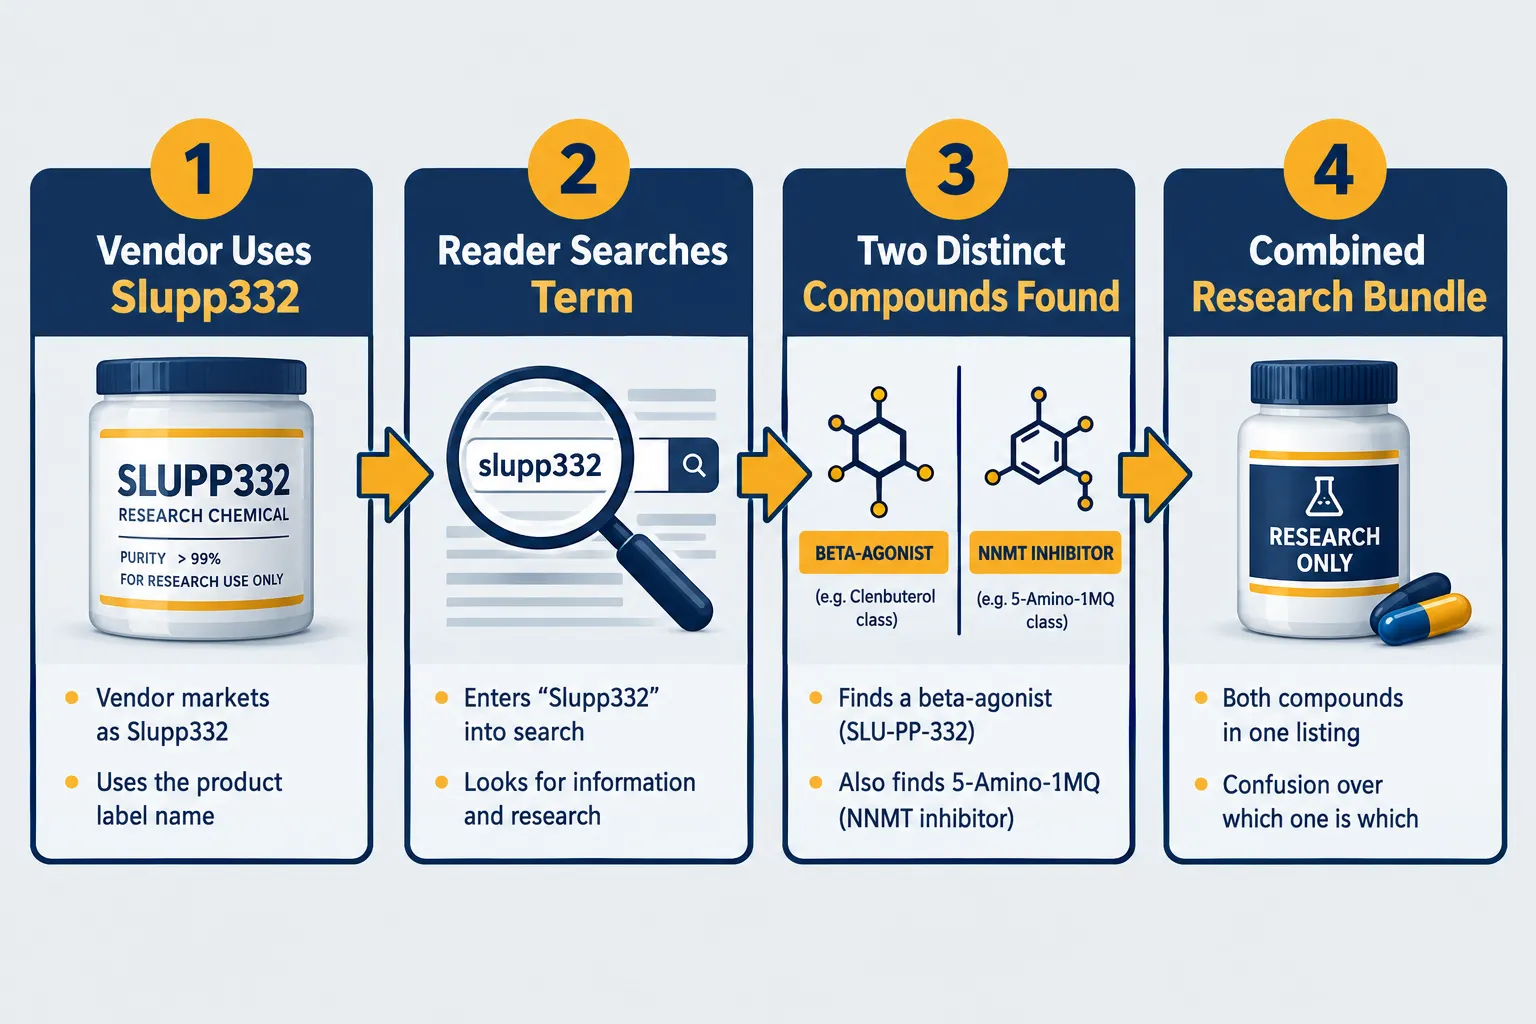
  • The two compounds are sold together in research bundles but are not the same substance and do not share a mechanism of action.
  • Naming inconsistencies across vendor pages, "SLUPP-332," "SLU-PP-332," "Slupp332", are a primary source of confusion for researchers.
  • As of 2026, both compounds remain investigational, with no approved clinical indications and no large-scale human outcome data.

Decoding the Naming Confusion Around Slupp332 and 5-Amino-1MQ

The term "Slupp332" is not a standardized chemical name. It is a vendor-simplified version of SLU-PP-332, a compound developed in academic pharmacology research. Across supplier catalogs, it appears as "SLU-PP-332," "SLUPP-332," "Slupp-332," and "Slupp332", all referring to the same molecule. This inconsistency is not trivial. A researcher unfamiliar with the compound might assume these are different substances or mistake the informal name for a peptide blend.

Decoding the Naming Confusion Around Slupp332 and 5-Amino-1MQ

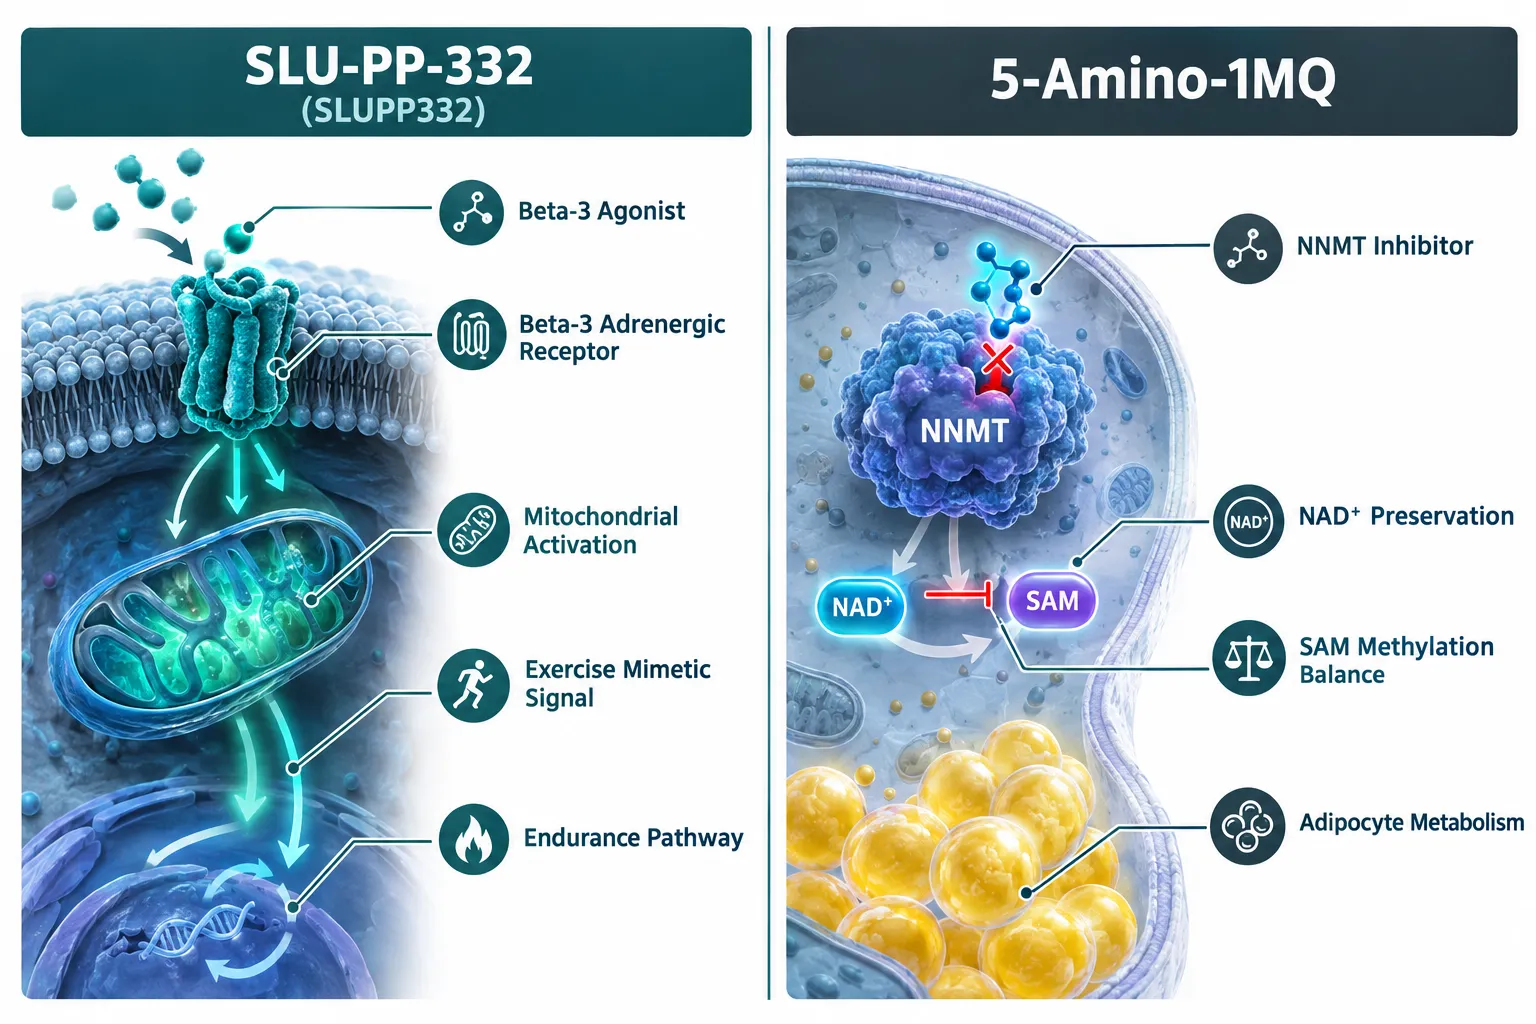
SLU-PP-332 is a beta-3 adrenergic receptor agonist. Its research interest centers on its potential to mimic some physiological effects of exercise, specifically, activating pathways linked to mitochondrial biogenesis and endurance adaptation, without physical activity. In research bundles, it typically appears at 250 mcg per capsule, explicitly labeled for laboratory research only.

5-Amino-1MQ (full name: 5-amino-1-methylquinolinium) is an entirely different class of compound. It is a small-molecule, membrane-permeable inhibitor of nicotinamide N-methyltransferase (NNMT), the enzyme responsible for methylating nicotinamide using S-adenosyl methionine (SAM). When NNMT is active, it diverts nicotinamide away from the NAD+ salvage pathway. By blocking NNMT, 5-Amino-1MQ preserves nicotinamide for NAD+ synthesis, which may support cellular energy metabolism, particularly in metabolically aged or obese tissue.

To explore the broader landscape of small molecules and peptides in this research space, the Peptides 101 for Research-Use Only Buyers guide provides useful structural and mechanistic context.


Research Context: What Each Compound Does Separately

SLU-PP-332 as an Exercise Mimetic

SLU-PP-332 targets the beta-3 adrenergic receptor, a G-protein-coupled receptor expressed primarily in adipose tissue and, to a lesser extent, in skeletal muscle. Activation of this receptor triggers downstream signaling associated with:

  • Mitochondrial activation and increased oxidative capacity
  • Enhanced fat oxidation in adipose depots
  • Endurance-related gene expression changes

Preclinical research has described these effects as "exercise mimetic," meaning the compound may activate some of the same cellular programs that physical training does. This positions SLU-PP-332 alongside other compounds studied for visceral fat research and metabolic optimization in animal models.

5-Amino-1MQ as an NNMT Inhibitor

5-Amino-1MQ's mechanism is rooted in methylation biochemistry. Preclinical work in differentiated adipocytes demonstrated that exposing cells to 0.3-60 µM of 5-Amino-1MQ over 24 hours reduces intracellular NNMT activity and alters levels of NAD+, nicotinic acid, SAM, and S-adenosylhomocysteine (SAH). These changes support a direct role in both cellular energy metabolism and epigenetic regulation of metabolic genes.

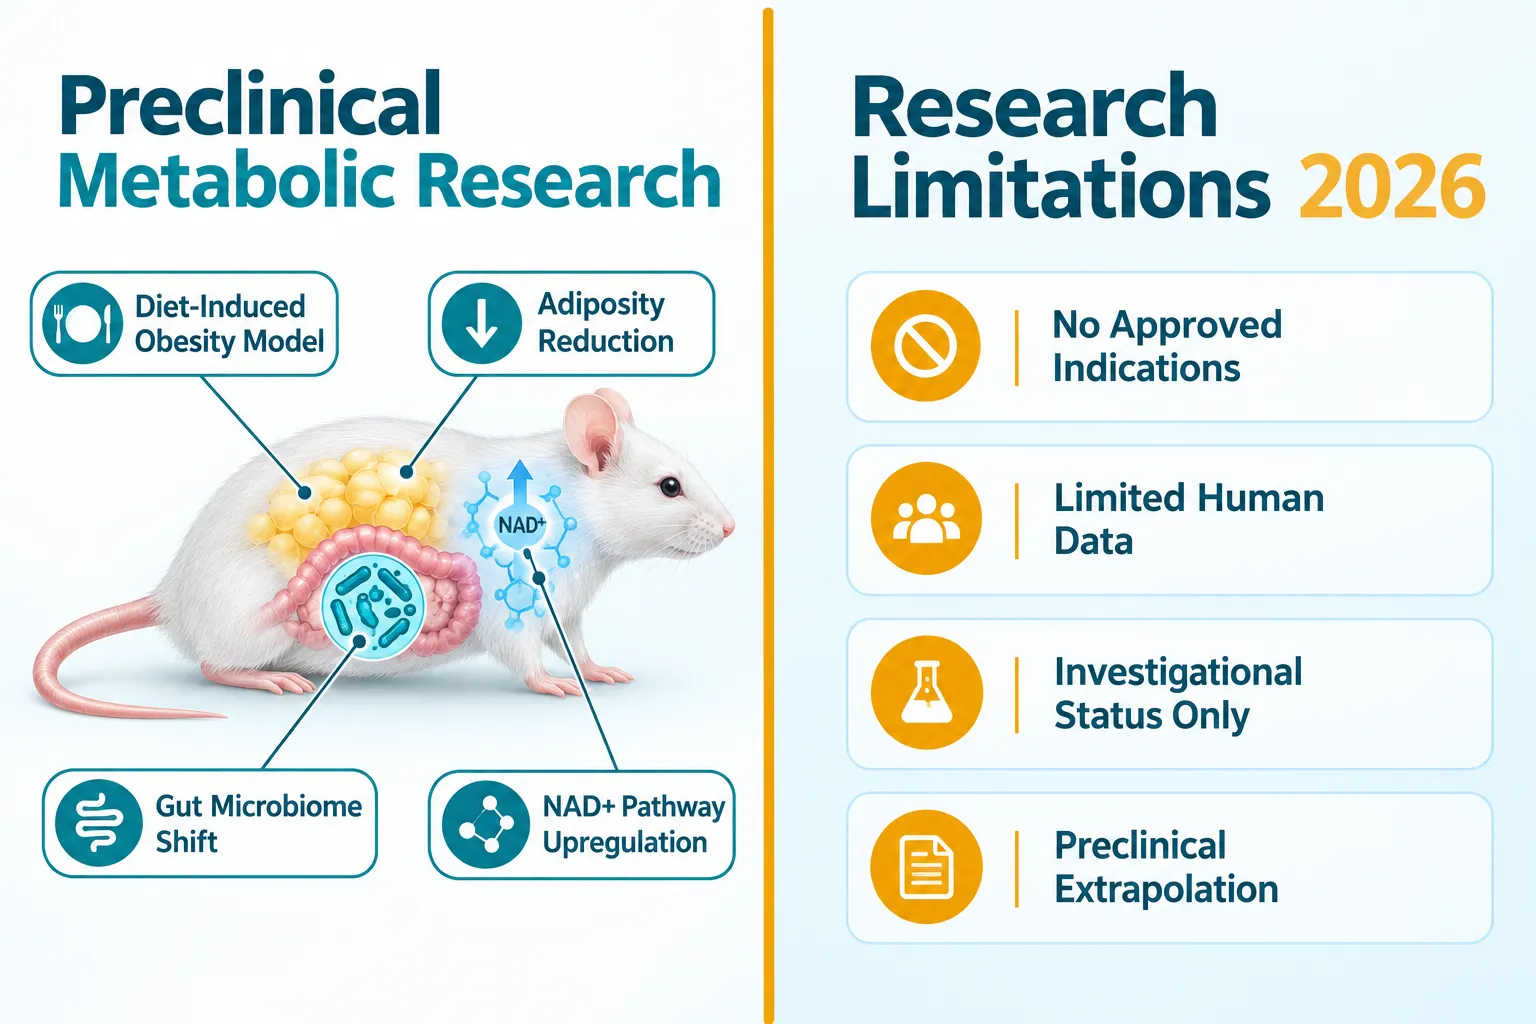
A 2022 study in Scientific Reports reported that combining an NNMT inhibitor with a reduced-calorie, low-fat diet in diet-induced obese mice produced rapid adiposity and weight loss, normalizing measures to lean controls faster than diet alone, while also shifting the gut microbiome to a distinct profile.

Pharmacokinetic data from rat studies show an oral bioavailability of approximately 38.4% for 5-Amino-1MQ, with a mean terminal half-life of 3.80 hours after intravenous administration and 6.90 hours after oral dosing. These parameters are foundational for designing future exposure models.

Researchers interested in 5-Amino-1MQ capsules for preclinical study can find research-grade formulations through specialized suppliers.


Potential Metabolic Relevance of the Slupp332 + 5-Amino-1MQ Combination

The pairing of these two compounds in research bundles is not arbitrary. Vendors and research guides describe the combination as a framework for interrogating fat oxidation, energy regulation, glucose control, and cellular health within the same experimental design.

Potential Metabolic Relevance of the Slupp332 + 5-Amino-1MQ Combination

The rationale is mechanistically complementary:

Compound Mechanism Research Target
SLU-PP-332 Beta-3 adrenergic agonism Mitochondrial activation, fat oxidation
5-Amino-1MQ NNMT inhibition NAD+ preservation, adipocyte size reduction

By combining beta-3 adrenergic signaling with NNMT inhibition, researchers can study whether activating exercise-mimetic pathways while simultaneously preserving NAD+ produces additive or synergistic effects on metabolic parameters. This dual approach is part of a broader trend in 2026 research positioning compounds as longevity-oriented metabolic modulators.

"The combination is hypothesis-generating, not clinically validated, a distinction that matters enormously when evaluating preclinical data."

For context on related mitochondrial research compounds studied alongside metabolic modulators, see SS-31 mitochondrial research themes and the SS-31 mitochondrial research tag.


Current Limitations and Regulatory Status

Current Limitations and Regulatory Status

Despite promising animal data, several important limitations apply to both compounds as of 2026:

  • No approved indications exist for SLU-PP-332 or 5-Amino-1MQ from any major regulatory agency.
  • Human clinical evidence is extremely limited. At least one 2026 clinical-trial summary explicitly frames 5-Amino-1MQ as experimental, with no large peer-reviewed human outcome data available.
  • All research-grade products are sold for laboratory use only and are not intended for human consumption.
  • Claims about obesity, diabetes, or longevity benefits remain extrapolated from preclinical models and should be treated as hypothesis-generating.

Authoritative guidance remains confined to basic-science NNMT and adrenergic-signaling literature. Any therapeutic application would be speculative and off-label.


Conclusion

The question of what is Slupp332 with 5-Amino-1MQ, including the research context, naming confusion, and potential metabolic relevance, has a clear answer once the terminology is untangled. "Slupp332" is an informal rendering of SLU-PP-332, a beta-3 adrenergic receptor agonist. 5-Amino-1MQ is a separate NNMT inhibitor. They are distinct compounds with different mechanisms that vendors bundle together for complementary preclinical research into fat metabolism, mitochondrial function, and NAD+ biology.

Actionable next steps for researchers:

  1. Always verify the formal chemical name (SLU-PP-332, not "Slupp332") when sourcing compounds to avoid cross-contamination of data.
  2. Treat preclinical findings as hypothesis-generating only; design studies with appropriate controls before extrapolating to metabolic outcomes.
  3. Review pharmacokinetic parameters (bioavailability, half-life) before selecting dosing intervals in animal models.
  4. Monitor regulatory updates in 2026 and beyond, as the investigational status of both compounds may evolve as human trial data accumulates.

For researchers exploring adjacent compounds in metabolic and peptide science, the IPA Sermorelin stack research overview offers additional context on how stacked research compounds are evaluated in preclinical frameworks.

https://www.puretestedpeptides.com/wp-content/uploads/2026/09/what-is-slupp332-with-5-amino-1mq-research-context-naming-confusion-and-potentia.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-09-29 13:03:422026-09-29 13:03:42What Is Slupp332 With 5-Amino-1MQ? Research Context, Naming Confusion, and Potential Metabolic Relevance
5-Amino-1MQ Research Assays: How NNMT-Related Readouts Can Be Separated From MOTS-c and SLU-PP-332 Effects

5-Amino-1MQ Research Assays: How NNMT-Related Readouts Can Be Separated From MOTS-c and SLU-PP-332 Effects

September 25, 2026/0 Comments/in Uncategorized/by

Three metabolically active compounds, 5-Amino-1MQ, MOTS-c, and SLU-PP-332, each touch mitochondrial energy metabolism, yet they do so through entirely different molecular mechanisms. When researchers design experiments involving more than one of these agents, conflated readouts are a genuine risk. Understanding the 5-Amino-1MQ research assays framework, specifically how NNMT-related readouts can be separated from MOTS-c and SLU-PP-332 effects, is essential for generating interpretable, publication-quality preclinical data.

Key Takeaways

  • 5-Amino-1MQ is a substrate-competitive NNMT inhibitor; its primary assay endpoints are NNMT enzyme activity, 1-methylnicotinamide (1-MNA) levels, and NAD+/SAM pool dynamics.
  • MOTS-c signals through AMPK phosphorylation and one-carbon metabolism remodeling, pathways that are mechanistically orthogonal to NNMT inhibition.
  • SLU-PP-332 activates estrogen-related receptors (ERRs) to drive transcriptional programs for mitochondrial biogenesis, a downstream node distinct from NNMT substrate competition.
  • Factorial experimental designs with single-agent control arms are the most reliable way to attribute effects to each compound.
  • As of 2026, all available efficacy data for 5-Amino-1MQ remain preclinical; no human trials have been published.

Understanding the NNMT Pathway: The Biochemical Basis of 5-Amino-1MQ Assays

Understanding the NNMT Pathway: The Biochemical Basis of 5-Amino-1MQ Assays

5-Amino-1MQ is a cell-permeable quinolinium salt that competitively inhibits nicotinamide N-methyltransferase (NNMT) at the nicotinamide binding site. NNMT normally consumes S-adenosylmethionine (SAM) to methylate nicotinamide, producing 1-MNA. By blocking this reaction, 5-Amino-1MQ preserves SAM and redirects nicotinamide back into the NAD+ salvage pathway. Reported in vitro data place the IC50 for human NNMT at approximately 1.2 µM, with cellular models showing 1.2-1.6-fold increases in intracellular NAD+.

The most cited preclinical evidence comes from a 2018 mouse study in which 20 mg/kg administered for 11 days reversed diet-induced obesity without reducing food intake, a result attributed to NNMT inhibition shifting adipose tissue toward fat oxidation. More recently, aged-mouse data published in 2026 showed that 5-Amino-1MQ combined with exercise improved grip strength beyond exercise alone, extending the compound's assay relevance into sarcopenia-like models.

Primary NNMT-centric assay endpoints to track:

Endpoint What It Measures Why It Is NNMT-Specific
NNMT enzyme activity Catalytic rate of nicotinamide methylation Direct measure of inhibitor engagement
1-MNA concentration Product of NNMT reaction Falls with effective inhibition
Nicotinamide pool Substrate availability Rises as NNMT is blocked
SAM/SAH ratio Methyl-donor status Increases when NNMT is not consuming SAM
NAD+ salvage flux Isotope-traced NAD+ synthesis Rises as nicotinamide is redirected

These endpoints are naturally separable from MOTS-c and SLU-PP-332 readouts because neither of those agents directly modulates NNMT catalytic activity or 1-MNA output. For researchers sourcing the compound, exploring the 5-amino peptide product category provides context on purity specifications and research-use designations relevant to assay planning.


Mapping the Mechanistic Differences: MOTS-c and SLU-PP-332 Versus NNMT Inhibition

Mapping the Mechanistic Differences: MOTS-c and SLU-PP-332 Versus NNMT Inhibition

The core challenge in multi-agent metabolic research is that MOTS-c, SLU-PP-332, and 5-Amino-1MQ all converge on mitochondrial energy output, but at entirely different upstream nodes.

MOTS-c: AMPK Signaling and One-Carbon Metabolism

MOTS-c is a mitochondria-encoded peptide that activates AMP-activated protein kinase (AMPK) and remodels folate and one-carbon metabolism. Its downstream effects include phosphorylation of ACC (acetyl-CoA carboxylase) and activation of stress-response transcriptional programs. These readouts are mechanistically orthogonal to substrate-competitive NNMT inhibition.

MOTS-c-specific assay markers:

  • AMPK phosphorylation (Thr172)
  • Downstream ACC activity
  • Folate cycle intermediates
  • Stress-response gene expression panels

Researchers pairing MOTS-c with 5-Amino-1MQ, a combination studied alongside related mitochondrial peptides, as discussed in resources on SS31 and MOTS-c research applications, should reserve AMPK phosphorylation readouts exclusively for MOTS-c attribution. Changes in 1-MNA or SAM pools should not be attributed to MOTS-c exposure.

SLU-PP-332: ERR Agonism and Transcriptional Biogenesis

SLU-PP-332 is a pan-ERR (estrogen-related receptor) agonist studied for its exercise-mimetic and mitochondrial biogenesis effects. It drives transcriptional programs through ERR target genes and PGC-1alpha-linked pathways, increasing mitochondrial DNA copy number and oxidative capacity. No published animal or human studies of SLU-PP-332 combined with 5-Amino-1MQ existed as of mid-2026.

"NNMT inhibition increases NAD+/SAM upstream, while ERR agonism drives downstream transcription of oxidative-metabolism genes, these are distinct nodes, not redundant ones."

SLU-PP-332-specific assay markers:

  • ERR target gene expression (ESRRA, ESRRB, ESRRG)
  • PGC-1alpha mRNA and protein levels
  • Mitochondrial DNA copy number
  • Oxygen consumption rate (as an ERR-driven output)

Conceptual analyses in 2026 explicitly frame any combined use of SLU-PP-332 and 5-Amino-1MQ as hypothesis-generating only, recommending parallel single-agent arms to prevent conflating ERR-mediated transcriptional changes with NNMT-driven NAD+/SAM modulation. Researchers interested in related mitochondrial peptide mechanisms can also consult work on SS-31 mechanism and research applications for comparative pathway context.


Designing Assays That Cleanly Separate NNMT-Related Readouts From MOTS-c and SLU-PP-332 Effects

Designing Assays That Cleanly Separate NNMT-Related Readouts From MOTS-c and SLU-PP-332 Effects

Translating mechanistic knowledge into clean experimental design requires structured factorial layouts and pathway-anchored biomarker panels. The following framework reflects current best practices for 5-Amino-1MQ research assays where NNMT-related readouts must be separated from MOTS-c and SLU-PP-332 effects.

Experimental Architecture

A robust multi-agent study should include:

  1. Vehicle control arm, baseline for all endpoints
  2. 5-Amino-1MQ single-agent arm, isolates NNMT inhibition effects
  3. MOTS-c single-agent arm, isolates AMPK/one-carbon effects
  4. SLU-PP-332 single-agent arm, isolates ERR transcriptional effects
  5. Combination arms, factorial pairings and full triple combination

This structure allows statistical attribution of any observed change to a specific mechanism rather than the combination as a whole.

Biomarker Panel Assignment

Compound Primary Readout Category Key Markers
5-Amino-1MQ Enzymology / Metabolomics NNMT activity, 1-MNA, NAD+, SAM/SAH
MOTS-c Phosphoproteomics / Signaling p-AMPK, p-ACC, folate intermediates
SLU-PP-332 Transcriptomics / Biogenesis ERR targets, PGC-1alpha, mtDNA copy number

Controlling for Confounders

Several metabolic outputs, oxygen consumption rate, ATP production, and fatty acid oxidation flux, can be influenced by all three agents through different upstream routes. These shared endpoints should be treated as secondary, integrative readouts rather than attribution markers. Isotope tracing (e.g., 13C-labeled nicotinamide for NAD+ flux) provides the strongest evidence for NNMT-specific pathway engagement and cannot be mimicked by ERR agonism or AMPK activation.

All 5-Amino-1MQ work should be conducted with reagents carrying batch-specific certificates of analysis confirming purity at or above 99%, strictly within in vitro or ex vivo systems where exposure concentration and timing can be precisely controlled. This is consistent with the compound's current status as a research-only agent with no FDA-approved indication and no published human trials as of 2026. For parallel reading on rigorous preclinical peptide assay design, the overview of SS-31 10mg research peptide considerations offers useful methodological context.

A forward-looking note: Expert commentary in 2026 anticipates that the next major step for 5-Amino-1MQ will be formal GLP toxicology studies followed by early-phase human trials targeting obesity, fatty liver, or age-related muscle decline. Future multi-omic panels integrating metabolomics, phosphoproteomics, and transcriptomics will likely become the standard framework for dissecting NNMT versus ERR versus MOTS-c contributions in complex experimental designs. This remains speculative, pending formal study initiation.


Conclusion

Separating NNMT-related readouts from MOTS-c and SLU-PP-332 effects is not merely a technical preference, it is a prerequisite for interpretable data. The 5-Amino-1MQ research assays framework outlined here provides a practical roadmap: anchor NNMT attribution to enzyme activity, 1-MNA, and NAD+/SAM flux; assign AMPK phosphorylation and one-carbon intermediates to MOTS-c; and reserve ERR transcriptional signatures and mitochondrial biogenesis markers for SLU-PP-332.

Actionable next steps for researchers:

  • Build single-agent control arms into every multi-compound study before adding combination arms.
  • Use isotope-traced NAD+ salvage assays as the gold-standard NNMT-specific readout.
  • Treat oxygen consumption rate and ATP output as integrative, not attributive, endpoints.
  • Source 5-Amino-1MQ with verified COA documentation and maintain strict in vitro or ex vivo protocols.
  • Interpret all findings within the current preclinical-only evidence base, no human trial data exist as of 2026.

Rigorous pathway separation today will produce the mechanistic clarity needed for the human-trial assay panels that the field anticipates in the coming years.

https://www.puretestedpeptides.com/wp-content/uploads/2026/09/5-amino-1mq-research-assays-how-nnmt-related-readouts-can-be-separated-from-mots.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-09-25 13:09:272026-09-25 13:09:275-Amino-1MQ Research Assays: How NNMT-Related Readouts Can Be Separated From MOTS-c and SLU-PP-332 Effects
Slupp332 With 5-Amino-1MQ: How Researchers Frame This Metabolic Stack

Slupp332 With 5-Amino-1MQ: How Researchers Frame This Metabolic Stack

September 22, 2026/0 Comments/in Uncategorized/by

Fewer than a dozen published preclinical studies exist on SLU-PP-332, yet by 2026 it has already become one of the most discussed compounds in advanced metabolic research circles, almost always alongside 5-Amino-1MQ. The pairing is not accidental. Researchers who study energy regulation have begun framing Slupp332 with 5-Amino-1MQ: how researchers frame this metabolic stack as a mechanistically logical combination, one where two distinct enzyme targets converge on a shared outcome: improved mitochondrial efficiency and NAD+ availability. This article unpacks that framing, explains the underlying study logic, and clarifies what the current evidence actually supports.
Key Takeaways

  • SLU-PP-332 activates estrogen-related receptors (ERRs), mimicking the gene-expression signature of aerobic exercise in preclinical models.
  • 5-Amino-1MQ inhibits the NNMT enzyme, preserving the SAM cycle and elevating intracellular NAD+ levels.
  • Researchers frame the stack as complementary because the two compounds target different upstream nodes of the same metabolic pathway.
  • Both compounds remain strictly preclinical and research-only as of 2026, with no completed human clinical trials.
  • A tri-compound extension adding MOTS-c is increasingly discussed as a "metabolic trifecta" in analyst commentary, though evidence remains early-stage.

What SLU-PP-332 and 5-Amino-1MQ Each Do Individually

What SLU-PP-332 and 5-Amino-1MQ Each Do Individually

Understanding the stack begins with understanding each compound in isolation.

SLU-PP-332 is a small-molecule agonist that activates the estrogen-related receptor (ERR) family, specifically ERRalpha, ERRbeta, and ERRgamma. These nuclear receptors regulate genes involved in mitochondrial biogenesis, fatty acid oxidation, and oxidative phosphorylation. In rodent models, SLU-PP-332 administration produced measurable increases in endurance capacity and activated a gene-expression profile that closely resembles the cellular response to sustained aerobic exercise. This is why researchers frequently describe it using the term "exercise mimetic," though that label carries important caveats: the downstream metabolic effects observed in animal tissue do not automatically translate to human physiology.

5-Amino-1MQ works through a completely different mechanism. It is a selective inhibitor of nicotinamide N-methyltransferase (NNMT), an enzyme highly expressed in adipose tissue and the liver. When NNMT is active, it consumes S-adenosylmethionine (SAM) and converts nicotinamide into a methylated byproduct that exits the NAD+ biosynthesis cycle. By blocking NNMT, 5-Amino-1MQ preserves both the SAM pool and the nicotinamide available for NAD+ resynthesis. The result, in preclinical models, is an elevation of intracellular NAD+, a coenzyme central to energy metabolism, sirtuin activation, and mitochondrial repair signaling. Researchers interested in 5-Amino-1MQ and related NAD+ modulators often pair it with compounds that act downstream of NAD+ availability.
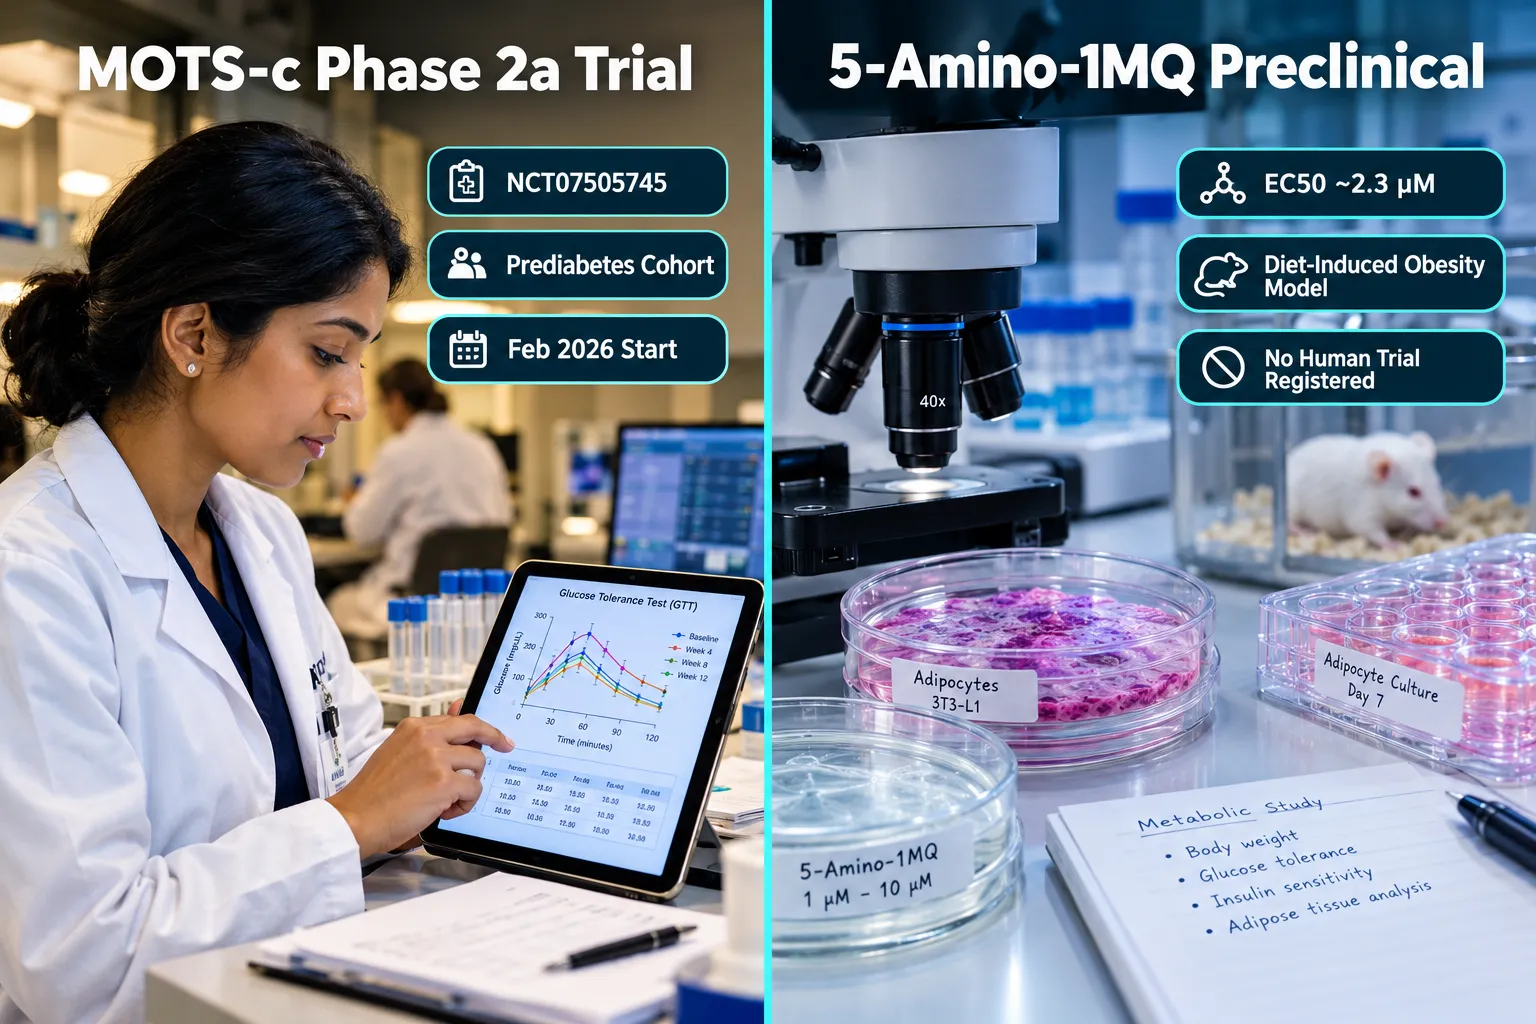

The Research Logic Behind Slupp332 With 5-Amino-1MQ: How Researchers Frame This Metabolic Stack

The Research Logic Behind Slupp332 With 5-Amino-1MQ: How Researchers Frame This Metabolic Stack

The core argument researchers make for combining these two compounds is mechanistic complementarity, not additive redundancy.

SLU-PP-332 drives the demand side of mitochondrial metabolism: it signals cells to build more mitochondria and upregulate oxidative pathways. 5-Amino-1MQ addresses the supply side: it ensures that the NAD+ substrate required to fuel those pathways is more readily available. In that framing, the stack functions like simultaneously upgrading both an engine and its fuel supply.

"The appeal of this combination is that it targets two separate rate-limiting steps in the same metabolic cascade, ERR activation and NAD+ substrate availability, without obvious mechanistic overlap."

This logic has appeared in commercial research bundle descriptions, analyst newsletters, and preclinical study design discussions throughout 2025 and 2026. It is worth noting, however, that no published study has directly tested this combination in a controlled animal model, let alone in humans. The synergy argument remains inferential, built from the individual compound literatures rather than direct co-administration data.

The Tri-Compound Extension: Adding MOTS-c

A growing subset of researchers extends the stack further by adding MOTS-c, a mitochondria-derived peptide that activates AMPK and influences glucose uptake in skeletal muscle. This three-way framing, SLU-PP-332 for ERR activation, 5-Amino-1MQ for NAD+ preservation, and MOTS-c for AMPK-mediated glucose handling, is sometimes called a "metabolic trifecta" in analyst commentary. Those interested in the broader mitochondrial peptide landscape can explore SS-31 mitochondrial research themes and SS-31 mitochondrial dynamics for adjacent mechanistic context, since mitochondrial-targeting compounds share several overlapping research questions.


Regulatory Status, Safety Framing, and 2026 Market Presentation

Regulatory Status, Safety Framing, and 2026 Market Presentation

Both SLU-PP-332 and 5-Amino-1MQ are classified strictly as research chemicals. As of 2026, neither compound has completed Phase I human clinical trials. They are not approved drugs, not dietary supplements, and not intended for human consumption. Expert commentary consistently emphasizes this classification, even as commercial interest has grown.

The 2026 market landscape shows these compounds increasingly available in capsule and tablet formats from research suppliers, often accompanied by third-party purity certificates. Suppliers emphasize lab-tested peptides and research compounds as a quality differentiator, and certificate-of-analysis documentation has become a standard expectation among serious researchers. That said, purity claims vary significantly across vendors, and researchers are advised to verify independent testing before use in any study context.

Key safety framing points from 2026 guidance:

  • No human dose-response data exists for either compound.
  • Rodent studies used weight-adjusted doses that do not directly translate to human equivalents.
  • Long-term toxicity profiles remain unknown for both compounds.
  • Stacking introduces additional complexity because interaction effects have not been studied.
  • Regulatory bodies in most jurisdictions have not issued specific guidance on these compounds, leaving their legal status ambiguous outside of research use.

Researchers interested in other metabolic compounds with more established preclinical profiles, such as those exploring SIRT1-related pathways or SS-31 elamipretide, will find that the evidence base for those compounds is comparatively more developed, which provides a useful benchmark for evaluating where SLU-PP-332 and 5-Amino-1MQ currently stand.

How Stacking Protocols Are Currently Described

Research protocol discussions in 2026 typically describe the following framing parameters, presented here strictly as reported research context, not as dosing recommendations:

Parameter SLU-PP-332 (Reported Range) 5-Amino-1MQ (Reported Range)
Administration route Oral (capsule) Oral (capsule)
Cycle length discussed 4-8 weeks 4-8 weeks
Primary research endpoint ERR activation markers NAD+ metabolite levels
Evidence tier Rodent preclinical only Rodent preclinical only

These figures reflect how researchers describe their protocols in published commentary, not clinically validated parameters.


Conclusion

The framing of Slupp332 with 5-Amino-1MQ: how researchers frame this metabolic stack is built on a coherent mechanistic argument, two compounds targeting distinct but complementary nodes in mitochondrial energy regulation. SLU-PP-332 drives ERR-mediated mitochondrial biogenesis from the demand side; 5-Amino-1MQ preserves NAD+ substrate availability from the supply side. The tri-compound extension with MOTS-c adds a third layer targeting AMPK and glucose handling.

That logic is intellectually compelling, but the evidence base remains firmly preclinical. No human trials have validated the combination, and safety data is limited.

Actionable next steps for researchers:

  1. Review the individual compound literatures separately before evaluating stack claims.
  2. Prioritize vendors that provide independent third-party purity documentation.
  3. Treat any synergy claims as hypothesis-generating rather than evidence-confirmed.
  4. Monitor peer-reviewed preprint servers for emerging co-administration studies, which remain the missing link in this research narrative.
  5. Consult regulatory guidance in your jurisdiction before designing any study involving these compounds.

The study logic is sound enough to warrant serious research attention. The evidence, as of 2026, has not yet caught up with the framing.

https://www.puretestedpeptides.com/wp-content/uploads/2026/09/slupp332-with-5-amino-1mq-how-researchers-frame-this-metabolic-stack.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-09-22 13:04:382026-09-22 13:04:38Slupp332 With 5-Amino-1MQ: How Researchers Frame This Metabolic Stack
Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models

Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models

September 21, 2026/0 Comments/in Uncategorized/by

Creatine monohydrate has more randomized controlled trial data behind it than almost any other supplement in sports science, yet two mitochondrial-pathway agents, MOTS-c and 5-amino-1MQ, are generating significant research interest in 2026. Understanding what separates these three compounds requires looking at where they act, what evidence supports them, and why comparing phosphagen energy buffering with mitochondrial peptide signaling is not as straightforward as it might seem. This article breaks down the science of Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models so researchers and informed readers can evaluate each agent on its actual merits.

Key Takeaways

  • Creatine monohydrate directly boosts intramuscular phosphocreatine, with decades of human RCT data confirming benefits for high-intensity performance.
  • MOTS-c is a mitochondrial-derived peptide currently in a Phase 2a prediabetes trial (NCT07505745, started February 2026); no completed human efficacy data exist for muscle or performance endpoints.
  • 5-Amino-1MQ is a small-molecule NNMT inhibitor with promising preclinical metabolic data but zero registered or published human clinical trials as of mid-2026.
  • All three compounds act through fundamentally different biological pathways, phosphagen buffering versus mitochondrial/NAD-linked metabolic signaling.
  • MOTS-c and 5-amino-1MQ should be regarded as experimental research tools, not practical replacements for creatine in muscle energy models.

The Phosphagen System: How Creatine Works in Muscle Cells

The Phosphagen System: How Creatine Works in Muscle Cells

Creatine's mechanism is well-defined and directly tied to the phosphagen energy system. When a muscle fiber contracts at high intensity, ATP is consumed faster than oxidative phosphorylation can replenish it. Phosphocreatine (PCr) stored in the cytoplasm donates a phosphate group to ADP via the creatine kinase enzyme, rapidly regenerating ATP. Supplementing with creatine monohydrate increases the intramuscular PCr reservoir, extending the window of high-power output before fatigue sets in.

This is not a theoretical model. Human skeletal muscle biopsy studies and in vitro myotube experiments have consistently shown that elevated creatine loading increases PCr content, improves repeated-sprint performance, and supports resistance-training adaptations including lean mass gains. Creatine is a dietary supplement available without prescription, and its safety profile in healthy adults is well-established across multiple decades of research.

Key phosphagen-system facts:

Feature Detail
Primary target Intramuscular phosphocreatine pool
Energy system Phosphagen (immediate ATP resynthesis)
Evidence level Multiple human RCTs, meta-analyses
Regulatory status Dietary supplement (no prescription needed)
Muscle model data Extensive in vitro myotube and in vivo human data

MOTS-c and 5-Amino-1MQ: Mitochondrial Peptide Pathways Explained

MOTS-c and 5-Amino-1MQ: Mitochondrial Peptide Pathways Explained

MOTS-c and 5-amino-1MQ operate through entirely different biological machinery. Neither targets the phosphagen system directly. Instead, both influence mitochondrial and NAD-linked metabolic pathways that affect systemic energy metabolism, insulin sensitivity, and adiposity.

MOTS-c: A Mitochondrial-Derived Peptide

MOTS-c is encoded within the mitochondrial genome and functions as a signaling peptide that activates AMPK and modulates metabolic stress responses. In preclinical models, it has been shown to improve insulin sensitivity, reduce fat accumulation, and support mitochondrial function. A CB4211 analogue of MOTS-c demonstrated reductions in liver enzymes (roughly 21% for ALT and 28% for AST) in overweight adults with non-alcoholic fatty liver disease, but those studies were small, short, and included no exercise-performance endpoints.

As of 2026, the most significant clinical development is a randomized, double-blind, placebo-controlled Phase 2a trial (NCT07505745) enrolling approximately 120 adults with prediabetes and overweight/obesity. The trial began in February 2026 and focuses on insulin sensitivity via oral glucose tolerance testing, HbA1c, and safety. No results have been posted. Researchers interested in MOTS-c peptide research materials can explore available options, though all use remains strictly preclinical.

5-Amino-1MQ: An NNMT Inhibitor

5-Amino-1MQ inhibits nicotinamide N-methyltransferase (NNMT), an enzyme that consumes methyl groups and suppresses NAD-dependent metabolic flux. In differentiated adipocytes, it shows an EC50 of approximately 2.3 µM with a well-fitted sigmoidal dose-response curve. In diet-induced obese mice, NNMT inhibition increased NAD-linked metabolic activity, reduced weight gain, and improved glucose handling.

"No human clinical trial of 5-amino-1MQ has been published or registered as of mid-2026. All available evidence is classified as preclinical only."

There is no FDA-approved indication, no publicly documented Investigational New Drug application, and no completed Phase 1 safety data for 5-amino-1MQ in humans. Expert commentary in 2026 consistently classifies any claims about human fat loss, muscle gain, or longevity as speculative extrapolations from animal and cell-culture data.

Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models

Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models

When evaluating Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models, the most important distinction is the type of muscle model each compound has actually been tested in.

Creatine has extensive dedicated skeletal-muscle data, myotube cultures, human biopsy studies, and exercise trials measuring fatigue resistance and hypertrophy. MOTS-c and 5-amino-1MQ data come primarily from systemic metabolic models: rodent obesity studies, adipocyte cultures, and hepatic cell lines. Neither has been tested as a direct substitute for creatine in phosphagen-system or muscle-performance models.

Side-by-side pathway comparison:

Compound Primary Pathway Muscle Model Evidence Human Trial Status
Creatine Phosphagen (PCr/ATP buffering) Extensive myotube and human RCT data Decades of completed trials
MOTS-c Mitochondrial peptide / AMPK signaling Systemic metabolic and adipocyte models Phase 2a ongoing (metabolic endpoints)
5-Amino-1MQ NNMT inhibition / NAD+ flux Adipocyte and rodent obesity models No registered human trial

Researchers exploring mitochondrial-targeted compounds alongside creatine may also find value in reviewing SS-31 peptide research considerations, as SS-31 represents another mitochondria-focused peptide with a distinct cardiolipin-binding mechanism. The SS-31 peptide category offers additional context for comparing mitochondrial-targeting agents.

If MOTS-c or 5-amino-1MQ were eventually shown to improve mitochondrial efficiency and body composition in humans, experts suggest they might serve as adjuncts to established interventions, diet, exercise, and creatine, rather than replacements. The MOTS-c Phase 2a trial targets primary completion in February 2027, with final completion around May 2028. Any muscle-specific or performance-oriented trials would likely follow only after convincing metabolic efficacy and safety data are available. For 5-amino-1MQ, near-term development would almost certainly focus on obesity and diabetes indications before any sports-performance application.

Those researching peptide purity and sourcing standards for experimental compounds can consult resources on evaluating research-grade peptide purity and compatibility for broader quality-assessment frameworks. For context on how peptides interact with endocrine and receptor biology, the overview of peptides and polypeptides in endocrine pharmacology provides useful mechanistic background.

Conclusion

The comparison of Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models reveals a clear evidence hierarchy. Creatine remains the only compound of the three with robust, reproducible human data for high-intensity exercise performance, supported by direct skeletal-muscle research. MOTS-c is a promising mitochondrial-derived peptide now entering Phase 2a human testing for metabolic endpoints, not muscle performance. 5-Amino-1MQ is a potent preclinical NNMT inhibitor with no human trial data at all.

Actionable next steps for researchers:

  • Treat creatine as the established reference point for phosphagen-system support in any muscle cell model comparison.
  • Monitor NCT07505745 for MOTS-c Phase 2a results expected in early-to-mid 2027 before drawing conclusions about metabolic efficacy.
  • Classify 5-amino-1MQ strictly as a preclinical tool; do not extrapolate adipocyte or rodent findings to human muscle performance without registered trial data.
  • When designing comparative in vitro studies, distinguish clearly between ATP-buffering endpoints (relevant to creatine) and mitochondrial signaling or NAD-flux endpoints (relevant to MOTS-c and 5-amino-1MQ).
  • Source all research-grade peptides from suppliers with verified third-party purity testing to maintain experimental integrity.
https://www.puretestedpeptides.com/wp-content/uploads/2026/09/creatine-supplementation-vs-mots-c-and-5-amino-1mq-comparing-phosphagen-and-mito.webp 1024 1536 https://www.puretestedpeptides.com/wp-content/uploads/2026/01/buy-peptides-online.jpg 2026-09-21 13:36:052026-09-21 13:36:05Creatine Supplementation vs MOTS-c and 5-Amino-1MQ: Comparing Phosphagen and Mitochondrial Peptide Pathways in Muscle Cell Models
Page 1 of 3123
×

Helpful Links

  • My account
  • Cart
  • Checkout
  • Refund and Returns Policy
  • Privacy Policy
  • SMS Privacy Policy
  • Login
  • My Account
  • Logout

USA Made Lab Tested Peptides

All products are sold for research, laboratory, or analytical purposes only, and are not for human consumption


Pure Tested Peptides is a chemical supplier. Pure Tested Peptides is not a compounding / chemical compounding facility as defined under 503A of the Federal Food, Drug, and Cosmetic act. Pure Tested Peptides is not an outsourcing facility as defined under 503B of the Federal Food, Drug, and Cosmetic act.

The statements made within this website have not been evaluated by the US Food and Drug Administration. The products we offer are not intended to diagnose, treat, cure or prevent any disease.

Human/Animal Consumption Prohibited. Laboratory/In-Vitro Experimental Use Only

Scroll to top Scroll to top Scroll to top